Understanding the 9:3:3:1 Pattern Without the Fluff
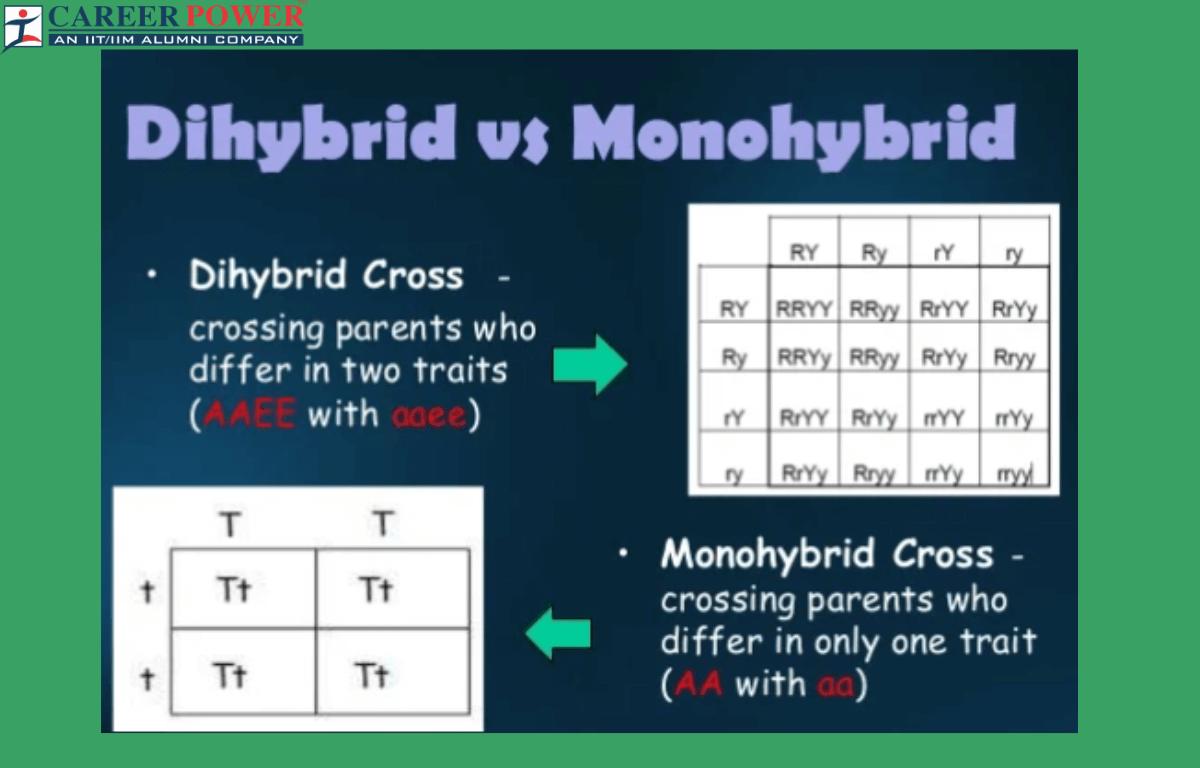
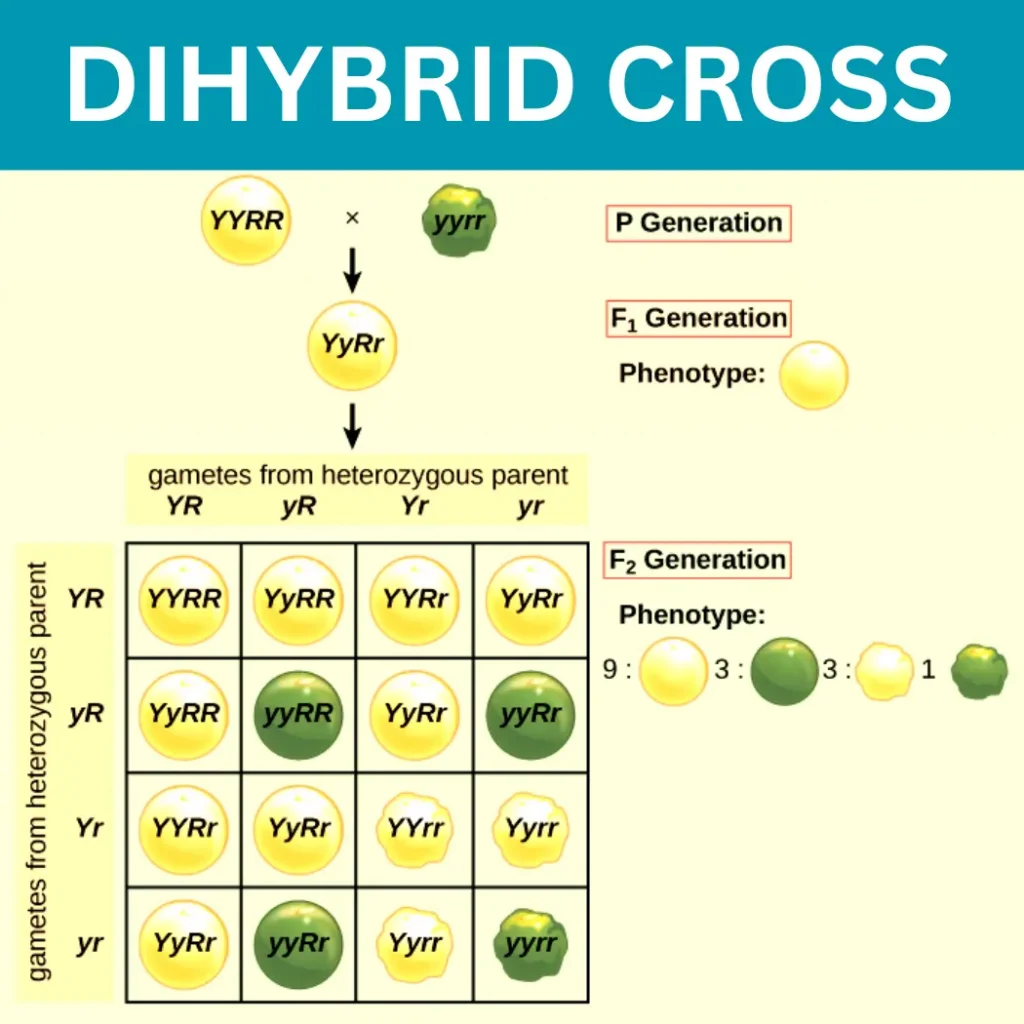
Most genetics classes spend two lectures on Punnett squares before you ever touch real data. I spent a semester trying to figure out why my pea plants weren't following the textbook ratios, and it wasn't because I couldn't do the math. It was because I didn't understand what the dihybrid cross actually assumes about how genes behave. A dihybrid cross tracks two different traits at the same time, not one after the other. You watch seed color and seed shape together in peas, or wing length and body color in fruit flies. The standard approach is to cross two individuals that are heterozygous for both traits, and then look at the phenotypes in the F2 generation. If the genes assort independently, you get that classic 9:3:3:1 ratio. Nine with both dominant traits, three with the first dominant and second recessive, three with the reverse, and one with both recessive.
What Is A Dihybrid Cross in Practice
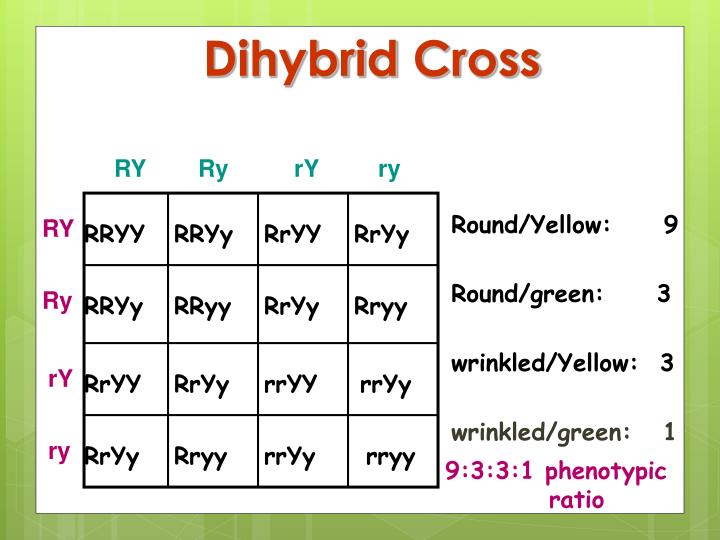
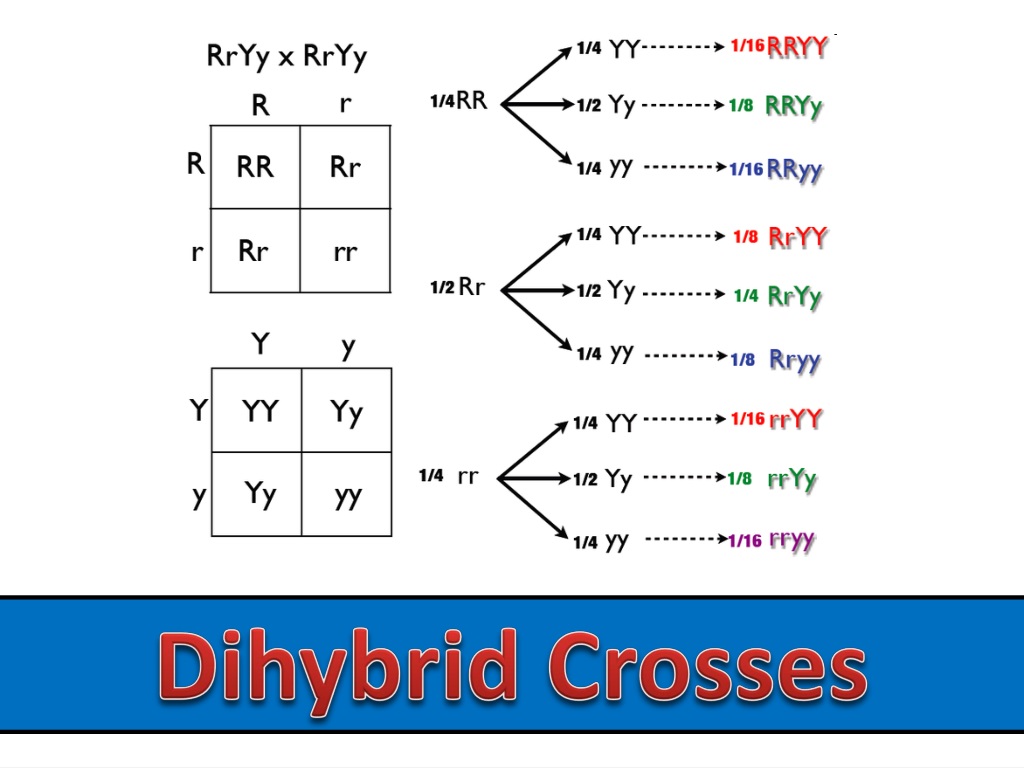
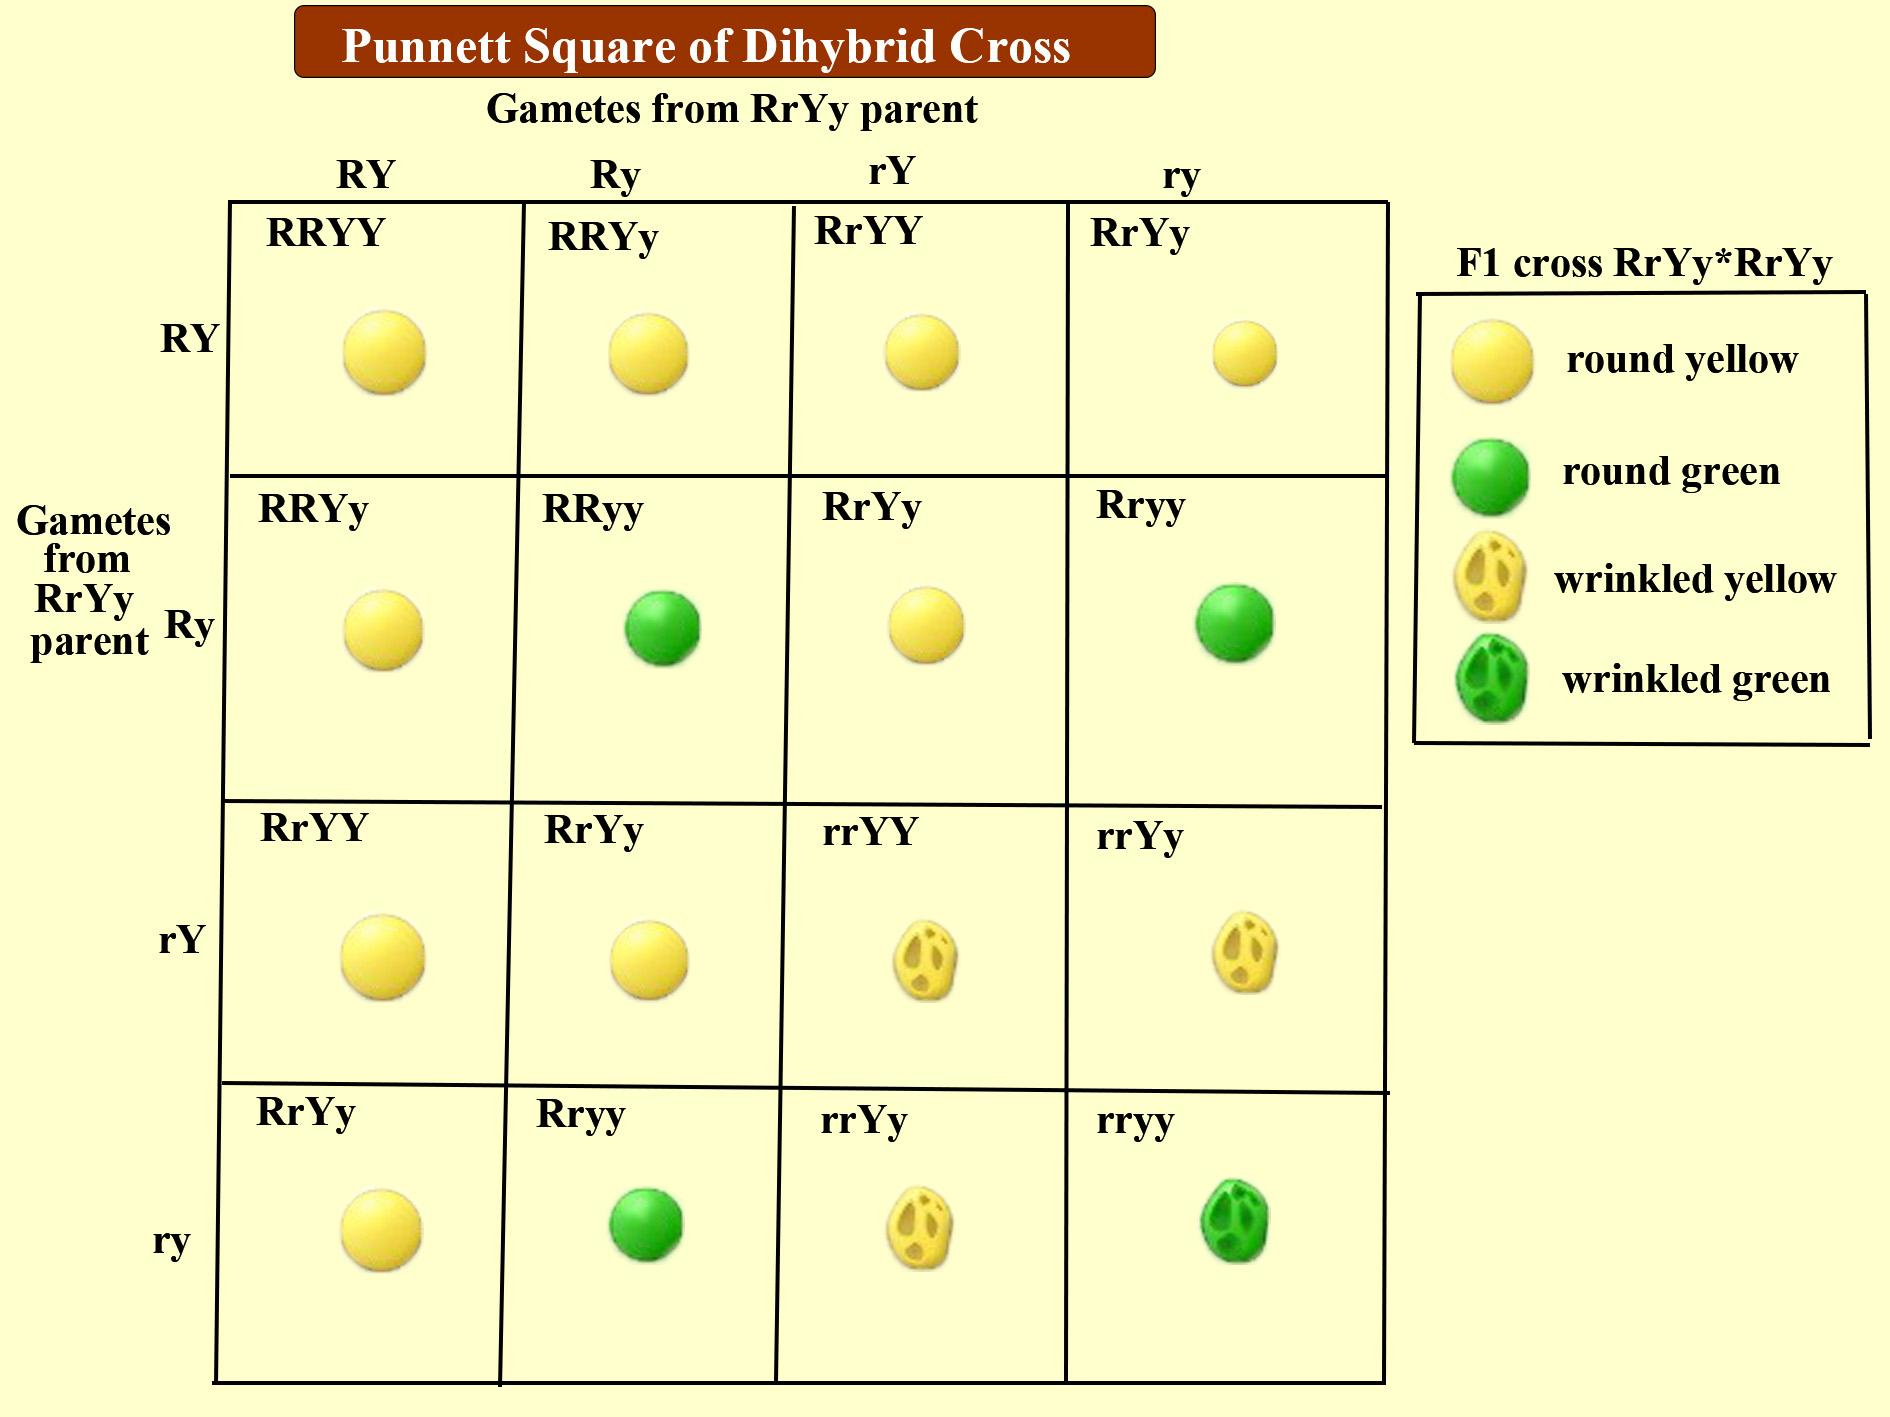
The actual work starts with writing out the parental genotypes. Say you cross true-breeding round yellow seeds with true-breeding wrinkled green seeds. The F1 generation is all heterozygous round yellow, which tells you round dominates wrinkled and yellow dominates green. Then you self-cross the F1, and you get sixteen possible combinations in the F2. That is where the 9:3:3:1 comes from, but only if the genes are on different chromosomes or far enough apart on the same chromosome. I ran into a real problem last year when I was working with a custom Drosophila cross. I expected independent assortment between two markers, but the ratios were completely off. After checking the map, I found the genes were less than five map units apart. The F2 ratio came out closer to 13:3:1 than 9:3:3:1 because recombination was happening but not at the 50 percent frequency that independent assortment requires. I had to calculate the actual recombination frequency from the data instead of assuming the textbook ratio would hold. The method itself is straightforward. You write the gametes each parent can produce. For a double heterozygote like RrYy, that is four gamete types: RY, Ry, rY, ry. Each gets a 25 percent chance if the genes are unlinked. Then you set up a 4x4 Punnett square with sixteen boxes, and you fill in the genotypes by combining the gametes from each parent. Finally, you group the phenotypes into the four categories and count them up.
But here is the part nobody tells you in the intro class. The 9:3:3:1 ratio is a phenotypic ratio, not a genotypic ratio. The genotypes are way more complicated. You get nine different genotypes in the F2, not four. If you count them properly, you find 1 RRYY, 2 RRYy, 2 RrYY, 4 RrYy, 1 RRyy, 2 Rryy, 1 rrYY, 2 rrYy, and 1 rryy. The phenotypes collapse these into four groups, which is why the ratio looks cleaner than it actually is. Another thing that trips people up is incomplete dominance and codominance. If either trait shows incomplete dominance instead of complete dominance, the ratio changes completely. Say red and white flowers show incomplete dominance, so heterozygotes are pink. Cross two pink flowers and you get 1 red:2 pink:1 white for that single trait. Do the same for two traits with incomplete dominance and you get a 1:2:1 ratio for each, which multiplies out to a 9:3:3:1 equivalent but with nine distinct phenotypes instead of four. The math is the same, but the phenotypic classes are different. Epistasis is another common complication. The classic example is coat color in labs, where one gene controls pigment production and another controls pigment deposition. If the deposition gene is homozygous recessive, the lab is yellow regardless of what the pigment gene says. In that case, the dihybrid cross gives a 9:3:4 ratio instead of 9:3:3:1. You can still use the same method, but you have to recognize when epistasis is hiding behind the numbers.
Get the Full Details
The biggest bottleneck with dihybrid crosses is sample size. You need enough offspring to see the ratio clearly. With peas, you can grow thousands of seeds, so the ratios usually match expectations pretty closely. With animals, you might only get twenty or thirty offspring per cross, and random chance can make the numbers look completely off even when the genes are assorting independently. I once saw a chicken cross where the observed ratio was 7:5:3:1 instead of 9:3:3:1, and the student in the lab thought the genes were linked. They weren't. It was just small sample size making the numbers wobble around the expected values. Statistical testing is the only way to know for sure. A chi-square test will tell you whether your observed numbers are close enough to the expected ratio to accept the null hypothesis of independent assortment. The calculation is simple: subtract the expected from the observed for each class, square the difference, divide by the expected, and add up the results. If the final number is less than the critical value for your degrees of freedom, you accept independent assortment. If it is greater, you reject it and look for linkage or some other explanation. I usually recommend starting with a monohybrid cross first if you are new to this. Get comfortable tracking one trait, understanding dominant and recessive relationships, and running a chi-square test. Then move to two traits. Going straight to dihybrid crosses without that foundation makes it easy to miss when something is actually wrong with your cross versus when the math is just showing you the complexity of real genetics.
There is also the issue of sex linkage. If one of the genes is on the X chromosome, the ratios are completely different between males and females. You cannot use the standard dihybrid cross method without accounting for the sex of each offspring. I once worked with a mouse cross where one trait was autosomal and the other was X-linked, and the F2 ratios looked nothing like 9:3:3:1 until I separated the data by sex. Males and females had different phenotype distributions because males only have one X chromosome and express whatever allele is on it, while females can be heterozygous. The workaround for sex-linked traits is to write out separate Punnett squares for each sex, or to include the sex chromosomes in your gamete notation. Instead of just RrYy, you write it as RrX^A X^a for a female or RrX^A Y for a male. Then the gametes are different depending on whether you are tracking the autosomal gene or the sex chromosome, and the ratios change accordingly. It is more work, but it is the only way to get the right answer. If you want to download a worksheet or practice problems, most university genetics courses post them online for free. Search for "dihybrid cross practice problems pdf" and you will find hundreds of examples with answers. The better ones include cases with linkage, epistasis, and sex linkage, not just the straightforward 9:3:3:1 scenario. Working through those variations will prepare you for real lab work better than any textbook diagram.
The key takeaway is that the dihybrid cross is a model, not a law. It works perfectly under ideal conditions with independent assortment, complete dominance, large sample sizes, and no epistasis or linkage. Real genetics is messier. The genes might be linked, the dominance might be incomplete, the sample size might be too small, or there might be epistatic interactions hiding in the data. The method still works as a starting point, but you have to know when to trust the ratio and when to dig deeper. I have seen students throw away perfectly good data because the observed ratio did not match 9:3:3:1 exactly, and then spend weeks looking for errors that were not there. Sometimes the genes are just linked. Sometimes there is epistasis. Sometimes it is small sample size. The ratio is a tool for understanding, not a strict rule that nature has to follow. Use it to generate hypotheses, then test those hypotheses with proper statistical methods and careful attention to the biological details.