The basics before we get into the weeds
Evolutionary theory describes how populations change over generations through mechanisms like natural selection, genetic drift, mutation, and gene flow. That is the textbook version. The real thing is messier. When you actually work with evolutionary models, you quickly realize that the framework is less a single theory and more a family of overlapping models that sometimes contradict each other depending on what population you are studying. I spent years running population genetics simulations and field work. The theory works beautifully for things like antibiotic resistance in bacteria or pesticide resistance in insects. Those are clean, rapid, high-selection-pressure cases. But try applying standard models to long-lived vertebrate populations with low reproduction rates, and the math starts to fall apart. The assumptions break down.
What Is A Evolutionary Theory
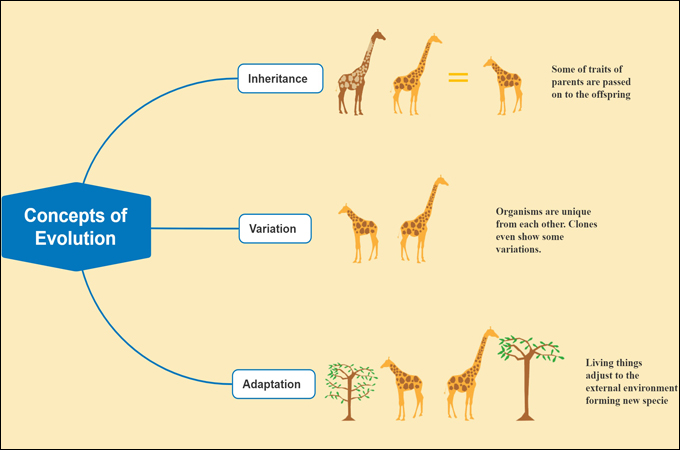
You need to understand that evolutionary theory in its modern form is the synthesis of Darwinian natural selection with Mendelian genetics, combined with population genetics mathematics. The core mechanism is differential reproductive success. Individuals with heritable traits better suited to their environment leave more offspring. Over time, those traits increase in frequency within the population. But here is the thing most beginners miss. Natural selection is not the only game in town. Genetic drift can overwhelm selection entirely in small populations. I once worked on a project with an endangered lizard species where we expected directional selection on a thermal tolerance trait. What we actually found was that drift was so strong in their tiny fragmented populations that selected alleles were being lost at random faster than selection could fix them. The standard adaptive narrative was completely wrong for that system.
How it actually works in practice
When you build an evolutionary model, you start with a population and define the fitness landscape. Fitness here means reproductive success relative to other genotypes. You assign selection coefficients to different alleles and track allele frequency changes across generations using equations like the Hardy-Weinberg principle as your baseline null model. The Hardy-Weinberg equilibrium tells you what happens when nothing evolutionary is occurring. Allele frequencies stay constant. If you see a deviation from H-W expectations in your data, something is happening. The trick is figuring out what. And that is where people make mistakes. They see a deviation and immediately assume selection. It could be inbreeding. It could be population structure. It could be genotyping error. I learned this the hard way on a plant population study. We saw what looked like strong selection on flowering time. The phenotype clearly deviated from the population mean, and the fitness gradient was steep. I spent three weeks writing up the results before a collaborator pointed out that we had missed a major weather event during the study period. The apparent selection was actually a demographic bottleneck. A drought killed half the population randomly with respect to the trait we were studying. What looked like evolution was just a population crash followed by regrowth. Correcting for the bottleneck shifted our estimated selection coefficient from 0.18 down to nearly zero.
Get the Full Details
The mechanics you need to know
There are four main forces. Mutation introduces new genetic variation. This is the raw material. Most mutations are neutral or deleterious. Only a tiny fraction are beneficial, and even fewer are fixed in a population. Natural selection increases the frequency of beneficial alleles and decreases harmful ones. The strength depends on the selection coefficient and the effective population size. In large populations, even weak selection can be effective. In small populations, drift dominates. Genetic drift is the random change in allele frequencies due to sampling error. Every generation, only a subset of individuals reproduce. By chance, some alleles may be overrepresented or underrepresented in the next generation. This effect is inversely proportional to effective population size. In populations below a few hundred individuals, drift can erase genetic variation faster than mutation can replace it.
Gene flow moves alleles between populations. Migration homogenizes genetic differences between groups. High gene flow can swamp local adaptation. If immigrants carry alleles maladapted to the local environment, selection has to work harder to maintain adaptation. There is a well-known threshold around Nm equals one, where m is the migration rate. Above that, gene flow prevents divergence. Below that, populations can differentiate.
Where the theory breaks down
One major limitation is the assumption of random mating. Real populations are rarely randomly mating. Assortative mating, inbreeding, and spatial structure all violate this assumption and change the dynamics significantly. When you ignore these factors, your predictions will be wrong. Another issue is epistasis. Most introductory treatments assume additive gene effects. Real genes interact. A mutation that is beneficial in one genetic background can be harmful in another. This context-dependence makes predicting evolutionary trajectories much harder. The fitness landscape is not smooth. It has peaks and valleys that shift depending on which alleles are already present. Then there is the problem of timescales. Evolutionary theory was developed largely for organisms with short generation times. Applying it to humans, elephants, or redwoods requires stretching the models in ways that sometimes do not hold. Generation time affects the rate of drift, the rate of mutation accumulation, and how quickly selection can respond. A model calibrated for fruit flies will overestimate the speed of evolutionary change in a slow-reproducing mammal.

I encountered a specific edge case with a tree species study where we were trying to predict adaptive response to climate change. The standard quantitative genetics approach uses the breeder's equation, R equals h squared times S, where R is the response to selection, h squared is narrow-sense heritability, and S is the selection differential. We measured heritability at 0.4 for growth rate and estimated the selection differential from climate data. The model predicted a certain rate of adaptation. In reality, the realized response was about thirty percent lower than predicted. The missing factor was a negative genetic correlation between growth rate and drought tolerance. Selection favoring faster growth was dragging along reduced drought tolerance. The multivariate breeder's equation handled this, but the univariate version did not. You have to measure the full G matrix, the genetic variance-covariance matrix, to get accurate predictions in these cases. And that requires either extensive pedigree data or genomic data from hundreds of individuals.
Common pitfalls to avoid
Do not confuse adaptation with optimality. Just because a trait exists does not mean it is optimal. It means it was sufficient for reproduction in past environments. Current environments may differ. organisms are often locally adapted, not globally optimized. Do not assume that genetic variation equals adaptive potential. Standing genetic variation may not contain the right alleles for future conditions. Adaptive evolution requires both variation and selection. If selection is weak or directional selection shifts faster than genetic variation can respond, populations can face extinction despite appearing genetically diverse. Do not overlook the role of non-adaptive processes. Not every trait is shaped by selection. Some traits are byproducts of selection on linked loci. Others are neutral. Genetic hitchhiking occurs when a neutral allele changes frequency because it is physically linked to a selected allele. Background selection removes neutral variation near deleterious mutations. These processes reduce genetic diversity in ways that look like selective sweeps but are not.
When building models, always check your assumptions. Test for Hardy-Weinberg equilibrium. Estimate effective population size. Consider whether drift, gene flow, or selection is likely dominating given your study system. Use simulation approaches like forward-time individual-based models when analytic solutions become intractable. Programs like SLiM or Nemo allow you to incorporate complex demographic histories, selection regimes, and recombination maps that traditional population genetics equations cannot handle. The field has moved toward combining theoretical models with empirical data from genomics. Whole-genome sequencing now lets us detect signatures of selection across the genome, identify selective sweeps, and estimate demographic parameters simultaneously. But the data alone do not tell you what is happening. You still need the theory to interpret patterns. A peak of differentiation between populations could reflect local adaptation or it could reflect a reduction in gene flow due to a geographic barrier. The pattern is the same. The interpretation depends on additional evidence.