Peptide Bonds And Why They Matter In Practice
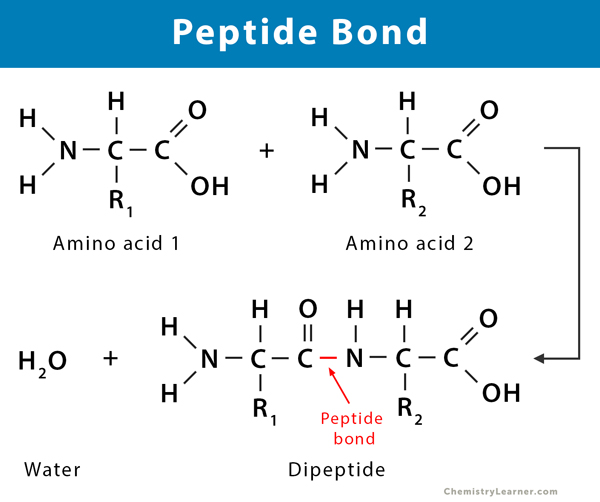
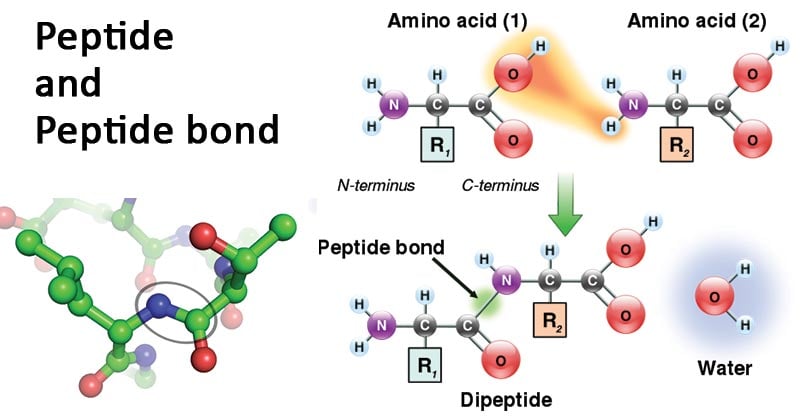
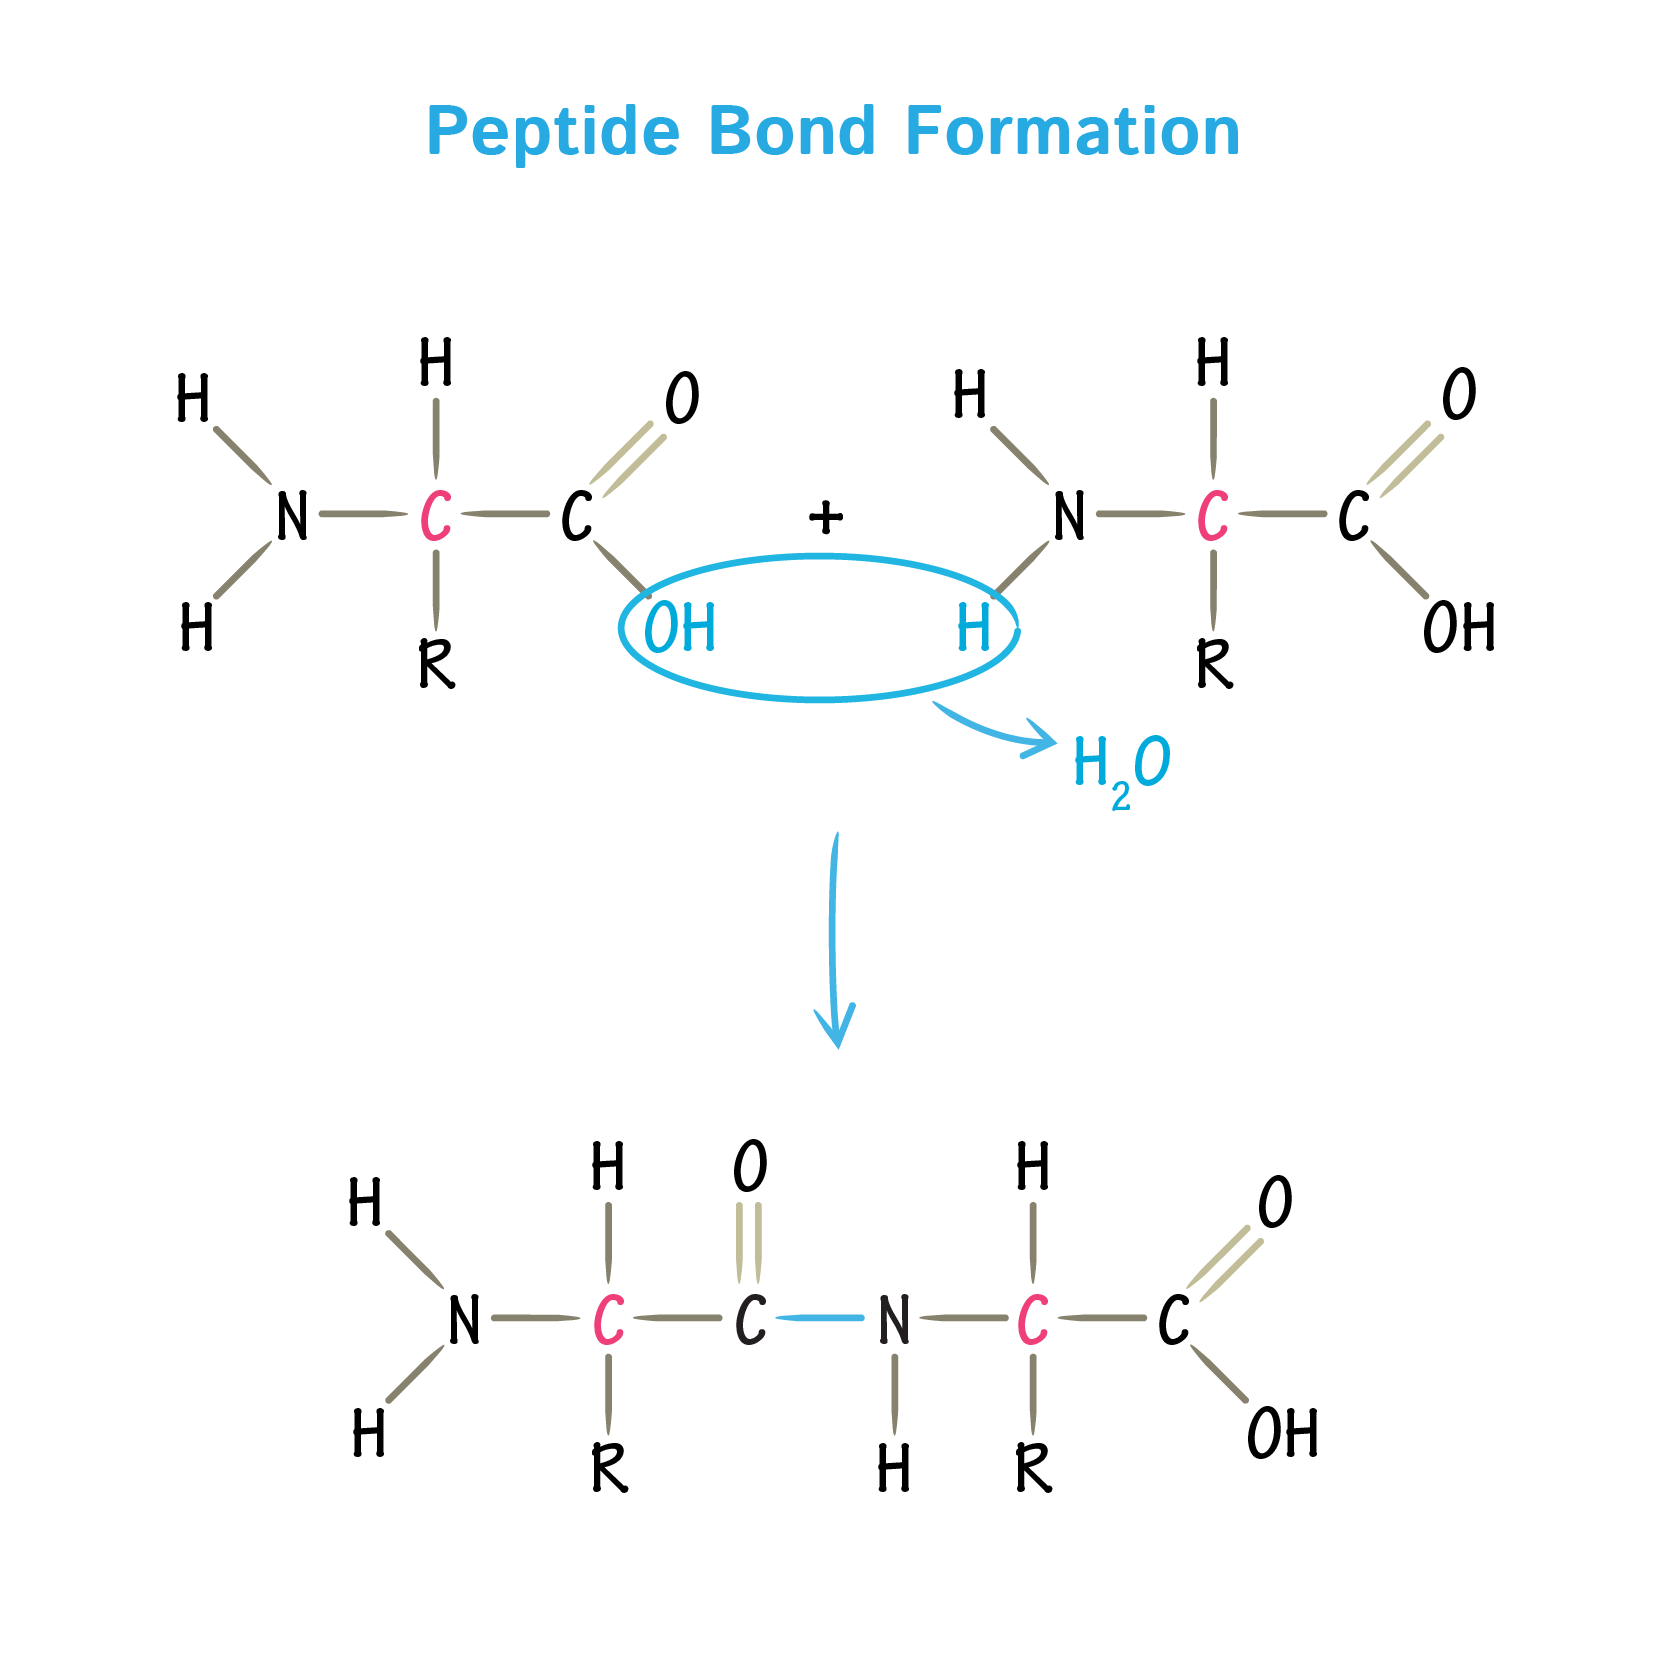
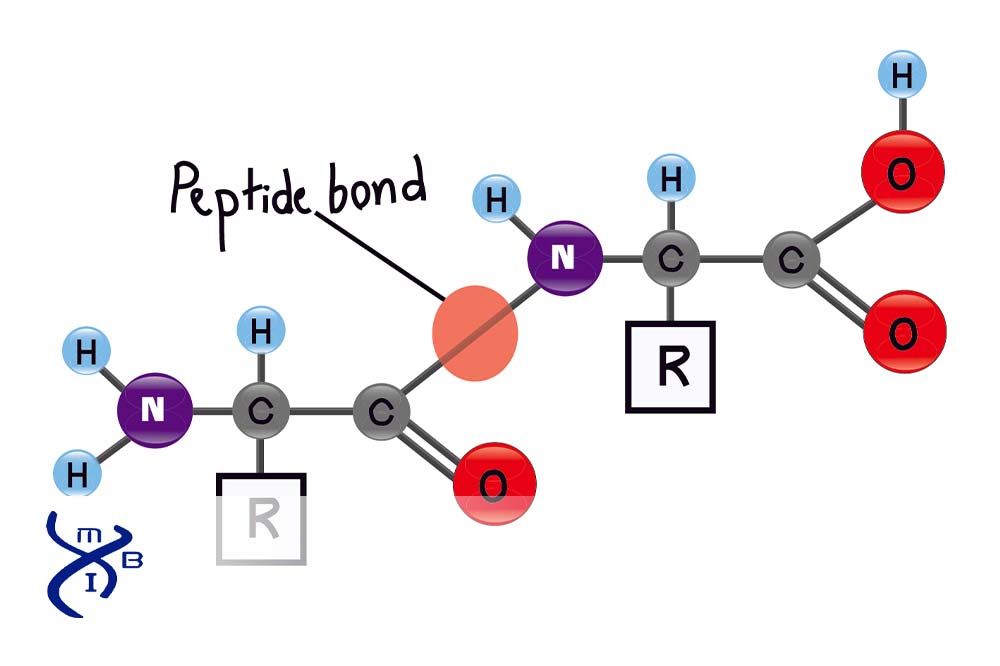
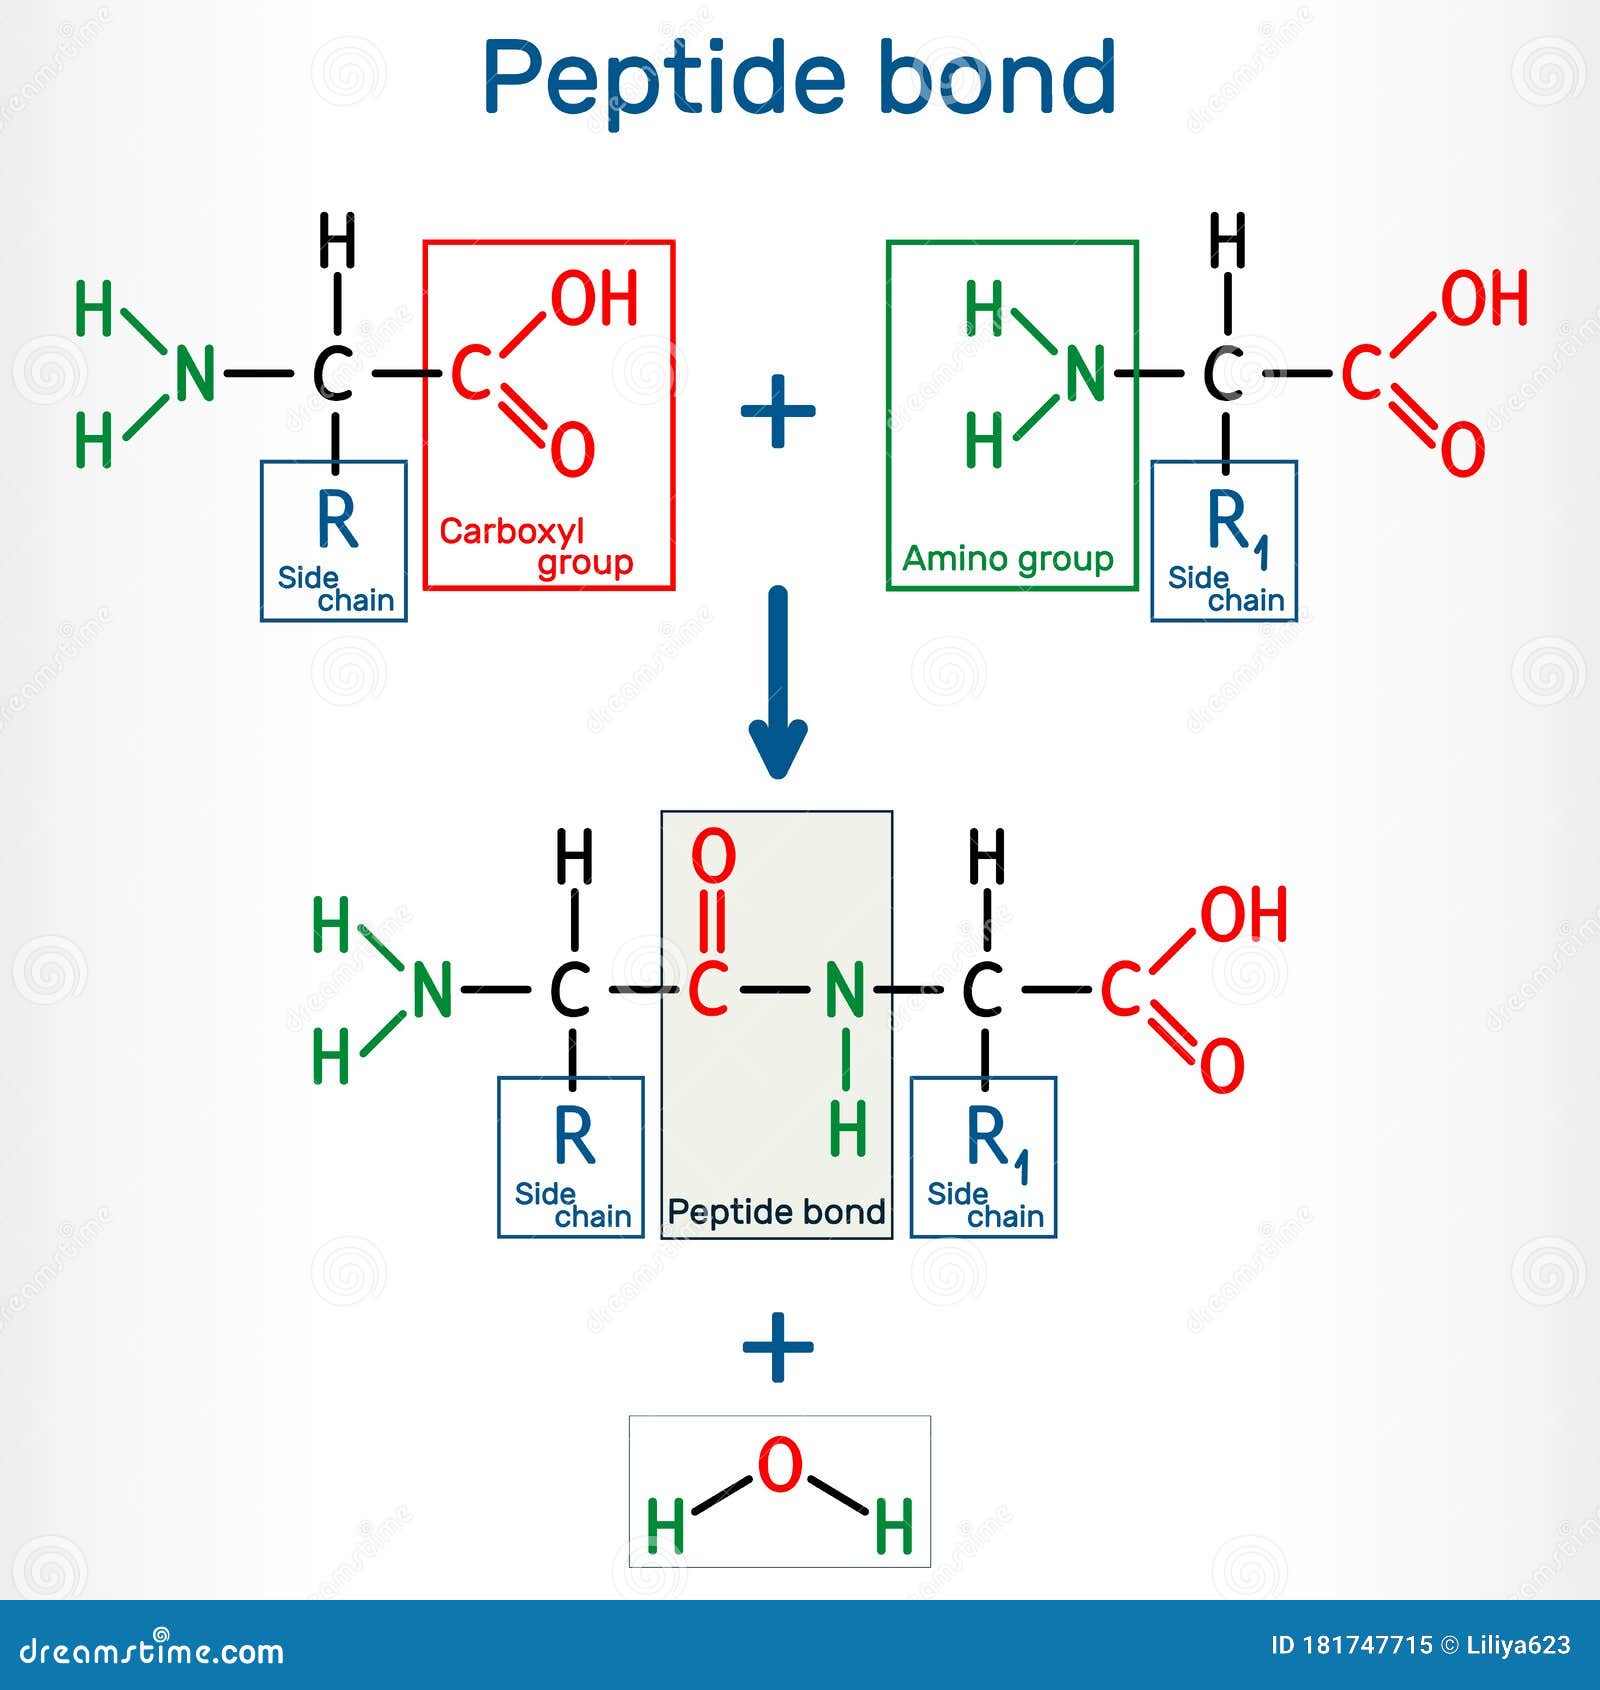
A peptide bond is a covalent chemical bond formed between the carboxyl group of one amino acid and the amino group of another, with the release of a water molecule. That is the textbook definition. The reality is messier and more interesting than that one sentence suggests. The bond itself is an amide linkage. Specifically, it forms between the carbonyl carbon of one residue and the nitrogen of the next. The resulting C-N bond has partial double-bond character because of resonance. This means the bond is planar and rigid. It does not freely rotate the way a typical single bond does. That rigidity shapes how proteins fold, and it matters a lot if you are trying to do anything beyond memorize the basic structure.
What Is A Peptide Bond From A Synthetic Chemist's Perspective
When you are actually making peptides in the lab, the peptide bond is not something that just appears. You have to activate the carboxyl group first. Normally you use a coupling reagent like HBTU, HATU, or DIC combined with an additive like HOBt or Oxyma. The activation step creates an ester intermediate that is much more reactive than the free carboxylic acid. Then the amine of the next amino acid attacks that activated carbon, and you get your peptide bond with the leaving group departing. I learned this the hard way early on. I was doing a solid-phase peptide synthesis run for a small hydrophobic sequence. I used standard Fmoc chemistry on Wang resin. The first three couplings went fine, then I hit a difficult residue. I had skipped adding the secondary amine additive to the coupling mix and just ran DIC alone. The coupling efficiency dropped to maybe forty percent. I could see it on the resin by the Kaiser test. Rather than try to push it harder with more reagent, which would just waste material, I switched to HATU with Oxyma and extended the coupling time to forty five minutes. That brought it back to around ninety five percent. Simple problem, but it cost me about four hours and some good peptide to figure out. One thing that catches people off guard is the directionality. Peptide synthesis always proceeds from the C-terminus to the N-terminus on the solid support. You attach the first amino acid through its carboxyl group and keep adding new residues to the growing N-terminus. If you mix that up even slightly, you end up with the wrong sequence. I have seen junior researchers lose days of work because they mislabeled a vial during the coupling steps.
Another nuance is racemization. When you activate the carboxyl group, there is a risk that the alpha carbon of that amino acid can invert its stereochemistry. This is especially problematic with cysteine and histidine because their side chains can participate in oxazolone formation. The older protocols using DCC had significant racemization issues. Modern reagents like HATU with Oxyma reduce this considerably, but it is not eliminated. If you are synthesizing a peptide with multiple Cys or His residues, you need to watch this. Running the coupling at lower temperature, around zero degrees Celsius, helps suppress racemization without killing the reaction rate too much. Also worth noting: the peptide bond is stable under physiological conditions but it is not unbreakable. Proteases cleave peptide bonds all the time in biological systems. In the lab, you can break them with strong acid hydrolysis, which is how you determine amino acid composition by breaking every peptide bond and then running the free amino acids through chromatography. Six molar HCl at one hundred ten degrees Celsius for twenty four hours will chew through almost everything. Some residues like tryptophan get destroyed in that process, so if you need to quantify tryptophan you have to use a different method like alkaline hydrolysis or direct sequencing. The partial double bond character also means that cis peptide bonds can form, though they are rare. Proline is the usual culprit here. In most cases the trans configuration is heavily favored, but with proline you can get a significant population of the cis form. This matters for protein folding kinetics because the cis to trans isomerization of a proline peptide bond can be the rate limiting step in folding. It is slow enough that chaperone proteins like cyclophilin exist specifically to catalyze that conversion. If you are doing structural biology or peptide design, ignoring this proline cis issue can lead to misleading results.
Get the Full Details

Mass spectrometry is where most people actually encounter peptide bonds in practice. When you run a peptide through tandem MS, the instrument fragments along the backbone at the peptide bonds. The fragment ions are called b ions and y ions depending on which side of the break retains the charge. Interpreting those spectra is how you sequence peptides. It is not always straightforward. You get internal fragments, neutral losses, and sometimes the bond just does not break where you expect it to. But understanding that the fragmentation happens at the peptide bond is the foundation of proteomics. If you are working with modified peptides or peptidomimetics, the peptide bond can be replaced with isosteric groups. A common example is the reverse amide bond where the NH and C=O are swapped. This can improve metabolic stability because proteases do not recognize the altered linkage as easily. I worked on a project where we substituted a few key peptide bonds with 1,3-disubstituted ureas. The compound was stable in serum for over twenty four hours compared to the native peptide which degraded in under fifteen minutes. The binding affinity dropped slightly but not catastrophically. Those kinds of modifications are standard in modern drug discovery programs targeting protein protein interactions. The takeaway is that peptide bonds are simple in definition but complex in execution. If you want to work with them effectively, you need to understand both the chemistry and the practical pitfalls. The resonance, the stereochemistry, the coupling strategies, the fragmentation patterns. All of it ties back to that one amide linkage between two amino acids.