Cell Membranes Are Not Passive Barriers
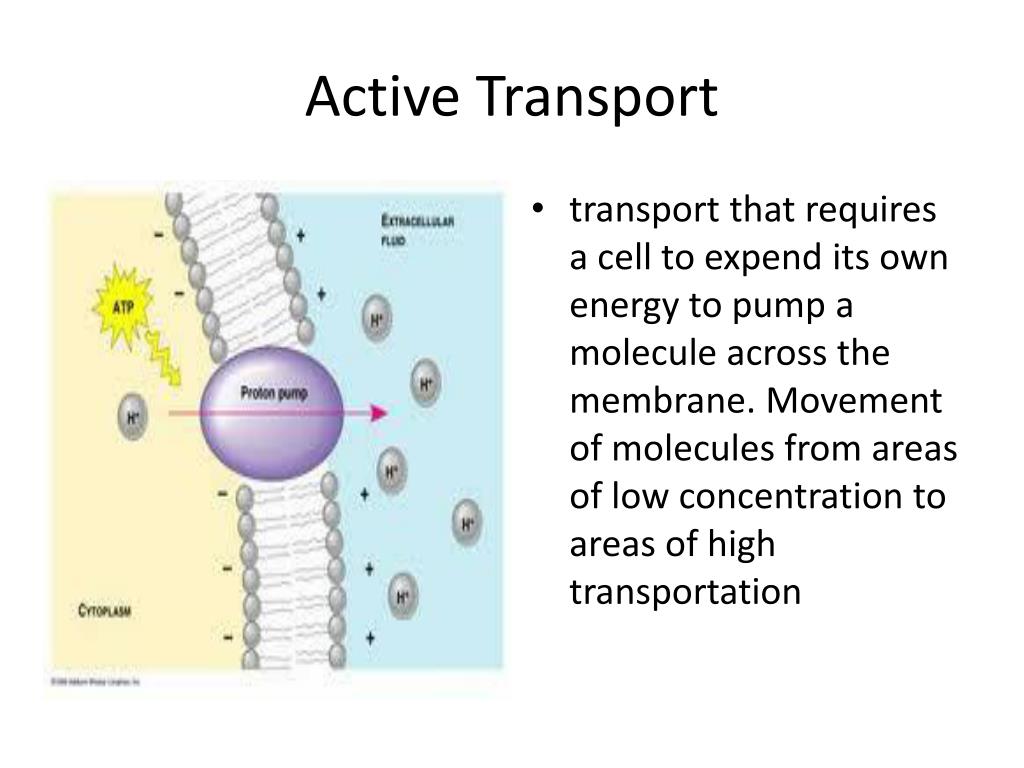
You probably learned about osmosis and diffusion in high school biology. Those processes move things from high concentration to low concentration. They require zero energy input. Active transport is the opposite. It moves substances against their concentration gradient, which means from low to high concentration, and it requires energy to do so. That energy almost always comes from ATP hydrolysis, but not always, and that distinction matters more than most textbooks let on. The sodium-potassium pump is the classic example. It sits in the membrane of nearly every animal cell and actively pumps three sodium ions out while pulling two potassium ions in. This establishes an electrochemical gradient that your nerves and muscles rely on to function. Without it, you'd be dead within minutes. But the pump isn't just about maintaining balance. It's about creating a state of organized disequilibrium, and that's a more expensive proposition than most people appreciate.
What Is Active Transport
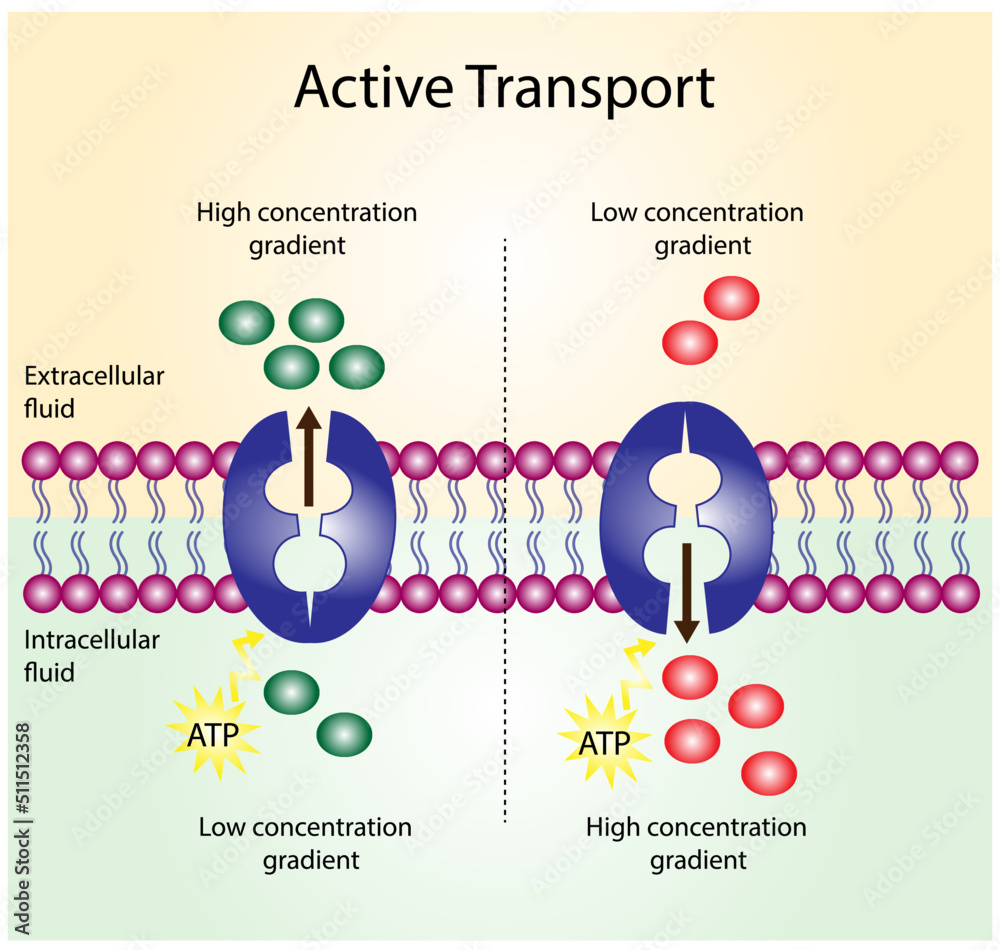
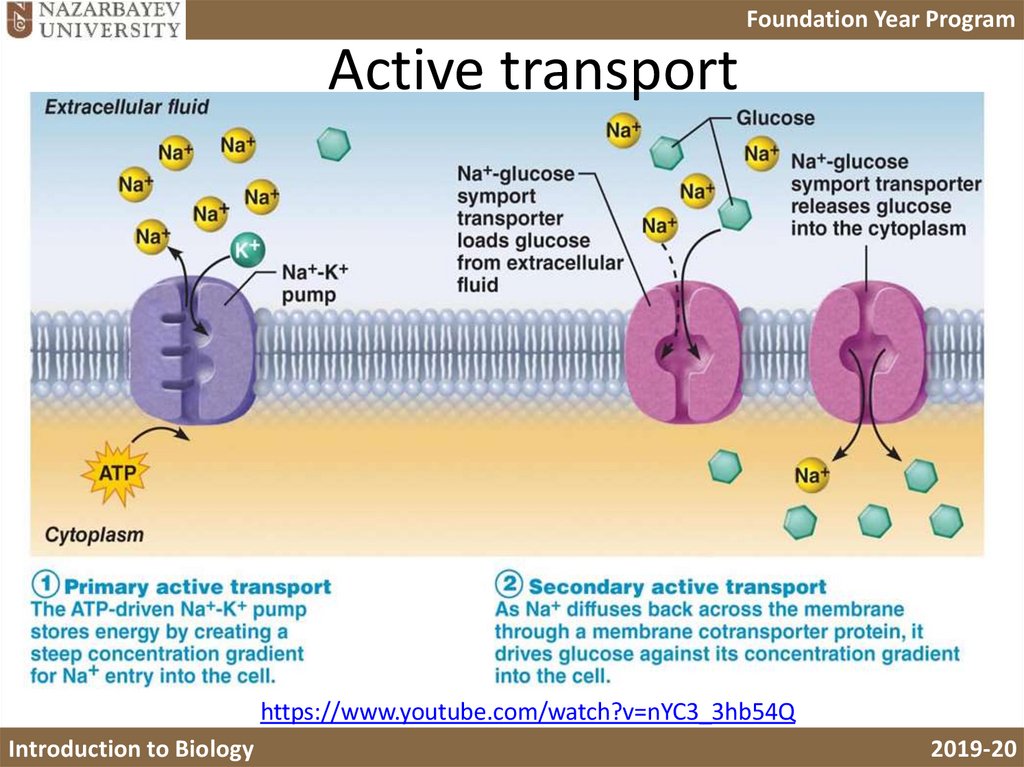
At its core, active transport refers to any mechanism by which a cell moves molecules across a membrane using energy to overcome a thermodynamic gradient. The key word is overcome. Diffusion does the work for you when things move downhill. Active transport does the work when things need to move uphill. Primary active transport uses energy directly from ATP or another high-energy molecule. Secondary active transport borrows energy from an ion gradient that was established by primary active transport. Both are real. Both are important. Confusing them is common and leads to real mistakes. I remember struggling through a membrane physiology lab in grad school where we were trying to isolate the contribution of the sodium-calcium exchanger in cardiac myocytes. We set up patch-clamp recordings and blocked the Na+/K+ pump with ouabain. The calcium handling went haywire. The textbook explanation didn't cover the messy interference we saw between secondary active transporters when you disrupted one gradient. It took me weeks of tweaking the solutions and running control after control to separate the signal from the noise. The problem was that blocking the sodium pump changed intracellular sodium, which in turn altered the driving force for the sodium-calcium exchanger, which is a classic example of secondary active transport. You have to think about the whole system, not just the component you're studying. One thing that doesn't get enough attention is that active transport is saturable. The proteins involved are finite in number, and they have a maximum turnover rate. When you're working with drug transporters or nutrient uptake in a research context, assuming linear uptake across all concentrations is a mistake. At high substrate concentrations, the transporters max out and you hit Vmax. The kinetics look like Michaelis-Menten. This is why dosing regimens for certain medications depend on how much of the carrier protein is available in the gut or kidney. It's not just about concentration gradients anymore.
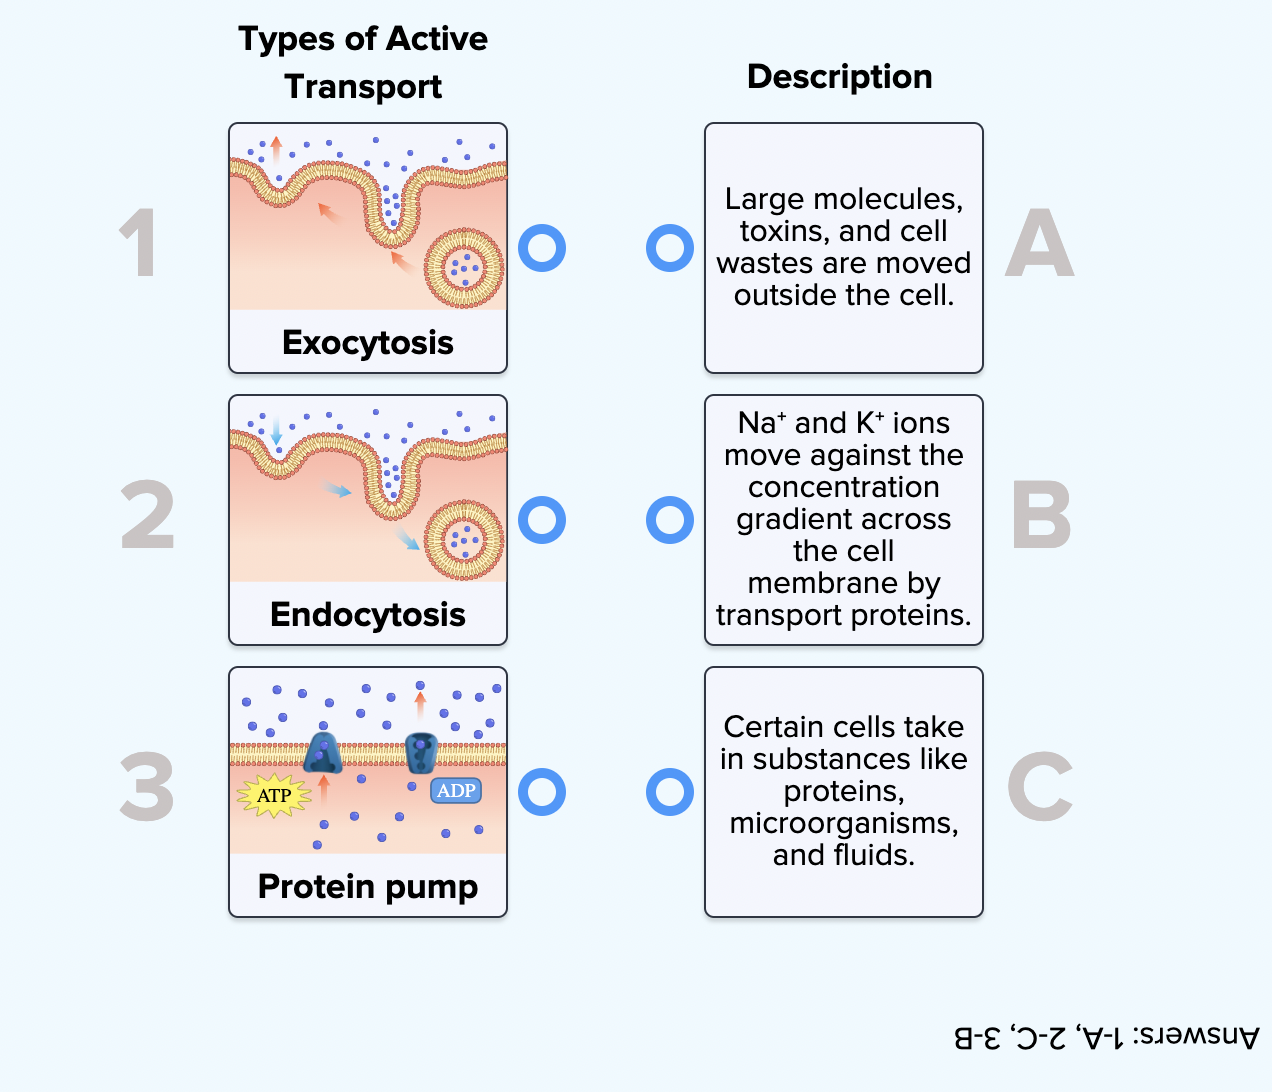
Another nuance people miss is that active transport isn't exclusively about small ions and molecules. Vesicular transport, which includes endocytosis and exocytosis, is sometimes classified as a form of active transport because it requires ATP. The distinction between protein-mediated transport and vesicular transport is more about scale than principle. Both move things against favorable gradients. Both consume energy. Both fail under similar stress conditions like temperature shifts or membrane disruption. There are real limitations here. Active transport proteins can be inhibited by changes in membrane potential, temperature, pH, or the presence of certain toxins. Cyanide shuts down ATP production and within seconds active transport grinds to a halt across every cell in your body. Heavy metals like mercury and lead can bind to the cysteine residues on transport proteins and disable them. Some pharmaceuticals work by selectively inhibiting specific transporters, which is both a mechanism of action and a source of side effects. Digoxin, for example, inhibits the Na+/K+ ATPase in the heart. It's useful for heart failure but toxic at slightly higher doses because it affects the pump everywhere, not just in cardiac tissue. If you're studying this for an exam, focus on understanding the difference between the pump mechanisms and the exchanger mechanisms. The pump moves ions using direct ATP hydrolysis. The exchanger couples the movement of one ion down its gradient to the movement of another ion against its gradient. Both are essential. Both are taught separately and then expected to work together in problems that assume you can integrate them without guidance. That's on the curriculum designers, not you.
Get the Full Details
Practical applications include understanding how diuretics work in the kidney, how antibiotics cross bacterial membranes, and why certain cancers develop resistance to chemotherapy by upregulating efflux pumps like P-glycoprotein. The latter is particularly relevant. When tumor cells overexpress these transporters, they actively pump the drug out faster than it can accumulate to therapeutic levels. Reversing that requires inhibitors that block the pump, which brings us back to the saturability problem and the risk of off-target effects. The bottom line is that active transport is a fundamental cellular process that operates under constraints most introductory courses don't emphasize. It costs energy. It has limits. It interacts with other transport systems in ways that are difficult to predict without understanding the underlying thermodynamics. Learning to think about membranes as dynamic, energy-dependent structures rather than simple filters will serve you better than memorizing the sodium-potassium pump cycle for the tenth time.