The Practical Reality of Aerobic Cellular Respiration
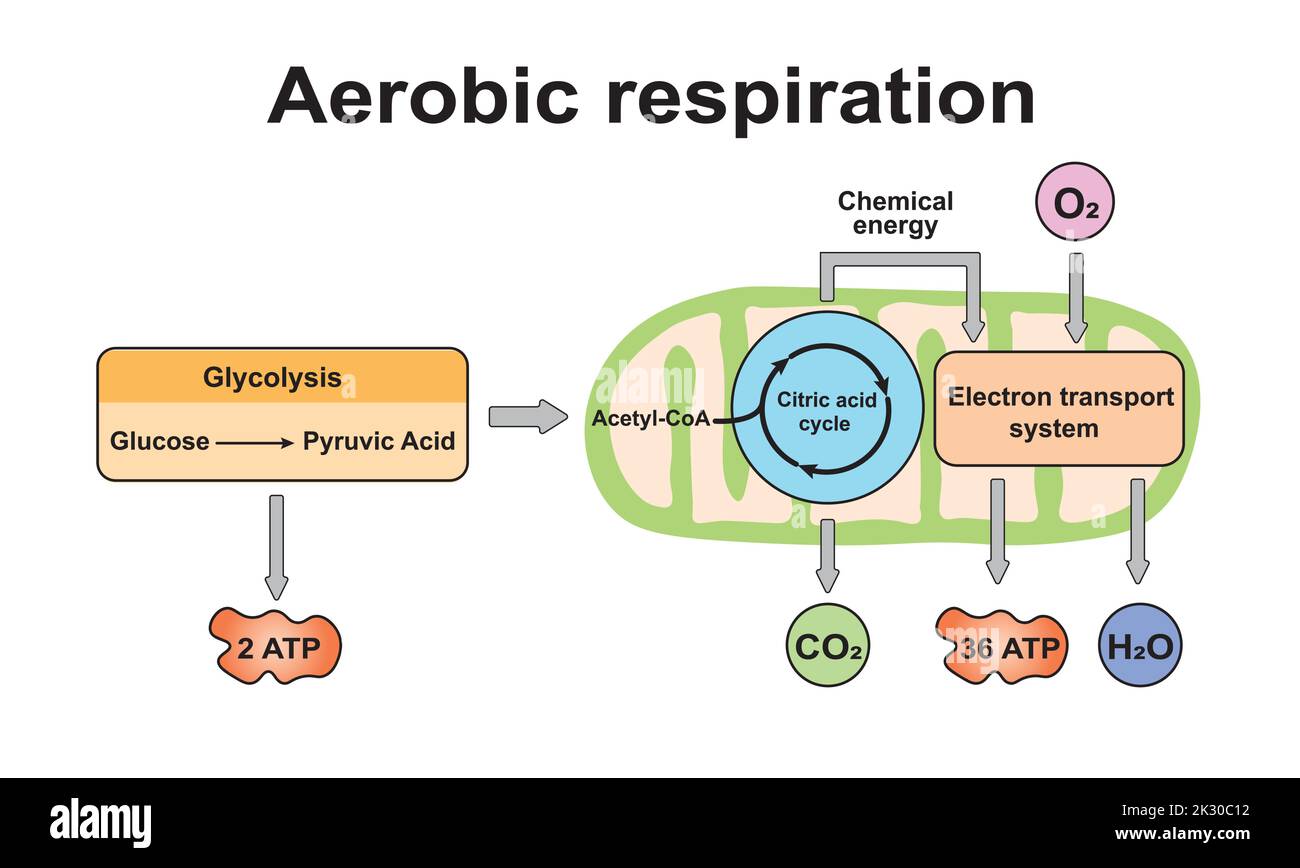
Most people learn this topic in high school biology and then never think about it again. The standard textbook diagram shows a clean flowchart: glucose enters, carbon dioxide leaves, and ATP appears somewhere along the way. In practice, it's messier than that. Aerobic cellular respiration is the metabolic pathway that uses oxygen to extract energy from organic molecules, primarily glucose, and convert it into adenosine triphosphate. The overall equation is straightforward — C6H12O6 plus six O2 yields six CO2, six H2O, and roughly 30 to 32 ATP molecules. But the actual mechanism involves four distinct stages that span two cellular compartments, and the stoichiometry breaks down if you try to memorize it without understanding the underlying bioenergetics. I've sat through too many lab sessions where students calculate a theoretical yield of 36 or 38 ATP and then get confused when their experimental data doesn't match. The modern accepted range is 30 to 32, and the reason has to do with the cost of transporting ADP and phosphate into the mitochondrion and the actual proton-to-ATP ratio required by the F1Fo ATP synthase, which turned out to be around 4 protons per ATP, not the 3 that older textbooks assumed.
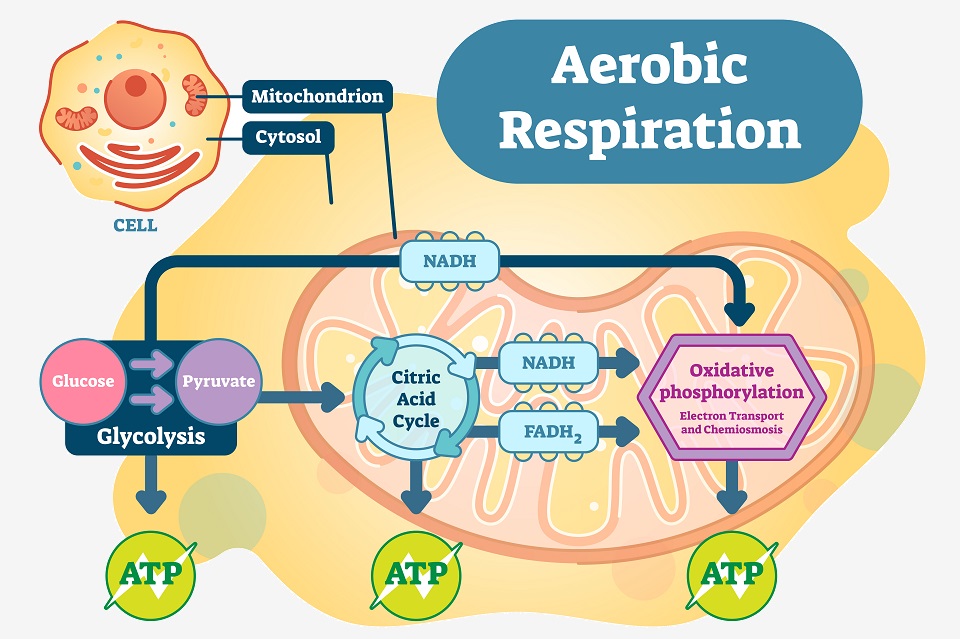
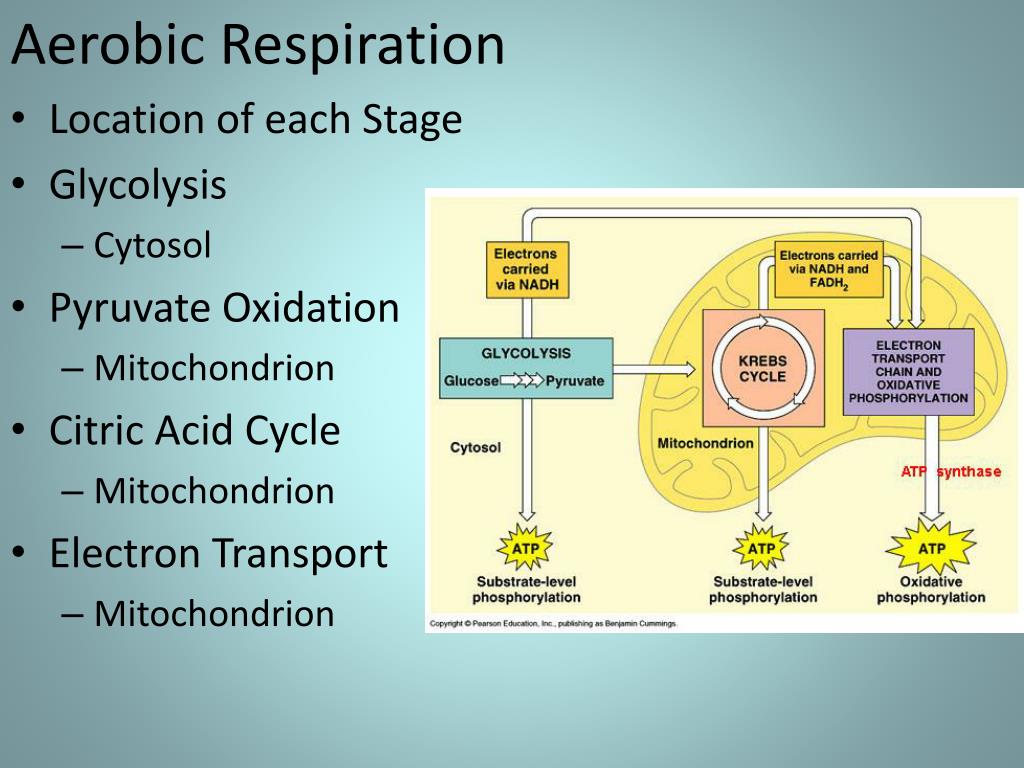
The process really starts with glycolysis in the cytoplasm, where one glucose molecule is split into two pyruvate molecules, generating a net gain of 2 ATP and 2 NADH. That part is simple enough. The problem begins when you have to decide whether those 2 cytoplasmic NADH molecules even make it into the mitochondria intact. Depending on which shuttle system is active — the malate-aspartate shuttle or the glycerol-3-phosphate shuttle — you either preserve their reducing equivalents at full value or you lose half of them as they get converted to FADH2 at the inner membrane. In liver and heart tissue, the malate-aspartate shuttle dominates. In skeletal muscle and brain, the glycerol-3-phosphate shuttle is more common. This detail alone shifts your total ATP yield by about 2 molecules per glucose, and most introductory courses completely skip over it.
Where Things Actually Happen Inside the Cell
After glycolysis, each pyruvate enters the mitochondrial matrix and gets converted into acetyl-CoA by the pyruvate dehydrogenase complex. This step releases one CO2 per pyruvate and generates one NADH. Two pyruvates mean two turns through this link reaction, so you've already accounted for 2 NADH and 2 CO2 before the Krebs cycle even starts. The citric acid cycle — sometimes called the Krebs cycle or TCA cycle — then processes each acetyl-CoA through eight enzymatic steps. Per turn, it produces 3 NADH, 1 FADH2, 1 GTP (which is functionally equivalent to ATP), and releases 2 CO2. Two turns per glucose molecule give you 6 NADH, 2 FADH2, and 2 GTP from this stage alone. Here's the part most people gloss over: the NADH and FADH2 are not energy products themselves. They're electron carriers. The actual energy capture happens at the electron transport chain, which sits embedded in the inner mitochondrial membrane. Complexes I through IV pass electrons from NADH and FADH2 through a series of redox reactions toward molecular oxygen, which acts as the terminal electron acceptor and gets reduced to water. The energy released at each transfer step is used to pump protons from the matrix into the intermembrane space, creating an electrochemical gradient.
Get the Full Details

Oxidative phosphorylation is what happens next. Protons flow back into the matrix through ATP synthase, and the mechanical rotation of that enzyme drives the phosphorylation of ADP. This is chemiosmosis, and it accounts for roughly 26 to 28 of the total ATP produced per glucose molecule. Without it, aerobic respiration would be functionally equivalent to fermentation, which is why the presence of oxygen makes such a dramatic difference in yield.
The Edge Case That Almost Broke My Data Set
I ran a respiration experiment using isolated rat liver mitochondria and measured oxygen consumption rates while adding different substrates. When I used succinate as the substrate instead of NADH-linked fuel like pyruvate or glutamate, the P/O ratio dropped noticeably compared to published values. It took me three days to figure out that the preparation I was using had a partially compromised inner membrane integrity — small leaks in the proton gradient meant some of the energy from electron transport was dissipating as heat rather than driving ATP synthesis. The workaround was measuring citrate synthase activity as a marker of mitochondrial contamination in the prep and comparing it against protein content to verify that my mitochondrial isolation was clean enough. Once I confirmed the integrity issue, I adjusted my calculations to account for the measurable proton leak and the data finally aligned with expected ranges. If you're working with isolated mitochondria and your oxygen consumption numbers look reasonable but your ATP yield doesn't add up, check membrane integrity before you assume your respiration quotients are wrong. It's almost always the prep, not the theory.
Counter-Intuitive Things That Beginners Miss
First, ATP is not the only thing this process produces. A significant fraction of the proton gradient is deliberately dissipated by uncoupling proteins, particularly UCP1 in brown adipose tissue. This isn't a malfunction — it's how hibernating animals and human infants generate heat. The mitochondria are burning fuel without making ATP, and the energy goes straight to warming blood. If you treat aerobic respiration as purely an ATP-generating pathway, you're missing a major physiological function it serves. Second, the rate of aerobic respiration is not primarily limited by the availability of oxygen under normal conditions. It's regulated by the energy demand of the cell, which shows up as the concentration of ADP and inorganic phosphate. This is called respiratory control, and it's why mitochondria in resting muscle consume oxygen much more slowly than in active muscle. Add ADP to a mitochondrial prep and oxygen consumption spikes immediately. Remove it and the chain nearly stops. The system is feedback-driven, not substrate-limited, in healthy tissue. There's also a practical limitation worth noting: the electron transport chain is highly sensitive to certain inhibitors. Cyanide blocks complex IV. Rotenone blocks complex I. Antimycin A blocks complex III. These aren't just academic curiosities — they're relevant if you're ever trying to interpret respiration data from treated cells. A complete shutdown of complex IV means the entire chain backs up, NADH can't be reoxidized, and glycolysis stalls within seconds because there's no NAD+ available. That's why cyanide is lethal at microgram-per-kilogram doses — it doesn't just reduce ATP production, it halts it entirely.
When Aerobic Respiration Just Won't Work for You
If you're studying organisms or cell types that live in low-oxygen environments, aerobic respiration is simply not an option. Some protists and certain parasitic worms have mitosomes or hydrogenosomes that perform modified forms of anaerobic metabolism. In humans, cancer cells often rely heavily on aerobic glycolysis — the Warburg effect — even when oxygen is plentiful, because the ATP yield per glucose is far lower but the biosynthetic intermediates they produce support rapid proliferation. If your question is about maximizing ATP yield per fuel molecule, aerobic respiration is unbeatable. If your question is about something else entirely, like fast glucose consumption or biosynthetic precursor generation, the answer changes completely. The takeaway isn't that aerobic respiration is poorly understood. It's one of the most thoroughly characterized pathways in biochemistry. The takeaway is that the textbook version leaves out enough details that applying it to real biological systems or experimental data requires knowing where the gaps are. The shuttle systems, the actual proton stoichiometry, the role of uncoupling, and the regulatory logic around ADP availability are the things that separate a memorized equation from an working understanding of what's actually happening inside every mitochondrion in your body right now.