Understanding Chromosomal Crossing Over
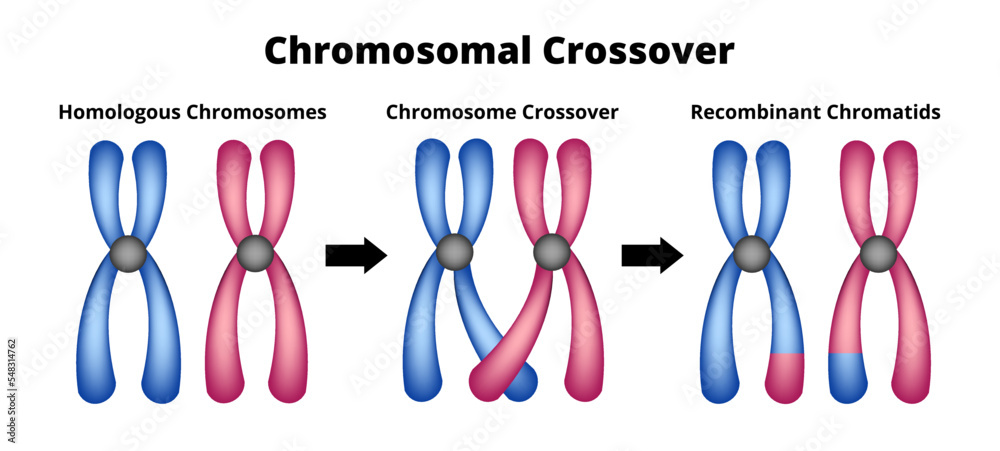
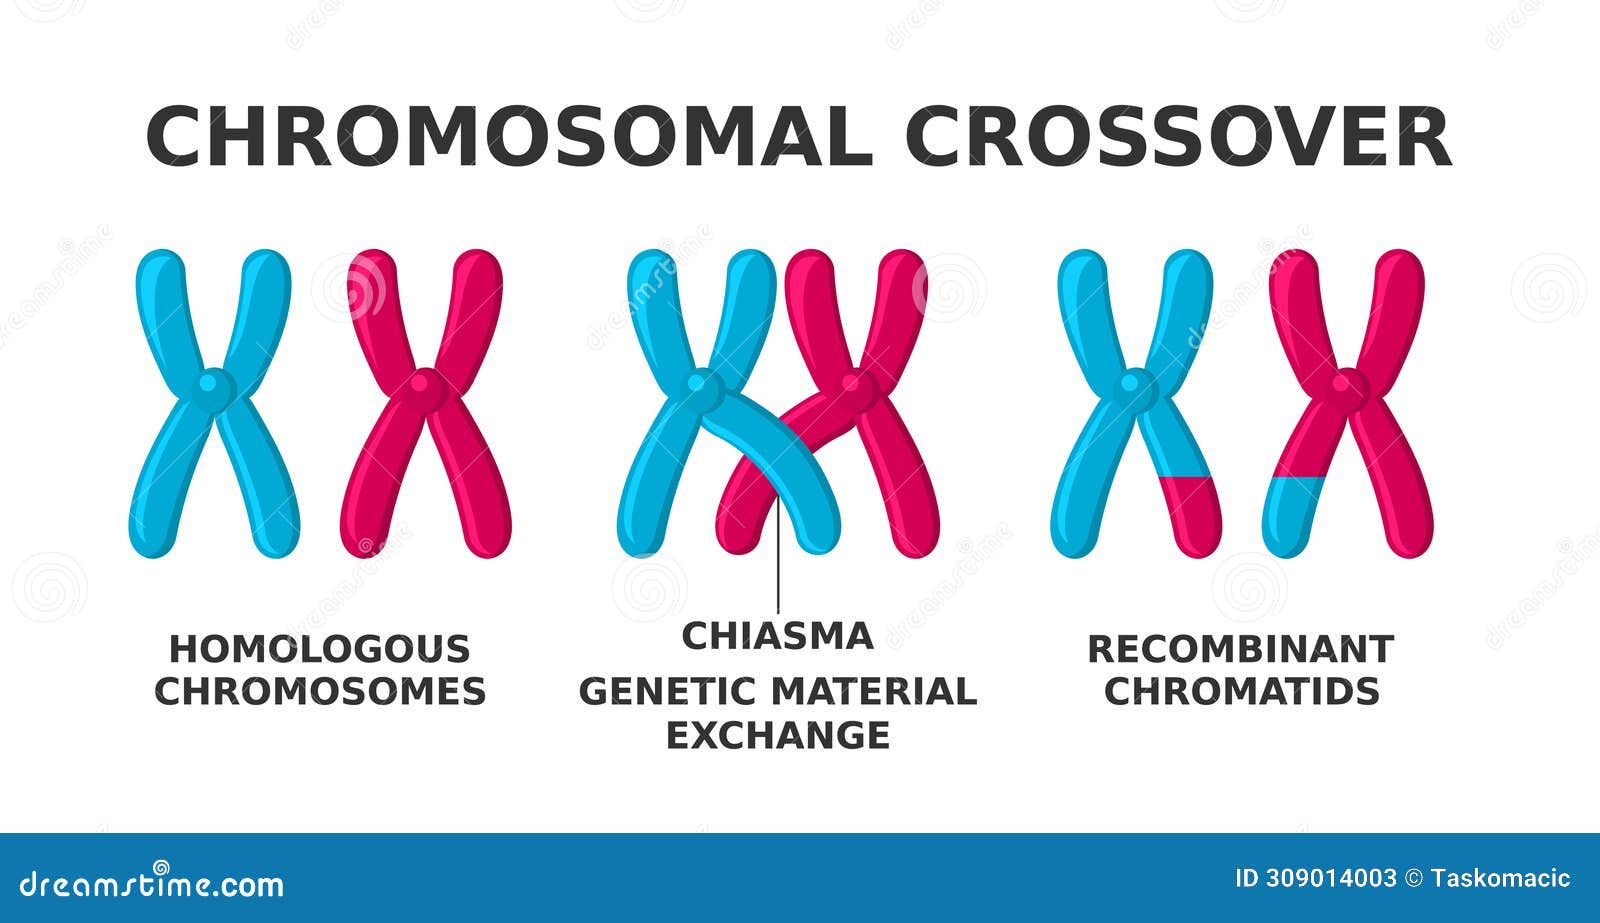
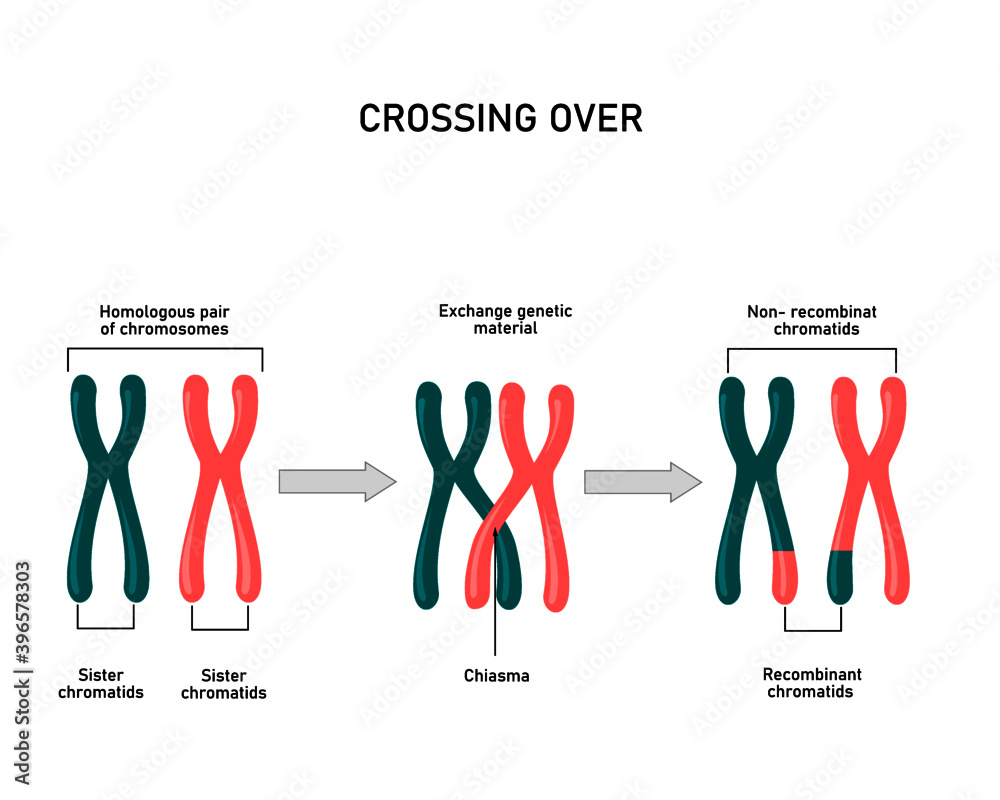
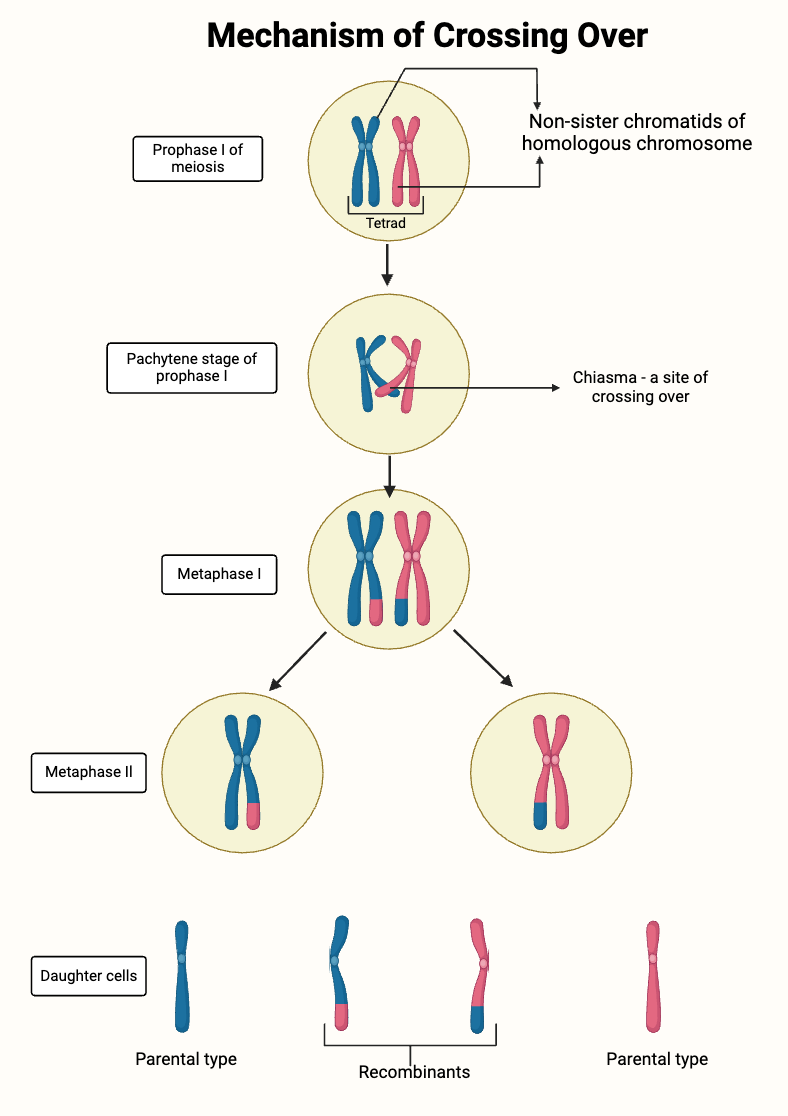
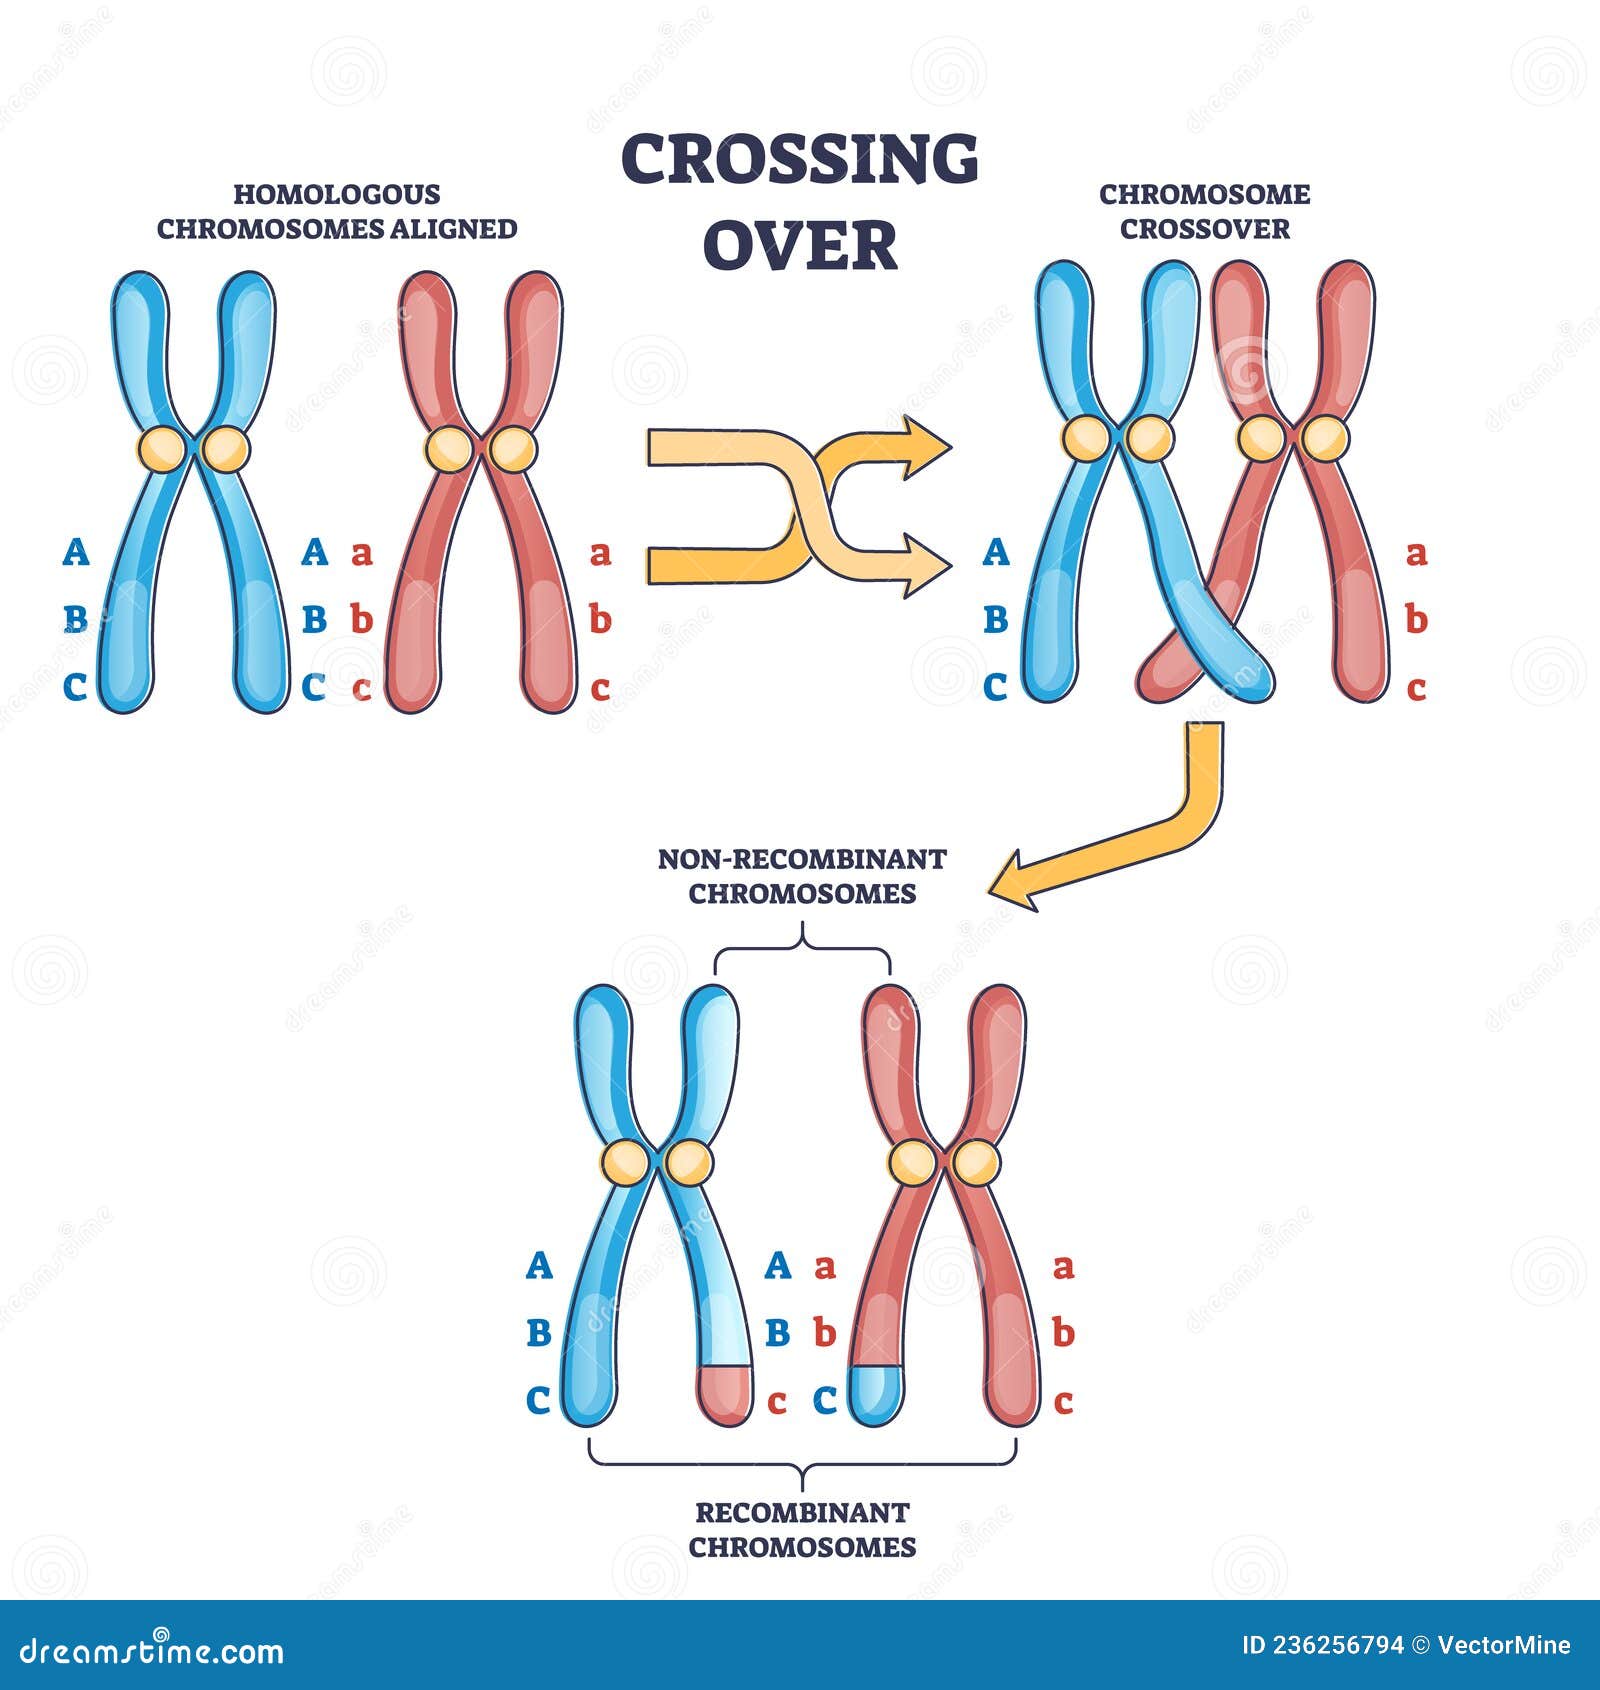
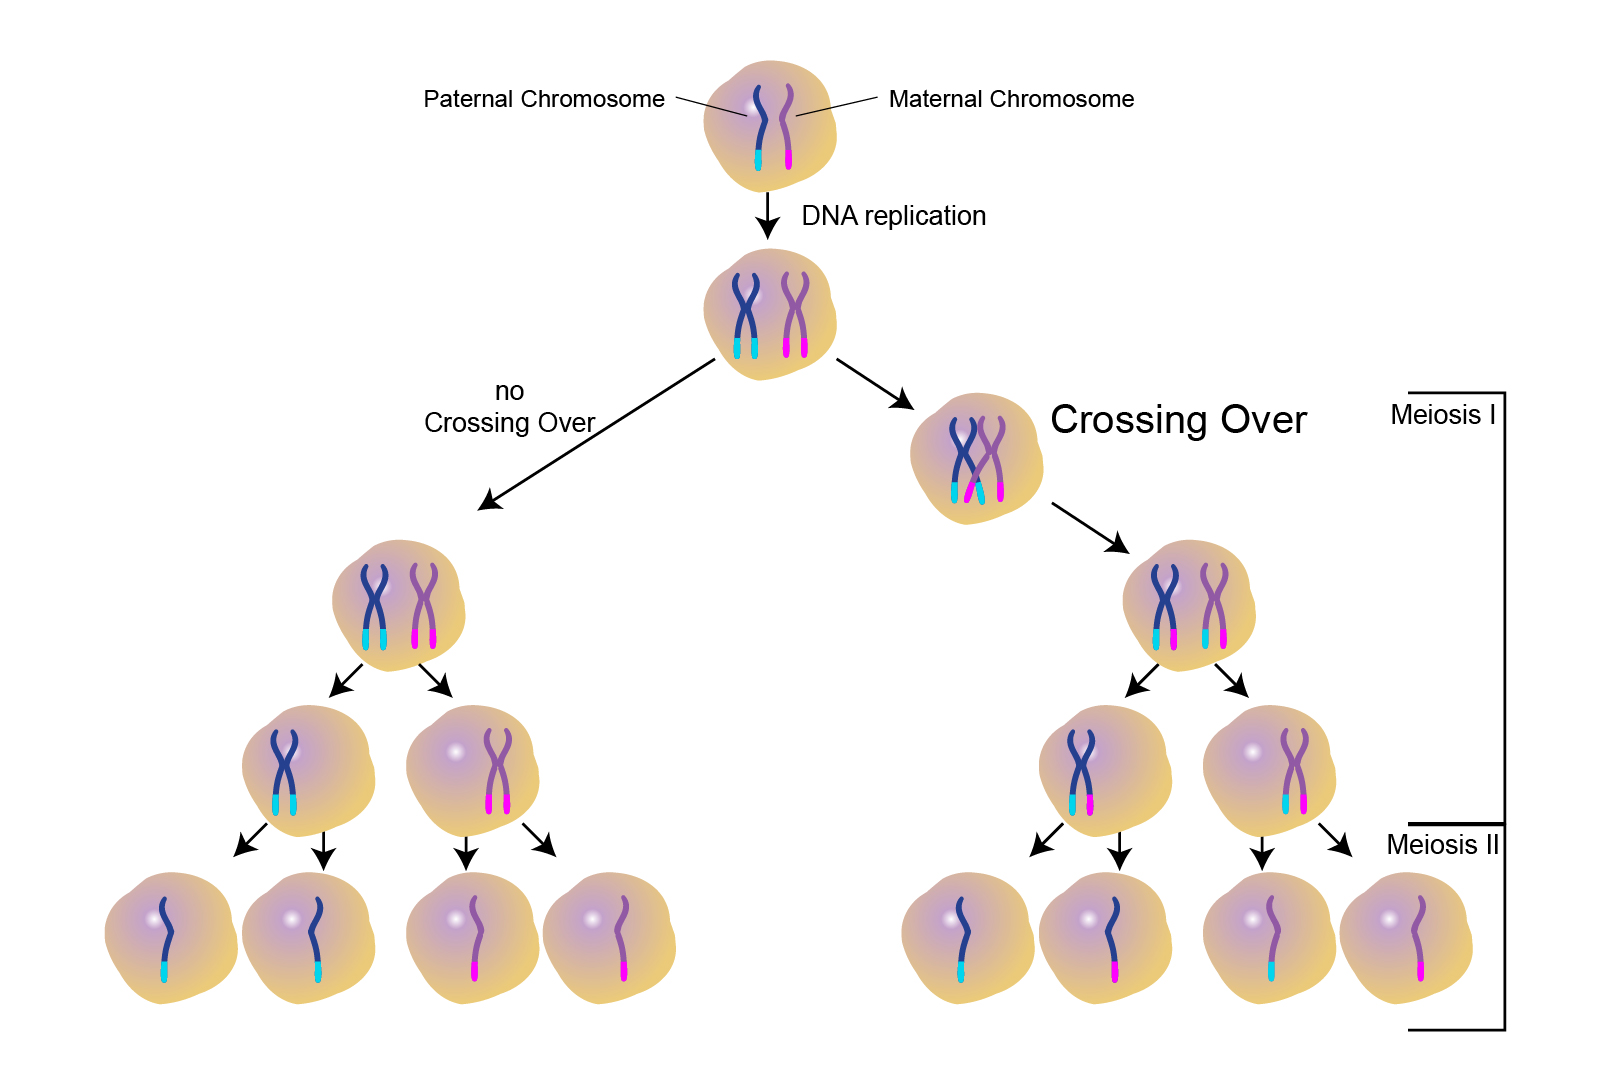
When you look at a chromosome spread under a microscope during meiosis, you are seeing the physical result of a very messy molecular process. Crossing over is the exchange of genetic material between homologous chromosomes. It happens during prophase I of meiosis, specifically at the pachytene stage, when paired chromosomes (called bivalents or tetrads) visibly swap segments. The result is recombinant chromatids — chromosomes that carry a mix of maternal and paternal alleles instead of the original linkage. Here is the mechanism in plain terms. Before crossover occurs, each chromosome has already replicated, so you have two sister chromatids per chromosome. The homologous chromosomes pair up tightly along their entire length. Enzymes create double-strand breaks in the DNA, and the broken ends invade the homologous chromosome. This forms structures called Holliday junctions. When those junctions are resolved, you get either a crossover (exchange of flanking markers) or a non-crossover event. Most of the time in a given cell, you get somewhere between one and three crossover events per chromosome pair in humans. Some chromosomes get more, some get fewer. It is not evenly distributed.
What Is Crossing Over in Practical Terms
The practical significance of crossing over is that it shuffles alleles. Without it, all the genes on a single chromosome would always be inherited together as a block. Think about a chromosome carrying genes for blood type, eye color, and a disease marker — all physically linked. Crossing over breaks those linkages in predictable ways. That predictability is what lets geneticists map genes to specific chromosomal positions. A recombination frequency of one percent equals one map unit, or one centimorgan. Ten percent recombination means the genes are roughly ten centimorgans apart on the same chromosome. The formula itself is straightforward: recombination frequency equals the number of recombinant offspring divided by the total number of offspring, multiplied by one hundred. But applying it correctly requires understanding that this relationship only holds for relatively short distances. Beyond about fifteen to twenty centimorgans, the observed recombination frequency underestimates the actual physical distance because multiple crossover events cancel each other out. Two crossovers between the same two markers produce parental-type gametes that look like no recombination happened at all. This is why genetic maps are additive only over short intervals and why you need multiple marker genes to build an accurate map across a large chromosomal region. I spent a semester trying to map three linked genes in Drosophila for an undergrad genetics lab. We were tracking body color, wing shape, and eye color. The recombination frequencies came out to roughly eighteen percent between gene A and gene B, twelve percent between gene B and gene C, and twenty-eight percent between gene A and gene C. Simple addition says A to B plus B to C should equal A to C. Eighteen plus twelve is thirty, not twenty-eight. The discrepancy was double crossovers — rare events where two exchanges happened between A and C, flipping the middle gene back into the parental configuration. If you do not score the middle gene separately, those double crossover individuals look parental for the outer markers and you completely miss them. The workaround was running a three-point cross and explicitly identifying the double recombinant phenotypes, then adding them twice to the recombination calculation for each interval. That corrected the map to something closer to thirty centimorgans between A and C, which matched the expected distance from published reference maps.
There are limitations people do not always emphasize. Crossing over does not occur at random positions along a chromosome. In many organisms, including humans, there are hotspots — specific DNA sequences where recombination is far more likely. The PRDM9 protein controls hotspot placement in mammals, and variation in this gene between individuals means your crossover hotspots may not match anyone else's. There is also interference, which means one crossover event reduces the probability of another crossover nearby. Positive interference is the normal case. Complete interference would mean exactly one crossover per chromosome pair, but that is rare. Partial interference is the default, and it makes simple map addition slightly inaccurate even at moderate distances. Another practical limitation is that recombination frequency peaks at fifty percent. Once two genes are far enough apart on the same chromosome, or on different chromosomes entirely, they appear to assort independently. You cannot tell from a standard cross whether two unlinked-appearing genes are on different chromosomes or just very far apart on the same one. You need physical mapping techniques — FISH, sequence alignment, or cytogenetic analysis — to resolve that ambiguity. A fifty percent recombination frequency tells you nothing about actual chromosomal location beyond "they behave as if unlinked." Non-disjunction is another edge case worth noting. If crossing over fails to occur between a chromosome pair, the homologs may not segregate properly during meiosis I. This is particularly problematic for small chromosomes that rely on at least one crossover for proper spindle attachment. The resulting gametes can end up with zero copies or two copies of a chromosome, leading to conditions like Turner syndrome or Klinefelter syndrome when fertilization proceeds. In plant breeding, this is a known issue with certain hybrid combinations where chromosome pairing is too divergent for crossover to initiate reliably.
Get the Full Details
For anyone working with genetic data, the takeaway is that crossing over is a measurable, calculable phenomenon with well-understood mechanics, but applying it to real data requires accounting for double crossovers, interference, hotspot variation, and the fifty percent ceiling. The math works cleanly on paper. The data rarely does.