The Actual Mechanics of Osmosis Beyond the Textbook
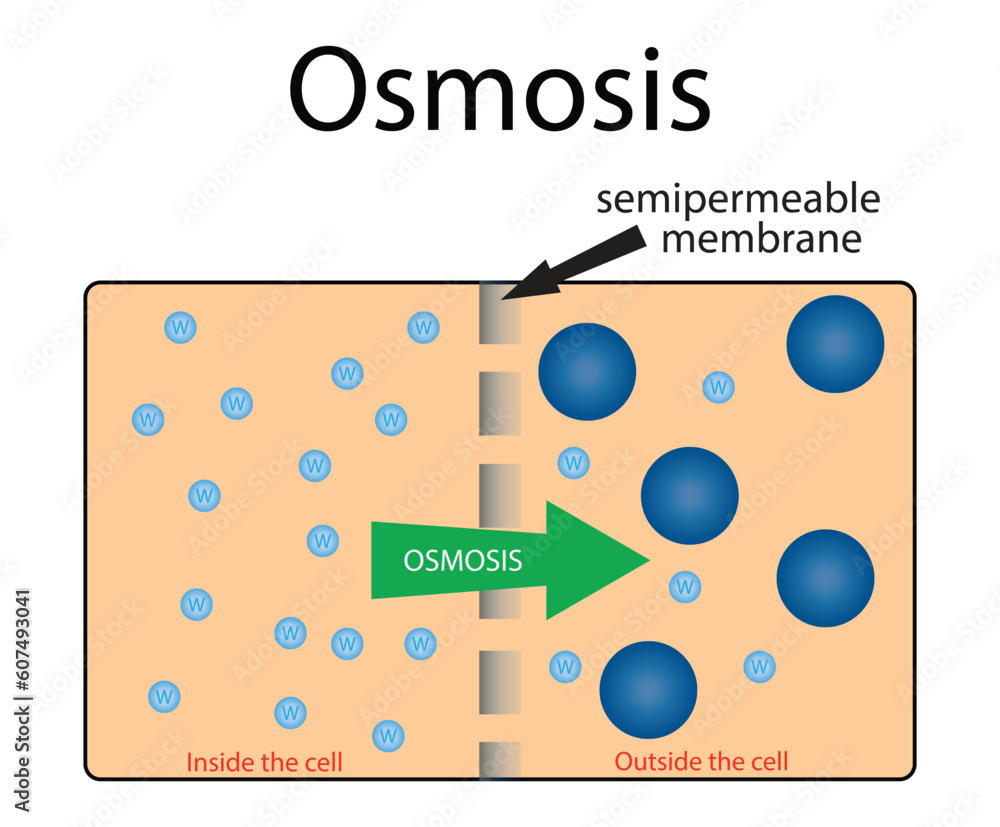
Osmosis is the net movement of water molecules across a selectively permeable membrane from a region of lower solute concentration toward a region of higher solute concentration. The driving force is the concentration gradient of the solvent itself, not the solute. Water moves to dilute the more concentrated side until equilibrium is approached or hydrostatic pressure counteracts the osmotic pull. In a biological context, osmosis explains how cells manage water balance, how kidneys concentrate urine, and why plant roots draw water from soil. It is not the same as simple diffusion. Diffusion describes the movement of any substance down its own concentration gradient. Osmosis specifically describes water movement driven by differences in solute potential across a membrane that water can cross but many solutes cannot. I used to see students confuse the two constantly. The distinction matters because the math and predictions diverge. If you are calculating water potential, you need osmotic potential and pressure potential as separate terms, not just a blanket diffusion model.
Water Potential Is the Framework That Actually Works
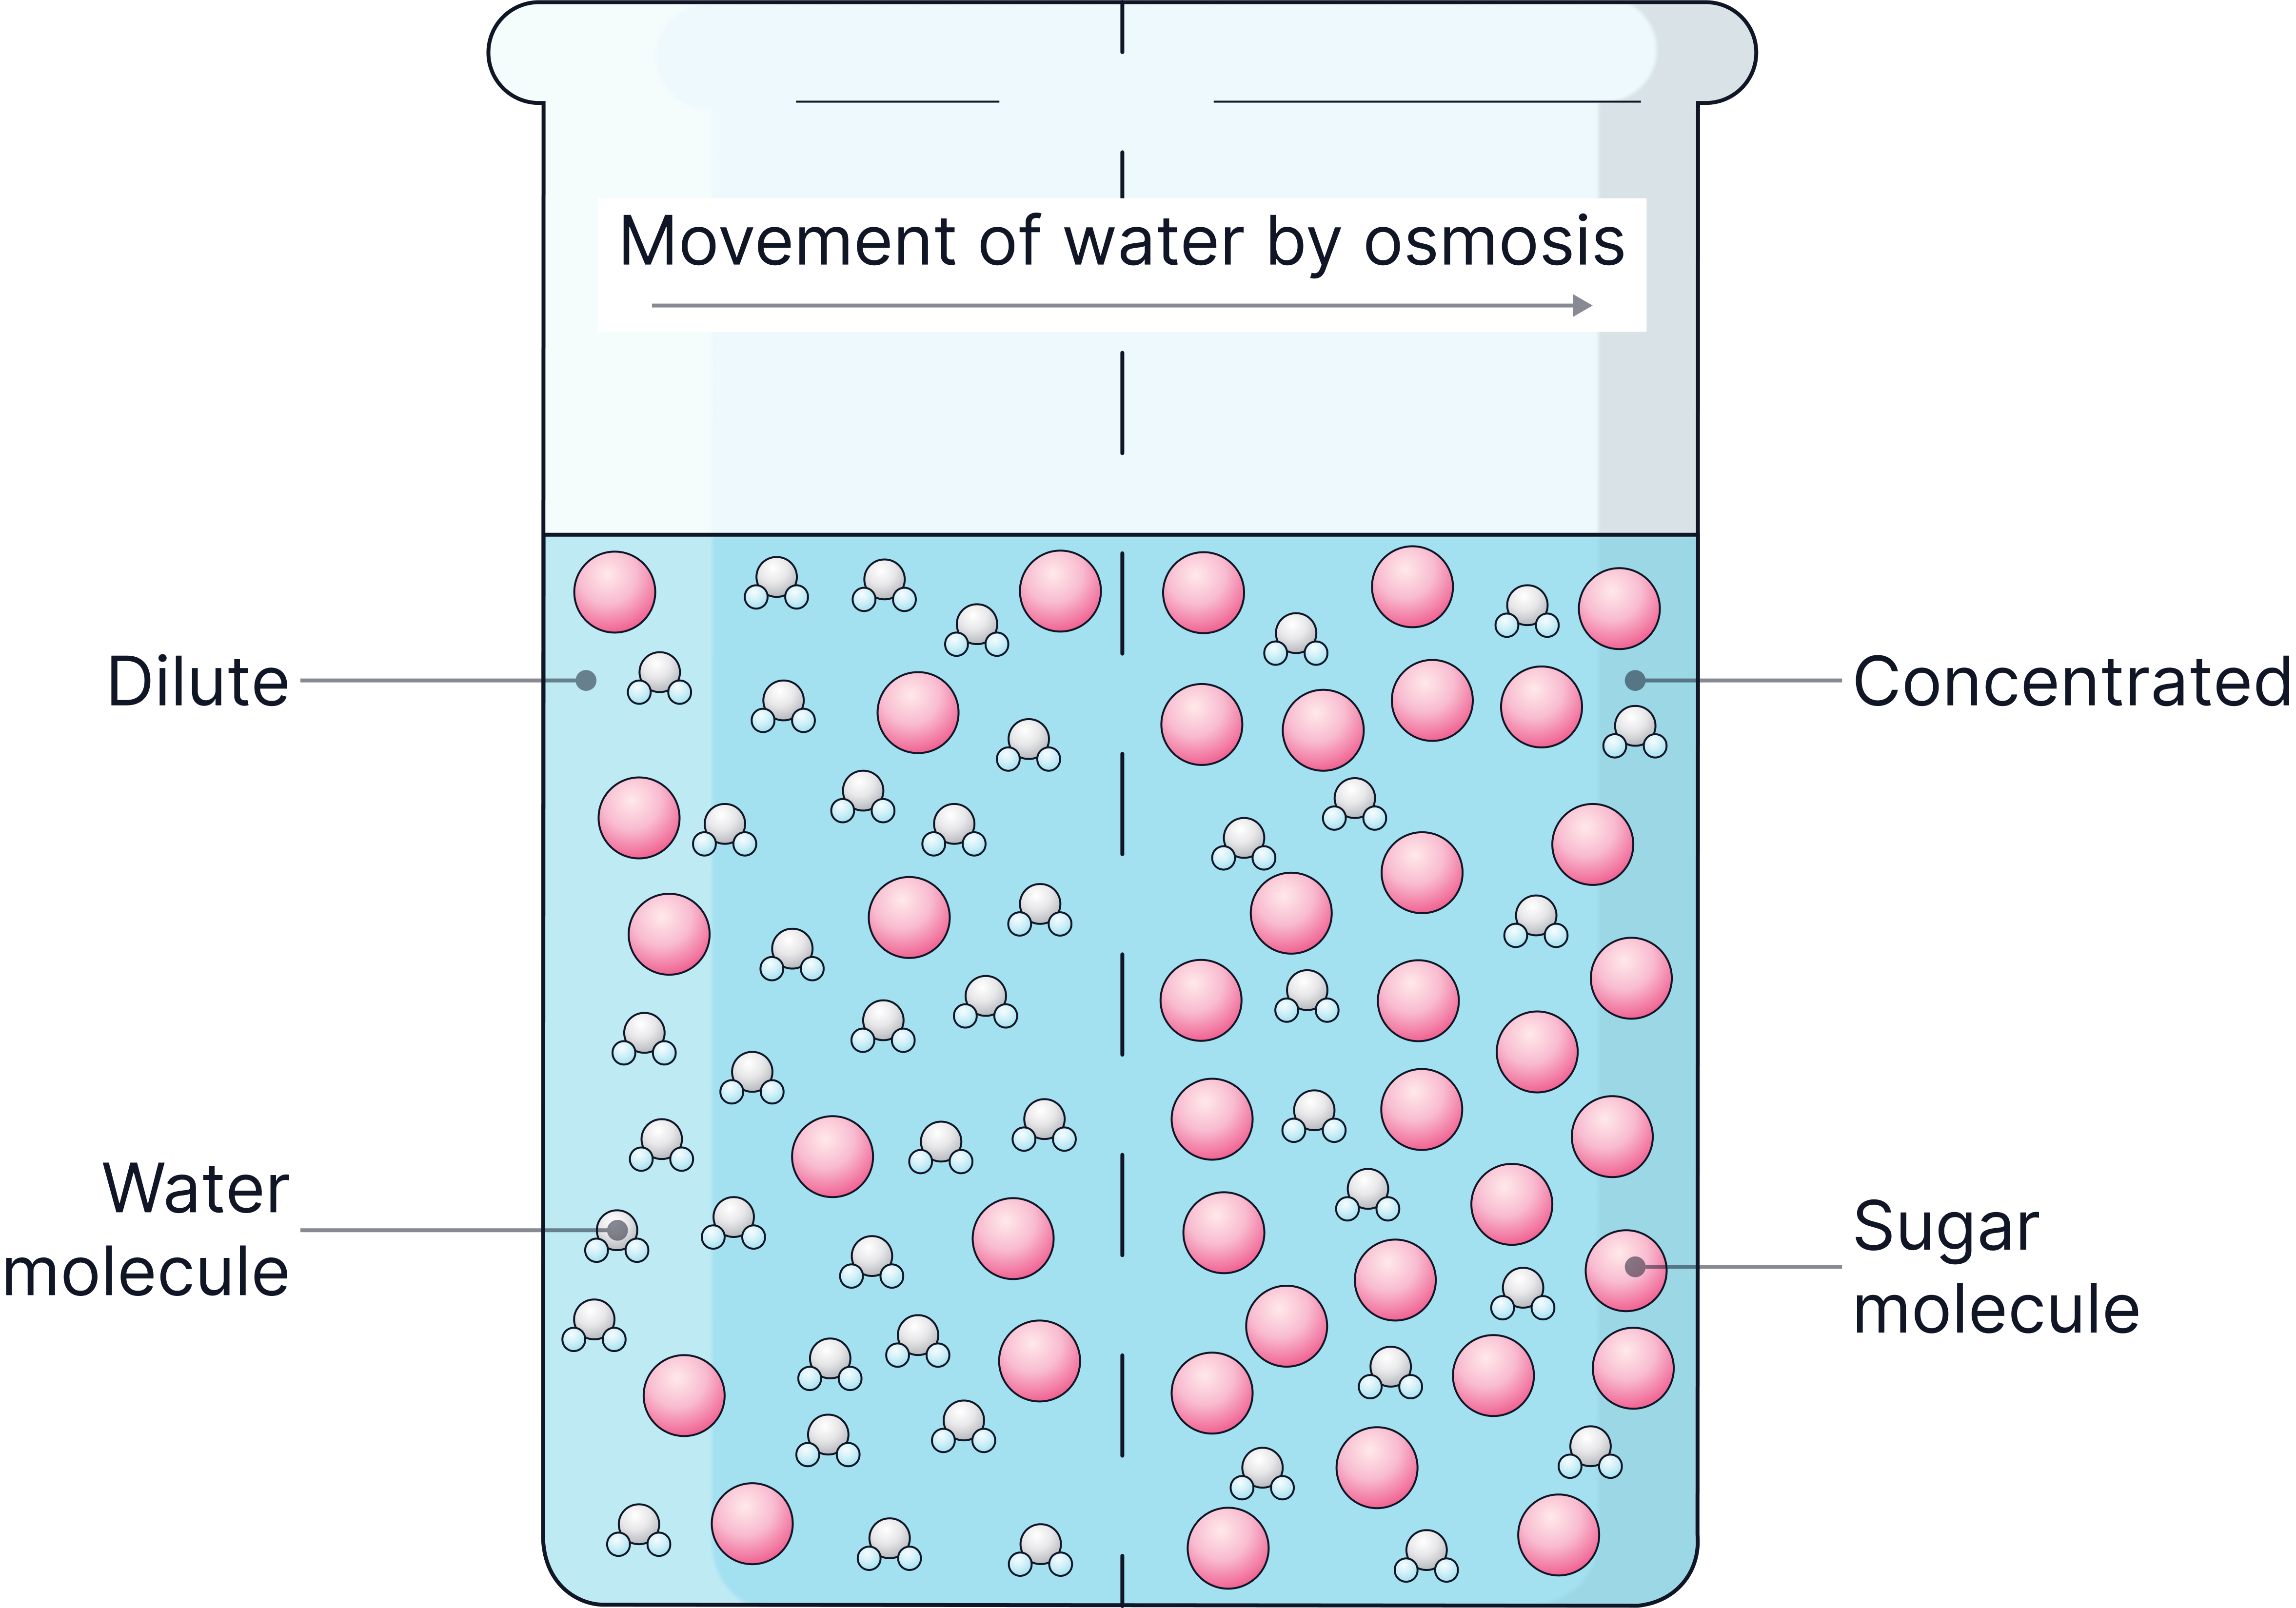
Biological osmosis is best modeled with water potential, expressed as psi or MPa. The equation is Psi = Psi_s + Psi_p + Psi_g, where Psi_s is solute potential, Psi_p is pressure potential, and Psi_g is gravitational potential. In most cellular scenarios, gravitational potential is negligible. Solute potential is always negative or zero. Pressure potential can be positive, negative, or zero depending on the system. Water always moves from higher water potential to lower water potential. This means from less negative to more negative. That directionality trips people up when they first encounter it. They picture water "attracted" to salt, which is not technically wrong as a shorthand, but it obscures the actual mechanism. Water moves because the chemical potential of water is lower on the concentrated side, not because salt pulls on water molecules directly. When I was running lab courses on membrane transport, I would set up U-tube experiments with dialysis tubing and different sucrose concentrations. The standard result tracks fine, but the edge case I always ran into involved temperature variation. Sucrose solutions change viscosity with temperature, and viscosity affects the rate of water movement through the membrane. I found that if the lab was more than three degrees off from the calibration temperature, the predicted equilibrium times were off by roughly twenty percent. The workaround was simple: equilibrate all solutions to room temperature in a water bath for at least thirty minutes before setting up the apparatus, and record the temperature. It added ten minutes to the prep time but eliminated a variable that was otherwise invisible in the data.
Hypertonic, Hypotonic, and Isotonic Are Useful but Limited
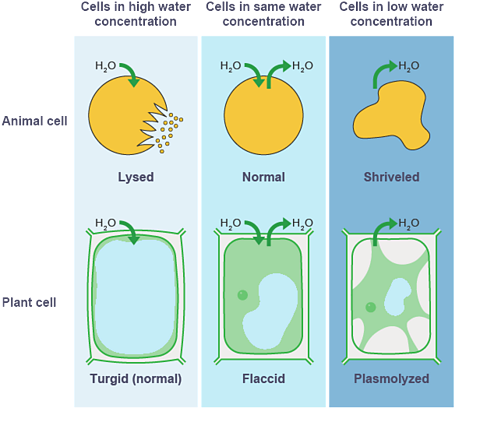
These terms describe relative solute concentrations between two solutions separated by a membrane. A hypertonic solution has higher solute concentration than the reference. A hypotonic solution has lower. An isotonic solution has equal concentration. In animal cells, hypotonic conditions cause water to enter the cell and potentially lyse it. Hypertonic conditions cause water to leave and the cell to shrivel. Isotonic conditions produce no net water movement. The limitation here is that these labels assume you are comparing the external medium to the cytoplasm. They do not tell you the rate of water movement, the volume change over time, or what happens when the membrane is not perfectly selective. Real biological membranes contain aquaporins, which dramatically increase water permeability. A cell with high aquaporin expression will reach equilibrium far faster than one without, even if the osmotic gradient is identical. This is why red blood cells respond to osmotic shock within seconds, while some epithelial cells take minutes. Another practical issue is that tonicity and osmolarity are not the same thing. Osmolarity measures total solute concentration. Tonicity measures the effective osmotic pressure that actually drives water movement, which depends on whether the solutes can cross the membrane. Urea is a classic problem. It is permeable across many cell membranes. A solution can be hyperosmotic because of urea, but isotonic in effect because the urea crosses the membrane and equalizes on both sides. I have seen exam questions trap students on this exact point, and it is a legitimate distinction that matters in clinical settings too, especially when managing IV fluids.
Get the Full Details
Practical Calculation Workflow
If you need to predict osmotic behavior quantitatively, start by determining the solute potential for each compartment. For non-electrolytes like sucrose, the formula is Psi_s = -iCRT, where i is the ionization constant, C is molar concentration, R is the pressure constant, and T is temperature in Kelvin. For electrolytes like NaCl, i accounts for dissociation. NaCl approximates i equals two in dilute solution. Then calculate pressure potential if it is relevant. In a plant cell, turgor pressure builds as water enters and pushes against the cell wall. At equilibrium, the inward osmotic drive equals the outward pressure potential. In an open system like a U-tube, hydrostatic pressure from the elevated column eventually balances the osmotic gradient. That is how osmotic pressure is measured experimentally: you wait until the fluid column stops rising and calculate pressure from the height difference. The common mistake here is forgetting to convert temperature to Kelvin and mixing up units for R. If you use atmospheres, R is 0.0821. If you use MPa, R is 0.00831. Pick one and stay consistent. Wrong units give you numbers that look plausible but are orders of magnitude off.
Where Osmosis Models Break Down
The standard textbook treatment assumes ideal behavior: dilute solutions, perfectly selective membranes, and constant temperature. Real systems violate all three assumptions frequently. Concentrated cytoplasm contains proteins and ions at levels that deviate from ideality. Membranes are not perfectly selective; they leak to some extent depending on composition and condition. Temperature fluctuates in living organisms, especially ectotherms. When working with concentrated solutions, the van't Hoff factor approaches unity and the simple equation underestimates osmotic pressure. You need activity coefficients from experimental data rather than calculated concentrations. This matters in industrial applications like reverse osmosis desalination, where feed water salinity varies and membrane fouling changes effective permeability over time. The theoretical calculations are useful for initial design, but they require empirical correction factors for accurate long-term prediction. Another scenario where the model fails completely is when the membrane is damaged or artificially permeabilized. If you treat a cell with a detergent, the membrane loses selectivity and osmosis as a controlled process stops. Water and solutes move freely until concentrations equalize by ordinary diffusion. This is why membrane integrity assays are a standard part of any transport study. Without them, your osmotic data is meaningless because you are measuring leakage, not osmosis.
The broader takeaway is that osmosis is a well-defined physical process, but its biological manifestation depends on membrane properties, solute permeability, and physical constraints that the basic definition does not capture. Understanding the core mechanism gets you through an introductory course. Understanding where it breaks down is what lets you work with it in any real setting.