Ecological succession is how biological communities change over time, and most people get it wrong because they only think about forests growing back after a fire.
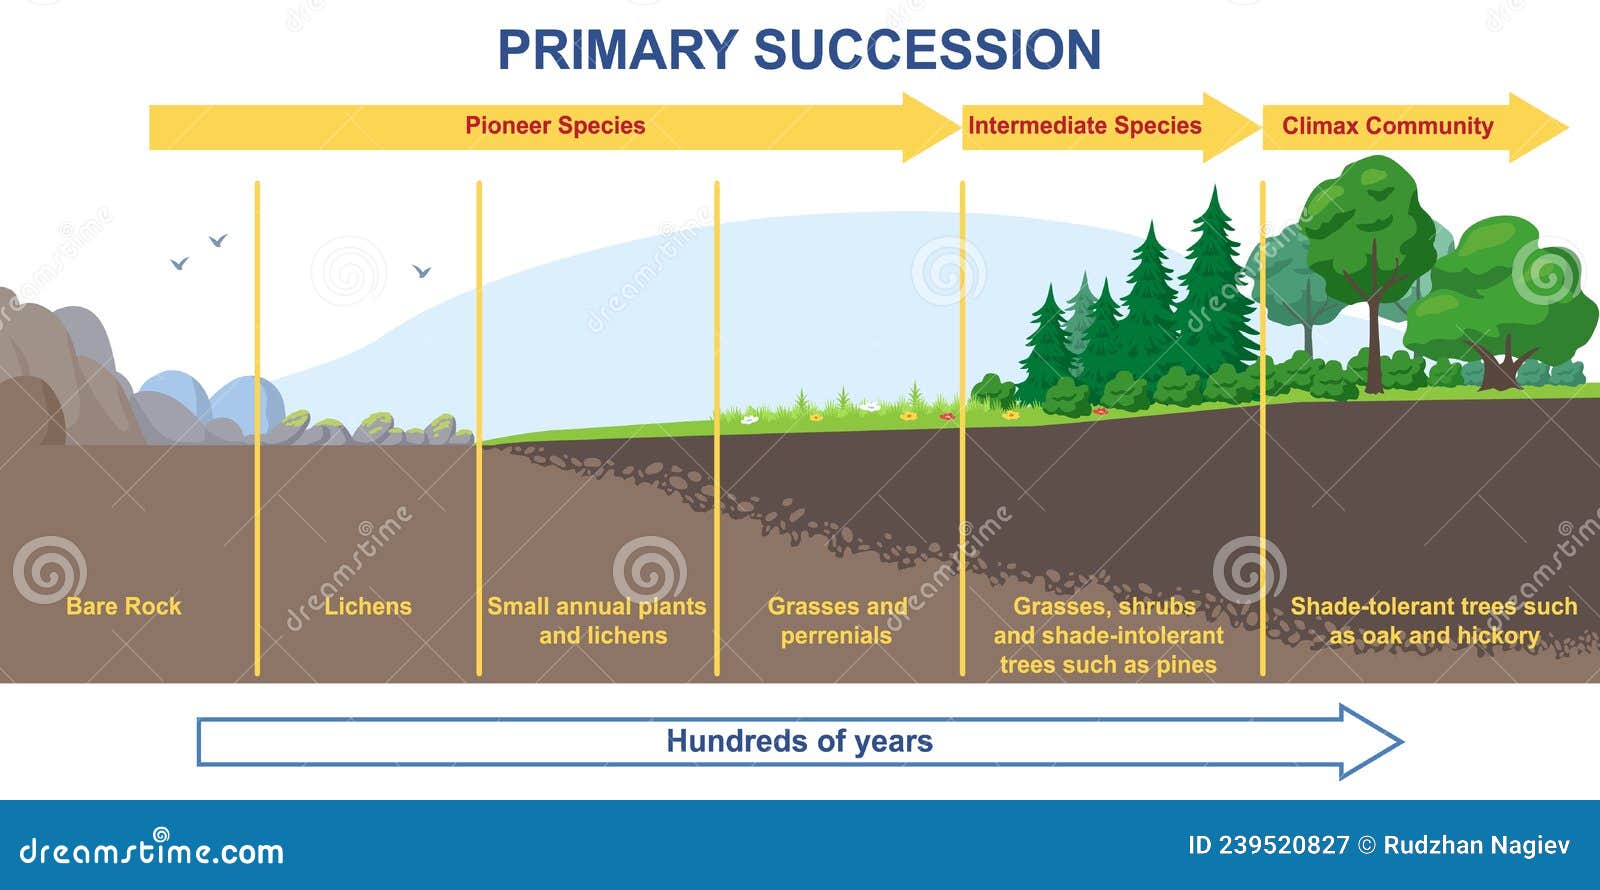
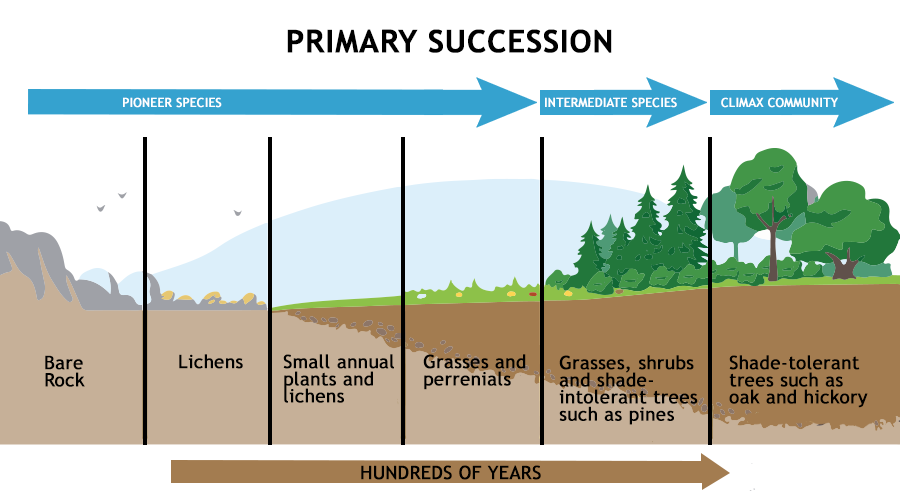
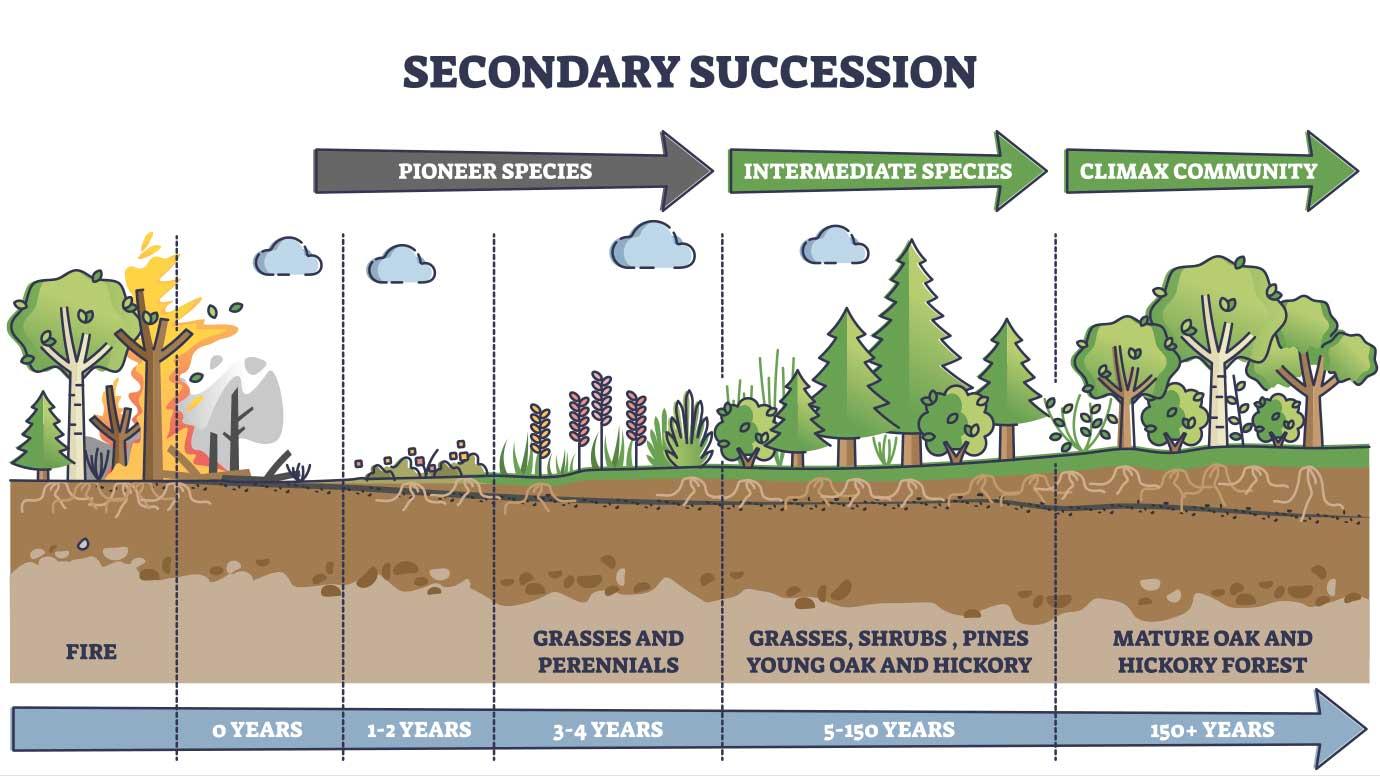
That is one type. The full picture is broader than that, which is why the term gets tossed around loosely in intro classes and then nobody really understands what happens when you dig into it. Succession describes the predictable sequence of community changes that occur after a disturbance creates an opening or exposes new substrate. Primary succession starts on bare rock or newly cooled lava with nothing organic. Secondary succession starts where soil already exists but the existing community has been wiped out or significantly altered. Those are the two buckets, and everything else is a nuance inside them. The mechanism is straightforward in theory. Pioneer species colonize first. They modify the environment. Later species move in and outcompete them. The community shifts toward something we call a climax state, which is a loaded term I will come back to. The whole process can take decades or centuries depending on climate, geography, and what the disturbance was.
How it actually plays out in the field
I spent a few years monitoring post-mining reclamation sites in Appalachia, and the textbook version does not hold up very well once you are standing in the dirt. The main problem is that soil chemistry at those sites is a mess. The underlying material is often acidic, nutrient-poor, and compacted from heavy equipment. Most people assume you just spread topsoil and plant natives, and that works sometimes, but the ground itself decides what actually grows, not the seed bag. At one site, we had a patch where the spoil material had an unusually high iron pyrite content. The oxidation was dropping pH to around 3.8 in the top twelve inches. Nothing standard would establish there except a few hardy grasses that died back after year two. The workaround was to amend with crushed limestone to neutralize acidity, but the reacts slowly, so you have to mix it deep, not just broadcast it on the surface. If you skip the mixing step, you end up with a layer of neutral soil sitting on top of acid rock, and the roots just don't go down past that interface. I wasted a full growing season on one quadrant because I assumed surface application would be enough. It wasn't. The plants failed by midsummer and the erosion started immediately.
The counter-intuitive parts people miss
First, succession is not always directional in a simple way. Facilitative models where early species help later species aren't the only pattern. There are also inhibitory models where early colonizers make it harder for others to establish, and tolerance models where later species just tolerate conditions that pioneers can't. The dominant pattern depends heavily on the stress level of the environment. In harsh conditions, facilitation matters more. In moderate conditions, competition and inhibition dominate. That means you can't predict the sequence just from knowing what species are present in the region. You need to know the environmental context. Second, the climax concept is basically broken for most practical purposes. The idea of a stable endpoint community assumes climate and disturbance regimes are constant, which they are not. With shifting weather patterns, a site that was approaching one type of climax community thirty years ago might be on track for something entirely different now. Ecologists have largely moved toward the idea of multiple stable states instead, where a site can end up in more than one possible configuration depending on chance events and the timing of disturbances.
Get the Full Details

Practical implications if you're managing land
If you are trying to restore a site or manage succession intentionally, the useful takeaway is that early interventions matter far more than anything you do after year five. The species that establish in the first three years tend to lock in the trajectory through competitive dominance or soil modification. I have seen sites where a single non-native forb took over in year one and effectively blocked establishment of the target native community for the next decade. Removing it after that point is expensive and often ineffective because the soil microbial community has adapted to the invader. A real constraint most people run into is the seed source. Not every site is near an intact natural community that can supply seeds through wind or animal dispersal. At my old work sites, we were often five to ten miles from the nearest remnant old-growth patch. That distance matters because most herbaceous pioneer seeds don't travel that far on their own. You either have to accept that the initial community will be largely colonized by widespread generalist species, or you have to actively seed or transplant, which drives up costs substantially. Active restoration typically costs between eight thousand and twenty thousand dollars per hectare depending on how degraded the starting conditions are, whereas passive restoration costs almost nothing but can take significantly longer and may not reach the target community at all.
When succession modeling fails completely
The biggest limitation is scale mismatch. Succession theory is built on local and landscape-level observations over decades, but management decisions often happen on seasonal budget cycles. When you try to use succession frameworks to justify short-term interventions, the predictions become unreliable because the underlying assumptions about disturbance frequency and intensity are wrong. This is especially true in fire-adapted ecosystems where the natural disturbance regime has been disrupted by suppression policies or climate change. You cannot apply classic seral stage progression to a system where the fire return interval has shifted from every five to ten years to every twenty to thirty years, or where drought is changing what survives the fire in the first place. There is also the issue of novel ecosystems. Human-altered landscapes often assemble species combinations that have no historical precedent. A site might end up with a mix of invasive grasses, scattered native shrubs, and opportunistic trees that simply never co-occurred before. Succession models do not handle this well because they assume a closed species pool from the surrounding region. When that assumption breaks, you are essentially watching an unscripted process and the old frameworks provide limited guidance. If you want to understand succession beyond the basics, the best approach is to pick a specific ecosystem type and track it over time rather than trying to generalize across all biomes. The patterns differ enough between a temperate deciduous forest, a tropical rainforest, and an alpine tundra that cross-biome comparisons often obscure more than they reveal. The fundamental mechanism is consistent, but the players and the pace are not.