What Actually Happens When a Species Splits Without Mountains or Oceans
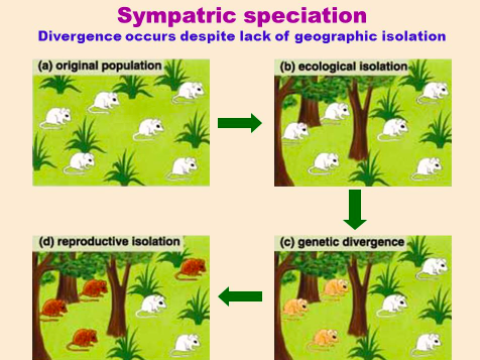
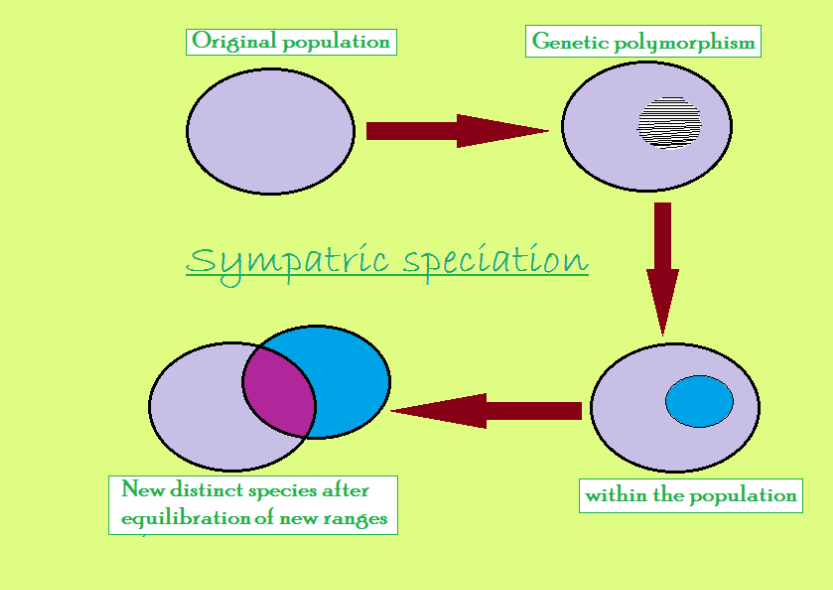
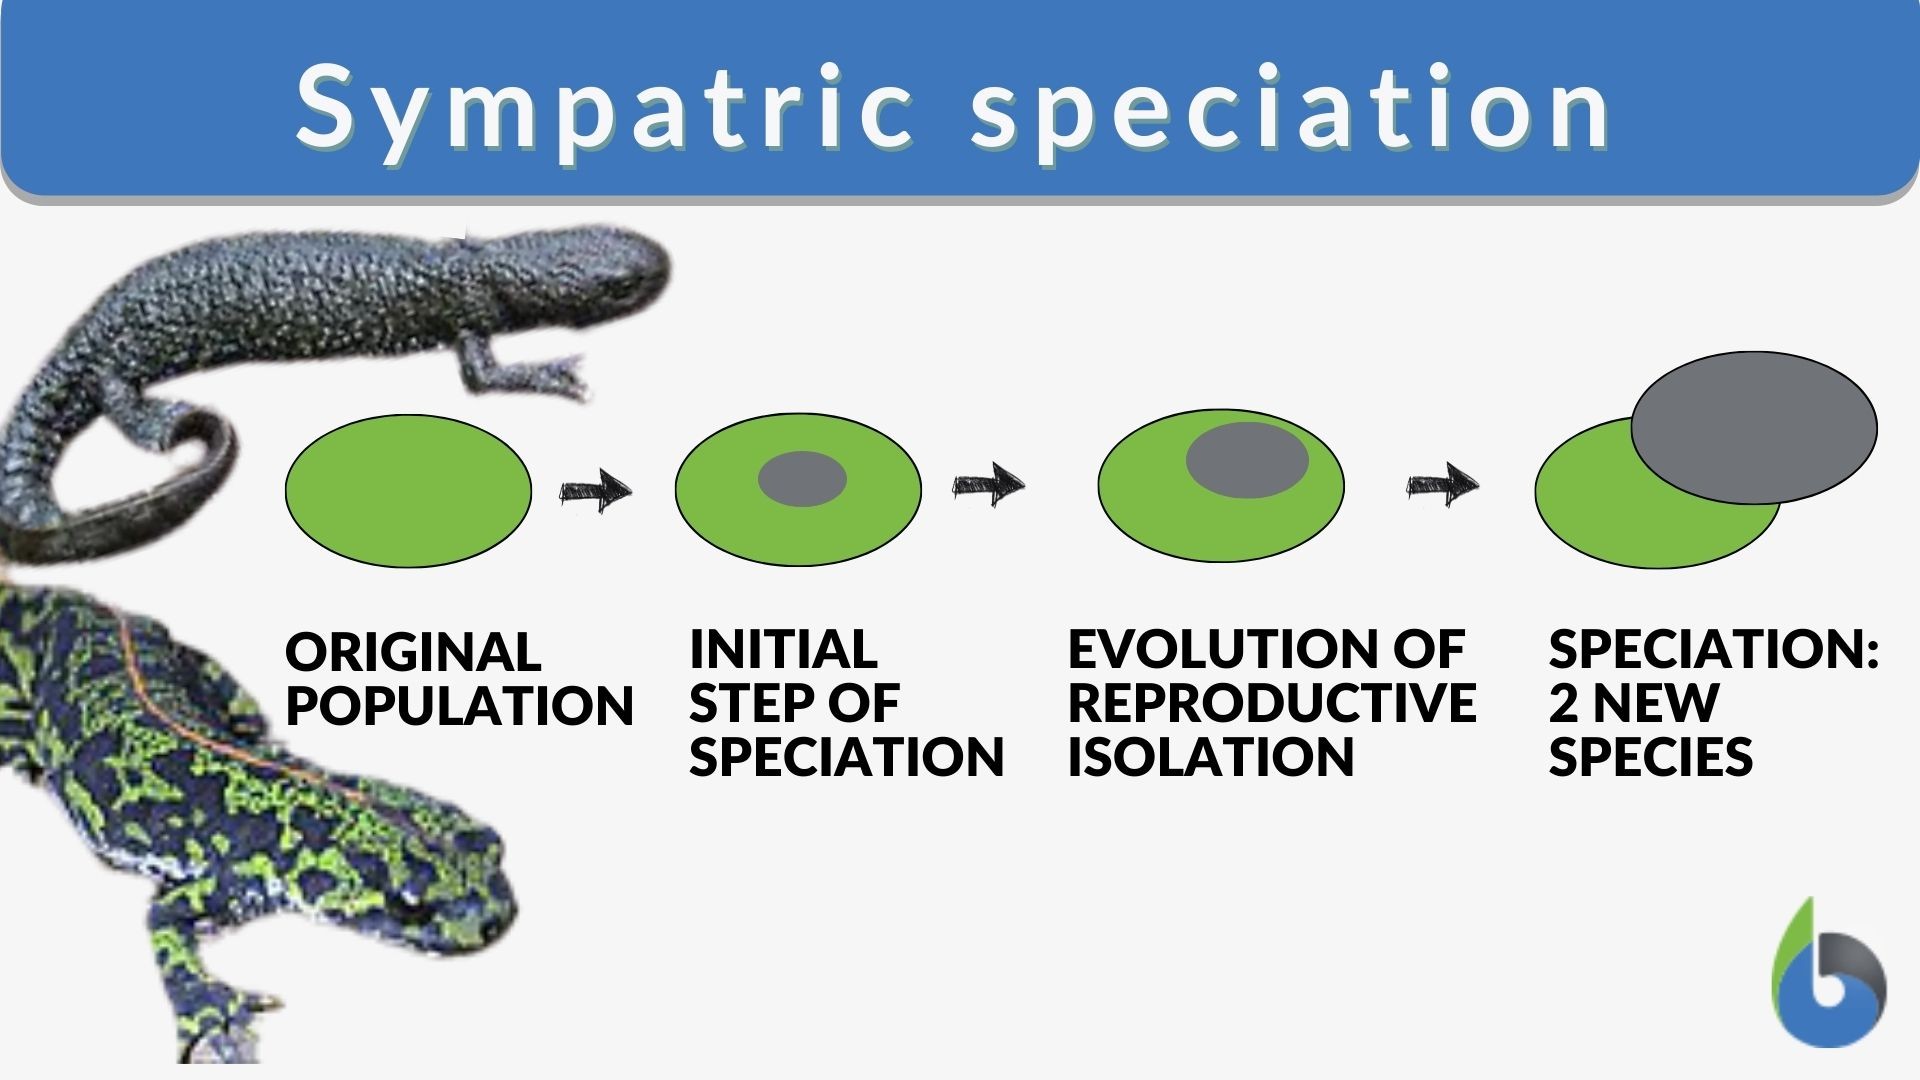
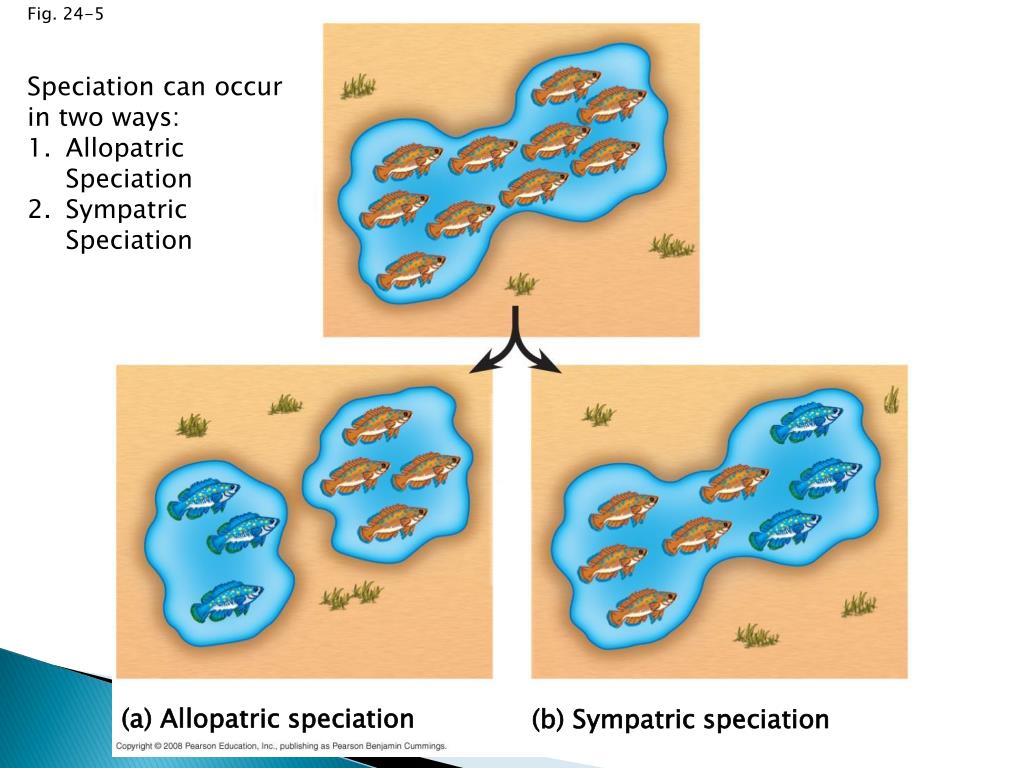
Sympatric speciation is the process where a new species evolves from an existing one while occupying the same geographic region. No physical barriers. No rivers shifting course. No island formation. Just pure reproductive isolation emerging from within a single population. It sounds counterintuitive because most introductory biology courses spend more time on allopatric speciation, but the mechanism is well documented and, honestly, more common than people give it credit for. The core mechanism comes down to reproductive isolation without geographic separation. A subset of a population stops interbreeding with the rest, and over time genetic divergence solidifies into a hard barrier. The most reliable pathway is polyploidy, particularly in plants. An error during meiosis doubles the chromosome count, and suddenly those individuals can't produce viable offspring with the original population. It happens in a single generation. That's not gradual. That's instant speciation on a chromosomal level. There's also ecological speciation, where subpopulations adapt to different niches within the same area. Aphids that switch from one host plant to another is a textbook case. The ones on the new plant mate at a different time of year because their life cycle is tied to the host plant's phenology. Over enough generations, the two groups stop exchanging genes even though they're living yards apart from each other.
Then there's sexual selection. If a subset of a population starts preferring a different mating signal, you can get divergence through mate choice alone. Some cichlid fish in African lakes show this pretty clearly, though I'd argue the lake depth gradients complicate the purely sympatric interpretation. The debate over whether some of those cases are truly sympatric or just parapatric with very narrow contact zones is still ongoing in the literature.
The Practical Side of Identifying Sympatric Speciation
Here's where it gets messy in practice. Distinguishing sympatric speciation from allopatric or parapatric scenarios requires careful geographic and genetic data. I've spent more time than I want to admit untangling cases where someone claimed sympatry but the populations had actually been separated by a habitat fragment during a past climatic shift. The genetic signature can look nearly identical. The workaround I settled on was combining coalescent-based demographic modeling with fine-scale spatial sampling. You need to test whether the divergence is older than the landscape feature that would have caused isolation, or if it's genuinely contemporaneous with the current habitat structure. Programs like DIYABC or fastsimcoal2 let you fit alternative demographic scenarios and compare their likelihoods. Without that step, you're mostly making an educated guess. A specific problem I ran into involved a group of threespine stickleback in a set of connected British Columbia lakes. The surface data suggested sympatry because the lakes were hydrologically linked and fish moved between them during spawning season. But the genetic data showed deep divergence that didn't match the dispersal pattern. It turned out the lakes had been isolated during the last glacial maximum, and the postglacial reflood created the appearance of sympatry. The "sympatric" ecotypes were actually relict divergent lineages that happened to end up in the same drainage. This kind of misattribution is probably the single most common error in the field.
Get the Full Details
Counter-Intuitive Things People Get Wrong
First, polyploidy isn't limited to plants. There are documented cases in amphibians and fish, though they're far rarer. When they do occur, the mechanism is identical. Chromosome doubling creates an immediate reproductive barrier. The resulting organism is effectively a new species the moment it forms, not after thousands of years of divergence. Second, sympatric speciation doesn't require a strong initial barrier. Weak disruptive selection can kickstart the process, and then assortative mating reinforces it. This reinforcement phase is what turns a partial split into a complete one. The initial niche differentiation might be slight, but once mating becomes tied to that niche, gene flow drops precipitously. You don't need a massive ecological difference to begin with. The biggest pitfall beginners encounter is assuming that observed sympatry equals sympatric speciation. Two species living in the same area now doesn't mean they speciated in that area. They could have arrived there separately. Always check the phylogeographic history before drawing conclusions about the speciation mode.
Limitations and Where This Framework Breaks Down
Sympatric speciation is genuinely harder to prove than allopatric speciation because you're trying to demonstrate the absence of a barrier rather than the presence of one. Absence of evidence is not evidence of absence, and the same logic applies here. You can never definitively rule out a historical geographic barrier, especially in taxa with good dispersal ability where range shifts over geological time are common. The method also struggles with recently diverged species pairs. When divergence is incomplete, gene flow may still be occurring at low levels, and the statistical power to distinguish sympatric from parapatric models drops significantly. I usually tell people that if you're working with species that diverged less than 500,000 years ago, treat any sympatric speciation claim as provisional unless you have exceptionally dense sampling. For organisms where polyploidy isn't a mechanism and ecological niches are hard to define, the whole framework becomes much less useful. In many animal groups, especially mobile vertebrates, the default assumption should lean toward allopatric or peripatric models until strong evidence points elsewhere. The burden of proof is genuinely higher here, and the literature reflects that with more skepticism toward sympatric claims in animals than in plants.
If your system doesn't have clear ecological divergence or chromosome-level data, consider shifting to a speciation-with-gene-flow model instead. It's more honest about what the data can actually support and gives you parameter estimates for the amount and timing of gene flow rather than forcing a binary sympatric versus allopatric answer that the data might not resolve.