The Cell Question Nobody Asks Straight
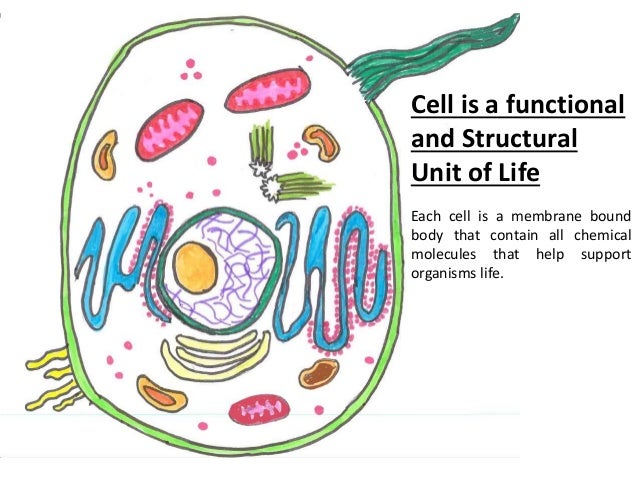
When you open a biology textbook it will tell you the cell is the basic unit of life. That is technically true and completely unhelpful if you have ever actually looked at a prepared slide of onion root tip or tried to explain why mycoplasma makes you want to throw your microscope across the lab. The question sounds simple but it sits in a zone where every definition immediately encounters something that refuses to behave. A cell is a membrane-enclosed system that can metabolize, replicate its information, and respond to its environment without stealing that work from something else. That is the working definition I use when I am grading undergraduate labs and trying not to lose my mind over edge cases. The membrane matters because without a boundary you do not have homeostasis and without homeostasis you do not have a system that stays alive when the beaker temperature drifts. Replication matters because a collection of molecules that cannot make copies of itself is chemistry, not biology. Metabolism matters because you cannot sustain order without energy flow and someone trying to run a cell purely on passive diffusion will watch their gradients collapse in about four minutes depending on surface area to volume ratio. The moment you accept that definition you still have to deal with organelles that think they are independent. Mitochondria have their own circular DNA, their own ribosomes that resemble bacterial ones, and they divide by binary fission inside the cytoplasm while the nuclear genome sits there doing its own thing. Chloroplasts do the same in plants. Endosymbiont theory explains this historically but it does not change the laboratory reality that you can sometimes detect residual protein import machinery that still runs on signals encoded outside the organelle. If you isolate mitochondria from a liver cell and drop them into a buffer with the right substrates they will keep respiring for a while, but they cannot replace the cell. They cannot rebuild their own membranes from scratch because most of the lipid synthesis genes moved to the nucleus over hundreds of millions of years. That is why the cell remains the operational unit even when its power plants pretend otherwise.
Viruses, Prions, and the Definition That Breaks
Everyone brings up viruses and nobody answers it cleanly. A virion is a packaged set of nucleic acids wrapped in protein, sometimes with a lipid envelope stolen from a host membrane. It does not metabolize. It does not grow. It does not replicate on its own. When you mix tobacco mosaic virus with a leaf extract you get no new particles until a functional ribosome shows up and starts translating the viral mRNA. In that gap between particle and active infection the virion sits in a gray area that taxonomists handle by saying it is not alive and biologists handle by studying it like it is alive because the behavior is indistinguishable once it engages a host. Prions are worse for your sense of boundaries. They are misfolded proteins that recruit normal copies of the same protein into the misfolded conformation. There is no nucleic acid involved in the propagation mechanism. You can transmit a conformational state between proteins the way you can transmit a rumor through a room, except the rumor folds the listeners wrong. From a strict definition standpoint prions are not units of life, but they are units of biological information transfer and they cause disease in mammals at concentrations that defeat conventional sterilization. Autoclaving at 121 degrees for 15 minutes works if you also combine it with strong alkali and extended exposure. Standard lab protocols assume autoclave alone is sufficient and then somebody runs a Western blot six months later and wonders why the signal is still there.
Artificial Cells and the Experiment That Teaches You More
Creating a protocell in a teaching lab usually starts with lipids, water, and something that generates an osmotic gradient. You can buy preformed liposomes or make your own from egg lecithin and a bit of cholesterol if you need membrane fluidity at room temperature. The moment you add an energy source like a proton gradient generator or a simple ATP analog you can sometimes drive transport across the bilayer. What you cannot do is make it self-replicate without a template and a polymerase and a whole metabolic scaffold that took billions of years to evolve. I ran a version of this with undergraduate students a few years ago and we spent three weeks trying to get encapsulated ribozymes to catalyze their own replication inside growing vesicles. The problem was not the chemistry, it was the membrane. Every time the internal reaction produced enough polymer to notice, the osmotic pressure spiked and the vesicle either burst or shrank to a point where the reactants could no longer diffuse past the bilayer. The workaround was to add a small fraction of amphiphilic peptides that increased membrane flexibility without compromising the barrier function. It was not elegant but it kept the vesicles intact long enough for the reaction to proceed for several hours. That told us more about why natural cells invest heavily in membrane repair and cytoskeletal support than any textbook diagram ever did.
Get the Full Details
Specialized Cases That Refuse to Fit
Synthetic minimal cells like those built by Craig Venter's group required you to transplant a complete genome into a recipient cell whose original genome you had removed. The result was a cell that could grow and divide but only because you had copied an existing self-replicating system into a compatible chassis. You did not create life from non-life. You copied life into a new container and hoped the container accepted the new manager. The experiment proved that the basic unit of life can be reconstructed when you start from a working version, but it did not solve the origin problem or give you a shortcut to generating a unit from scratch. Multicellular organisms add another layer. A single neuron or a hepatocyte removed from the body cannot survive on its own for long. It lacks the circulatory input, the hormonal signaling, the waste removal. Yet it still meets the definition of a cell and it still carries the full genome. Developmental biology shows that specialization comes from gene regulation, not from losing genetic information. A skin cell and a neuron have the same DNA but different expression profiles. The unit of life remains the cell, but the functional unit of an organism is often a tissue or an organ system that coordinates multiple cells through signaling networks.
Why the Question Still Matters
Defining the basic unit of life is not just academic trivia. It shapes how you approach synthetic biology, how you design containment protocols for engineered organisms, how you evaluate whether a discovery is truly novel or just a variation on an existing mechanism. If you believe the cell is the unit and nothing below it qualifies, you will invest in whole-cell platforms. If you believe functional subsystems can be portable, you will explore cell-free expression systems and modular biobricks. Both approaches have value and both hit hard limits when you try to scale them. The practical takeaway is that the cell is the smallest system that can maintain itself, replicate, and adapt without external rescue, given the right raw materials. Everything else is either a component of that system, a parasitic dependency, or an experimental artifact that looks alive until you remove the host. That boundary is fuzzy but it is real enough to build on, and it is where most of the interesting work happens whether you are running a lab or just trying to understand why your cultures keep dying on Tuesdays.