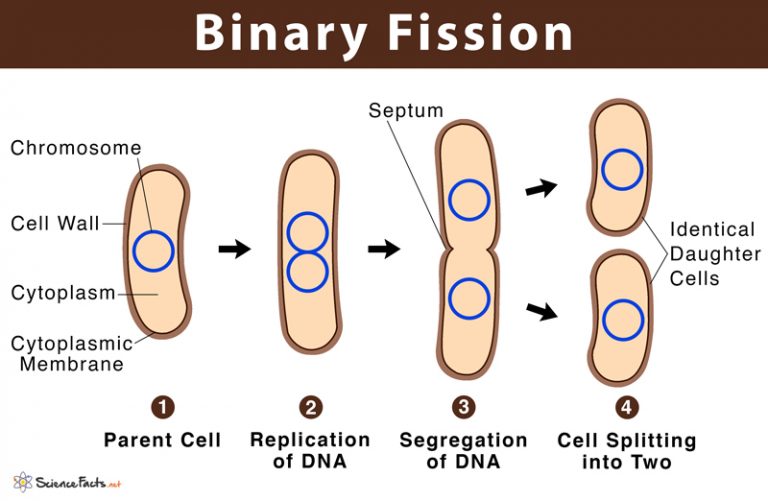
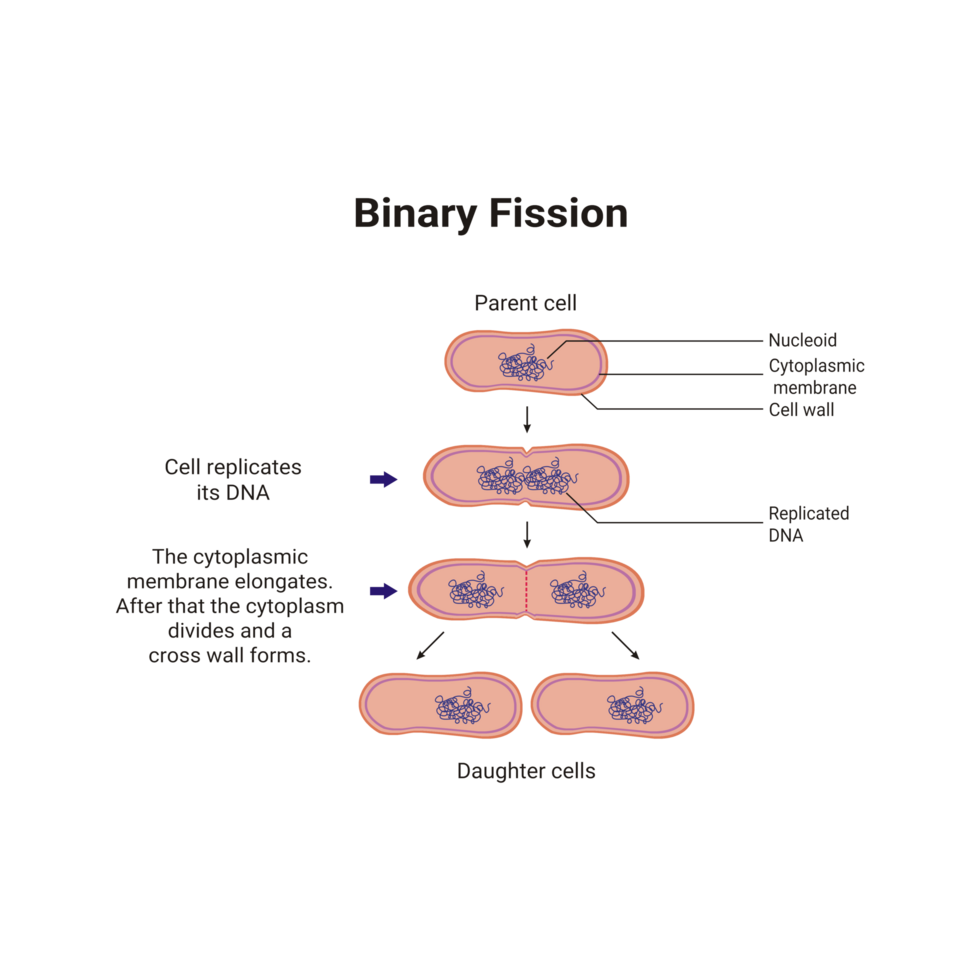
Binary fission is the primary method of asexual reproduction in bacteria and archaea. A single parent cell replicates its genetic material and then divides into two roughly equal daughter cells. It is mechanically simple compared to euk Mitosis and eukaryotic cell division. The core process involves three main steps. First, the circular chromosome is replicated. Second, the cell elongates and the two copies of the chromosome move to opposite ends. Third, a septum forms down the middle and the cell physically splits into two.
I spent years growing bacteria in a clinical lab, and watching binary fission under a microscope is straightforward once you understand the timeframes involved. A culture of Escherichia coli in rich media at 37 degrees Celsius can complete a full division cycle in about twenty minutes. Under less favorable conditions, that same organism might take two to three hours. The difference comes down to nutrient availability, temperature, and pH.
What Is The Binary Fission Process
The mechanism begins at a specific origin of replication on the bacterial chromosome. A protein called DnaA binds to this origin and unwinds the DNA helix. Replication proceeds bidirectionally around the circular chromosome until the two replication forks meet at the termination region opposite the origin. The result is two identical copies of the genome, each still attached to the cell membrane at different points.
Once the chromosomes are separated, the cell starts building a new cell wall and membrane between them. This construction is directed by a protein complex called the divisome. The key structural component is FtsZ, a GTPase that assembles into a ring at the future division site. This Z-ring recruits other proteins that synthesize peptidoglycan and constrict the cell membrane inward. The process continues until the septum is complete and the two daughter cells separate.
Most introductory textbooks present this as a clean, uniform process. In reality it is much messier and more variable than that. I ran into a problem once where my cultures of Pseudomonas aeruginosa were dividing extremely slowly despite appearing healthy under the microscope. The problem was not the organism itself but the plasmid I had introduced. The plasmid carried an antibiotic resistance gene and added significant metabolic burden. Every time I removed the antibiotic selection pressure to study the bacteria without it, the plasmid-free variants rapidly outcompeted the plasmid-containing cells because they reproduced faster. This is a well-documented issue in molecular microbiology called plasmid instability, and it is something you need to plan around if you are working with recombinant strains.
The generation time or doubling time is the metric that matters most when you are actually using this knowledge in a lab. Generation times vary enormously across species. Some deep-sea archaea divide once per year. Most common pathogens fall in the one to three hour range. E. coli and Salmonella enterica can hit twenty minutes under optimal conditions. This variation exists because the replication machinery, ribosome density, and metabolic rate all differ between organisms.
You should also understand that not all bacterial reproduction follows strict binary fission. Some species undergo budding where a small protrusion forms and eventually separates. Others do multiple fission and produce several smaller cells at once. Mycobacterium tuberculosis divides by a form of binary fission that is notably slower and more asymmetric than what you see in E. coli. The cell envelope of mycobacteria contains mycolic acids, making the septum construction more complex and the division cycle longer.
Conjugation is frequently confused with binary fission by people new to microbiology. It is not. Conjugation transfers genetic material between cells through direct contact via a pilus. No new cells are produced. Binary fission produces new individuals. These are fundamentally different processes.
Another thing that trips people up is the relationship between binary fission and endospore formation. Endospores are survival structures formed by certain genera like Bacillus and Clostridium. The sporulation process is not a reproductive mechanism. One vegetative cell produces one endospore. When the spore germinates, it returns to one vegetative cell. There is no increase in cell number. The cell still reproduces through binary fission when conditions improve.
I also encountered a practical limitation with binary fission that is easy to overlook if you are only working with petri dishes. When you culture bacteria in a liquid medium, the population does not grow exponentially forever. After the exponential phase, the culture enters stationary phase because nutrients are depleted and waste products accumulate. At that point, binary fission slows or stops entirely. Some cells may even lyse. This is why serial dilution is necessary if you want to measure viable cell counts beyond the exponential phase. Simply counting cells under a microscope without accounting for dead cells will give you inflated numbers.
Quorum sensing adds another layer of complexity. Bacteria release signaling molecules called autoinducers into their environment. As the population density increases, the concentration of these molecules rises. Once a threshold is reached, gene expression changes across the population. This can trigger biofilm formation, virulence factor production, or even the inhibition of further division in some species. The implication is that binary fission in natural environments is tightly regulated by population density, not just by nutrient availability. A lab culture in a shaking flask behaves differently from the same organism growing on a tissue surface in a host.
The molecular regulation of the division cycle is another area where textbooks oversimplify. The nucleoid occlusion system prevents the Z-ring from forming over unsegregated DNA. If the ring forms too early, it can slice through a chromosome and kill both daughter cells. The Min protein system in E. coli prevents Z-ring assembly at the cell poles by oscillating from pole to pole and keeping the concentration of MinC and MinD low at the midcell. Mutants lacking functional Min proteins form septa at the poles and produce minicells that lack chromosomal DNA. This is a real laboratory strain that is still used for plasmid prep because the minicells are enriched for plasmid DNA.
If you are working in a lab and need to ensure uniform division across a culture, maintaining logarithmic phase growth is essential. This requires regular subculturing into fresh medium at the right dilution factor. The typical approach is to inoculate a fresh culture at a density of one percent into fresh broth. The exact timing depends on your target generation time and the volume of your culture. Overcrowding a culture and then shifting it into fresh medium without accounting for the lag phase will give you uneven growth curves and unreliable experimental results.
Gallery What Is The Binary Fission
Binary Fission | Biology cell division, What is genetic engineering in ...
What Is Binary Fission In Bacteria
Explain The Process Of Binary Fission With Diagram Lesson Explainer:
Explain The Process Of Binary Fission With Diagram
Binary fission process of cell reproduction in the division stages ...