The Calvin Cycle Doesn't Start Where People Think It Starts
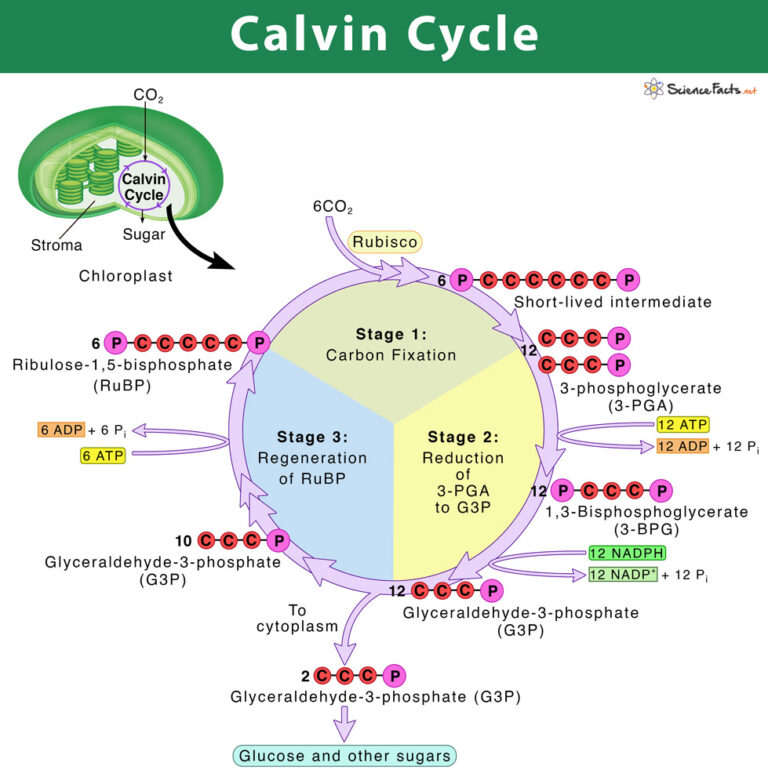
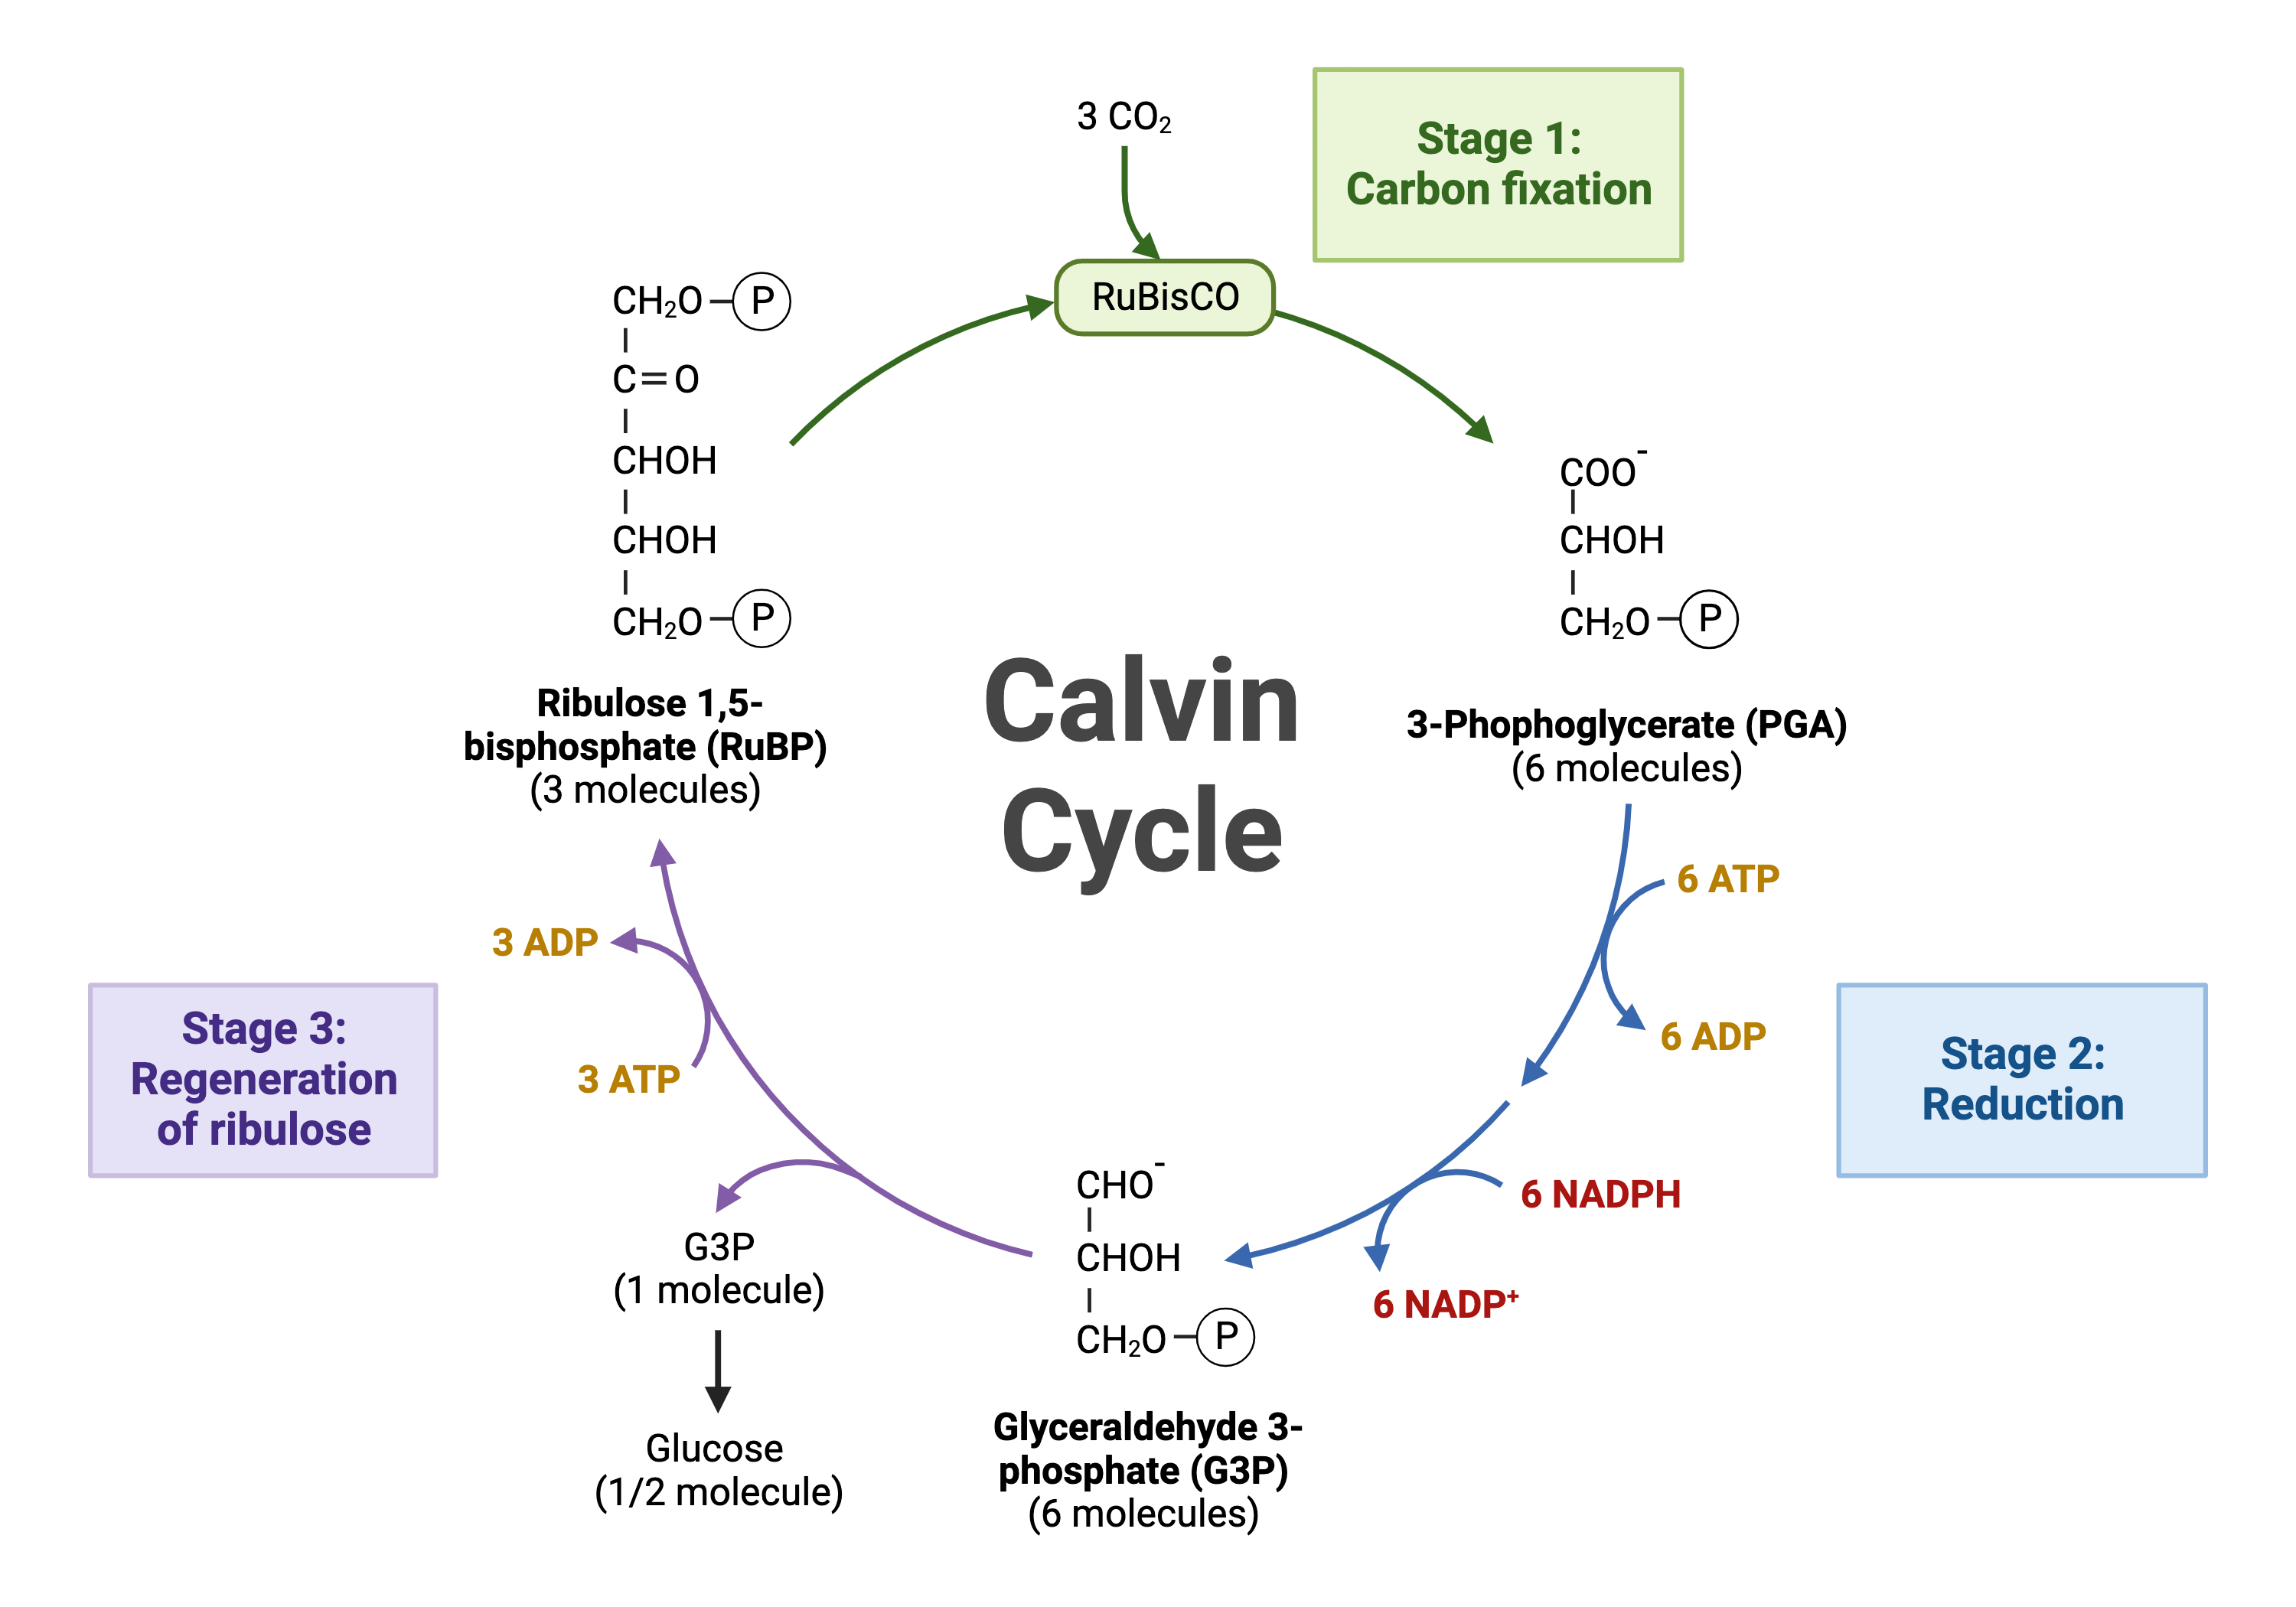
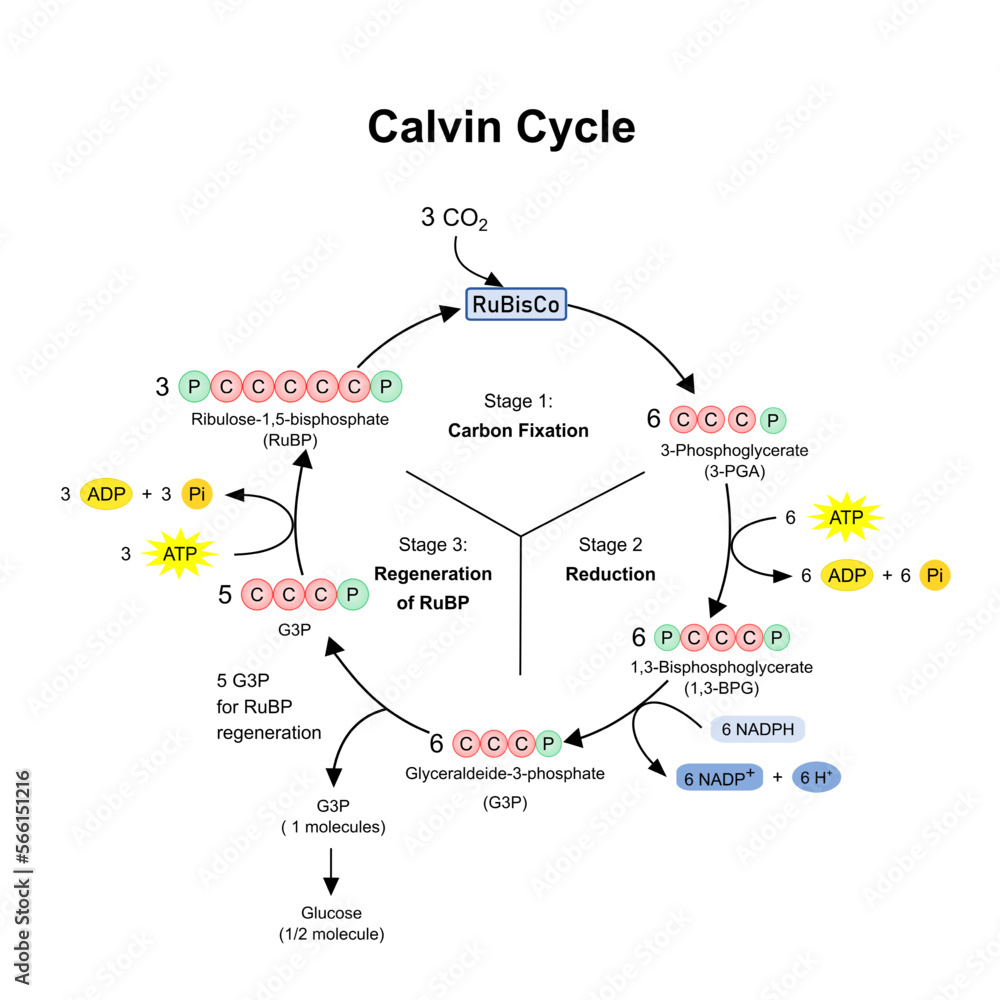
Most textbooks open the Calvin cycle chapter with a diagram showing three phases: fixation, reduction, regeneration. That's correct but misleading. The cycle actually lives inside the stroma of the chloroplast, and the real story isn't what happens inside it but how tightly it's coupled to everything else around it. Light reactions supply the ATP and NADPH. Without those, the cycle stops within seconds. I've seen students treat it like an isolated pathway, which is why they miss the regulatory connections. The core mechanism is straightforward enough. Ribulose-1,5-bisphosphate (RuBP) grabs a molecule of CO through the enzyme RuBisCO. This produces two molecules of 3-phosphoglycerate (3-PGA). ATP phosphorylates those, NADPH reduces them into glyceraldehyde-3-phosphate (G3P). Some G3P exits the cycle to make glucose and other carbohydrates. The rest recycles back into RuBP through a series of reactions that consume more ATP. For every three CO fixed, one G3P is net produced. It takes six turns to make one net glucose molecule.
What Is The Calvin Cycle
At its simplest, the Calvin cycle is the set of light-independent reactions that convert atmospheric CO into carbohydrate using energy from the light reactions. It runs in the stroma. It operates continuously during daylight as long as ATP and NADPH are being supplied. It does not directly use light, but it will shut down almost immediately if light stops, because the substrates it depends on run out fast. Here's something most introductory courses gloss over: RuBisCO is arguably the worst enzyme in existence. It's slow, it's abundant, and it makes mistakes. The enzyme can bind O instead of CO, which kicks off photorespiration. Photorespiration burns ATP and releases previously fixed carbon. It's a massive efficiency hit, especially in hot, dry conditions where stomata close and O accumulates inside the leaf. C and CAM plants evolved workarounds for this problem by spatially or temporally separating initial CO capture from the Calvin cycle itself. If you're studying plant physiology without understanding why photorespiration matters, you're missing the reason the Calvin cycle exists in the form it does. I ran into this exact issue once while working on a greenhouse experiment. We were growing spinach under controlled environmental chambers and noticed carbon fixation rates dropping far below model predictions, even though light and temperature were optimal. The issue was that the CO concentration in the chamber wasn't being refreshed properly. RuBisCO was essentially running out of substrate because the air wasn't circulating. We installed a small fan and supplemented with CO enrichment at 800 ppm. Fixation rates jumped by roughly 40 percent within two days. The Calvin cycle works fine when you give it what it needs. It fails quietly when you don't.
The regeneration phase is where things get complicated. The cycle involves a dozen intermediate compounds, including sugars with three, four, five, six, and seven carbons. Transketolase and aldolase shuffle carbon skeletons around. Phosphatases remove phosphate groups. Kinases add them back. If you're tracking this on paper, it looks like a mess. In practice, it's a self-sustaining loop that only needs a small input of ATP to keep turning. The key regulatory step is the regeneration of RuBP. If that slows down, the entire cycle backs up. Another thing beginners miss: the Calvin cycle is regulated by light, even though it doesn't use light directly. The enzyme fructose-1,6-bisphosphatase, along with several others in the cycle, is activated by the ferredoxin-thioredoxin system. When light hits the photosystems, electrons flow through ferredoxin, which reduces thioredoxin, which in turn reduces disulfide bonds in the Calvin cycle enzymes. They switch from a low-activity state to a high-activity state. At night, the enzymes oxidize and slow down. So the cycle is effectively gated by light through a redox cascade, not through direct photon capture. The cycle also has a pH and magnesium gradient dependence. The stroma becomes more alkaline and accumulates Mg² ions when the light reactions are active, because protons are pumped into the thylakoid lumen. RuBisCO and several other Calvin cycle enzymes have optimal activity at the higher pH and Mg² concentrations found in illuminated chloroplasts. This is another reason the cycle stalls in the dark. It's not just about running out of ATP and NADPH. The enzyme environments themselves change.
Get the Full Details
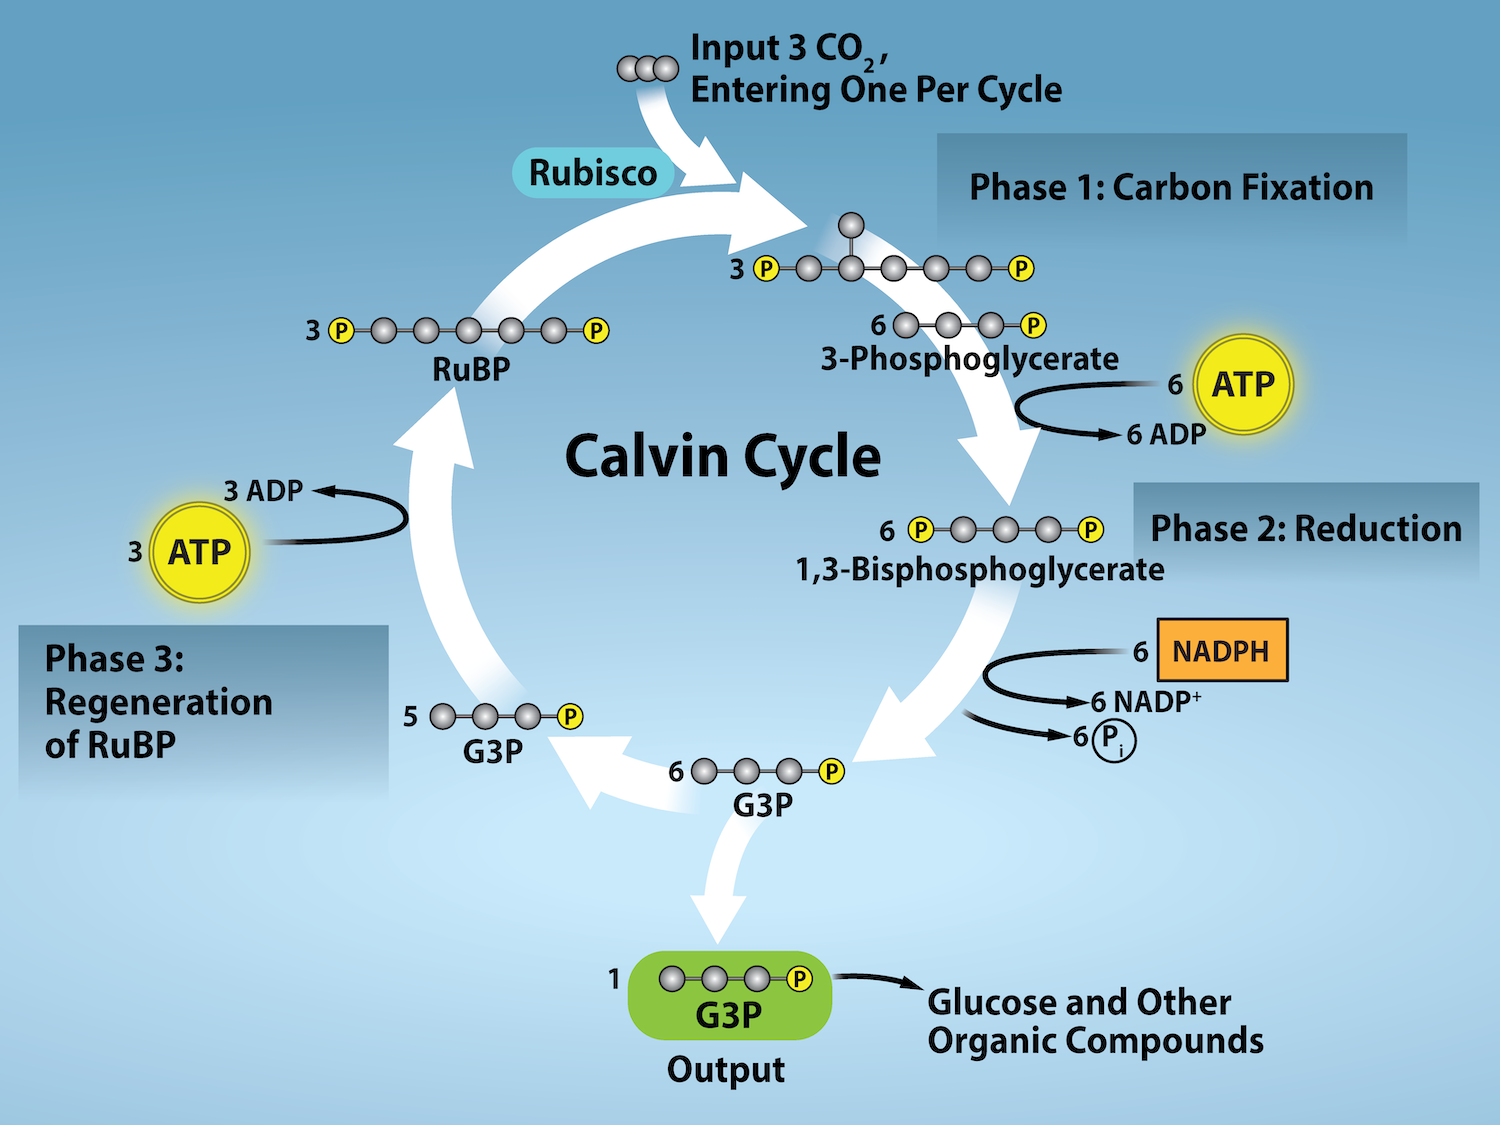
One practical limitation worth noting: the Calvin cycle is the rate-limiting step in most photosynthetic organisms under normal conditions. That means efforts to increase crop yield through genetic engineering often target RuBisCO or the surrounding regulatory machinery. So far, results have been modest. RuBisCO's catalytic rate is around 3 turnovers per second, which sounds terrible compared to other enzymes that do thousands. Improving it hasn't worked out well because the enzyme's specificity trade-off is baked into its structure. Speed and selectivity pull in opposite directions. Engineering a faster RuBisCO tends to make it worse at distinguishing CO from O, which just increases photorespiration. Some researchers are exploring alternative CO-concentrating mechanisms or swapping in bacterial RuBisCO variants, but nothing has scaled to agriculture yet. If you're trying to memorize this for an exam, don't try to memorize every intermediate. Focus on the inputs and outputs. Three CO enter. Nine ATP and six NADPH are consumed. One G3P exits. Five G3P recycle. Two G3P make one glucose. The rest is bookkeeping. The pathway itself is conserved across almost all photosynthetic organisms, from cyanobacteria to oak trees, which means the basics you learn in a first-year biology class are the actual basics, not a simplified cartoon.