How It Actually Works In The Lab
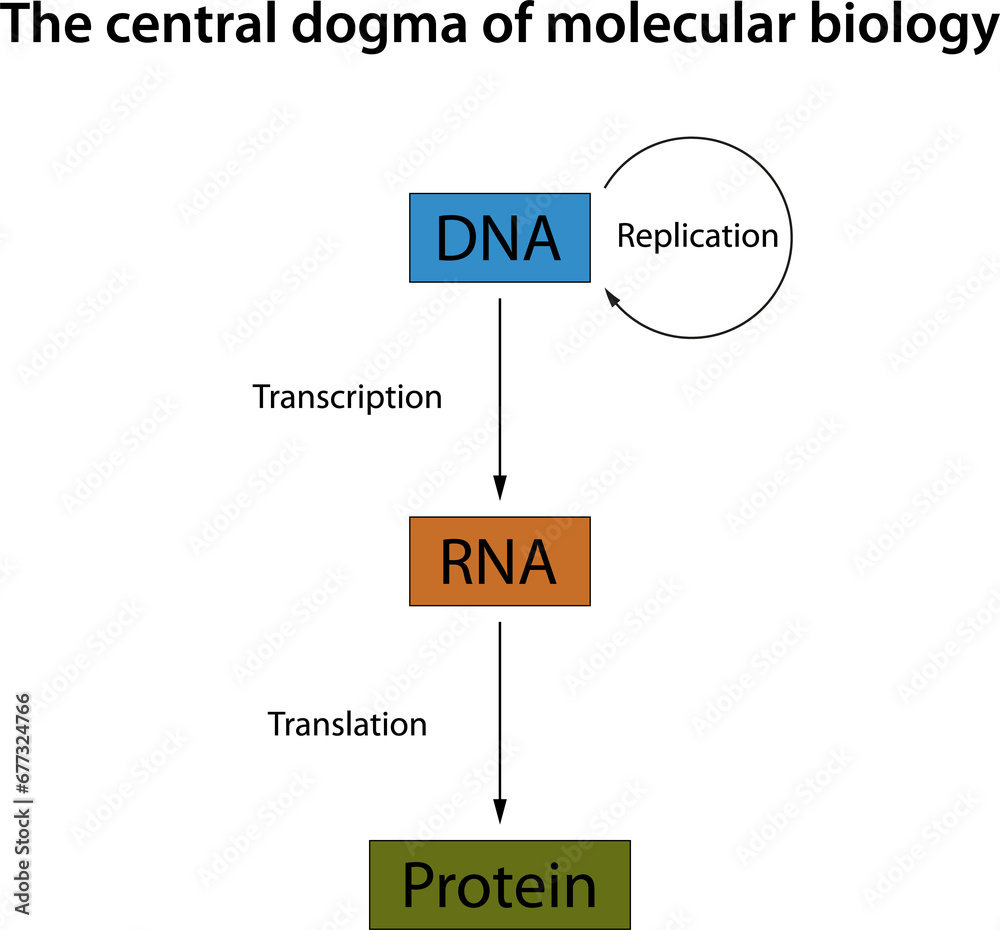
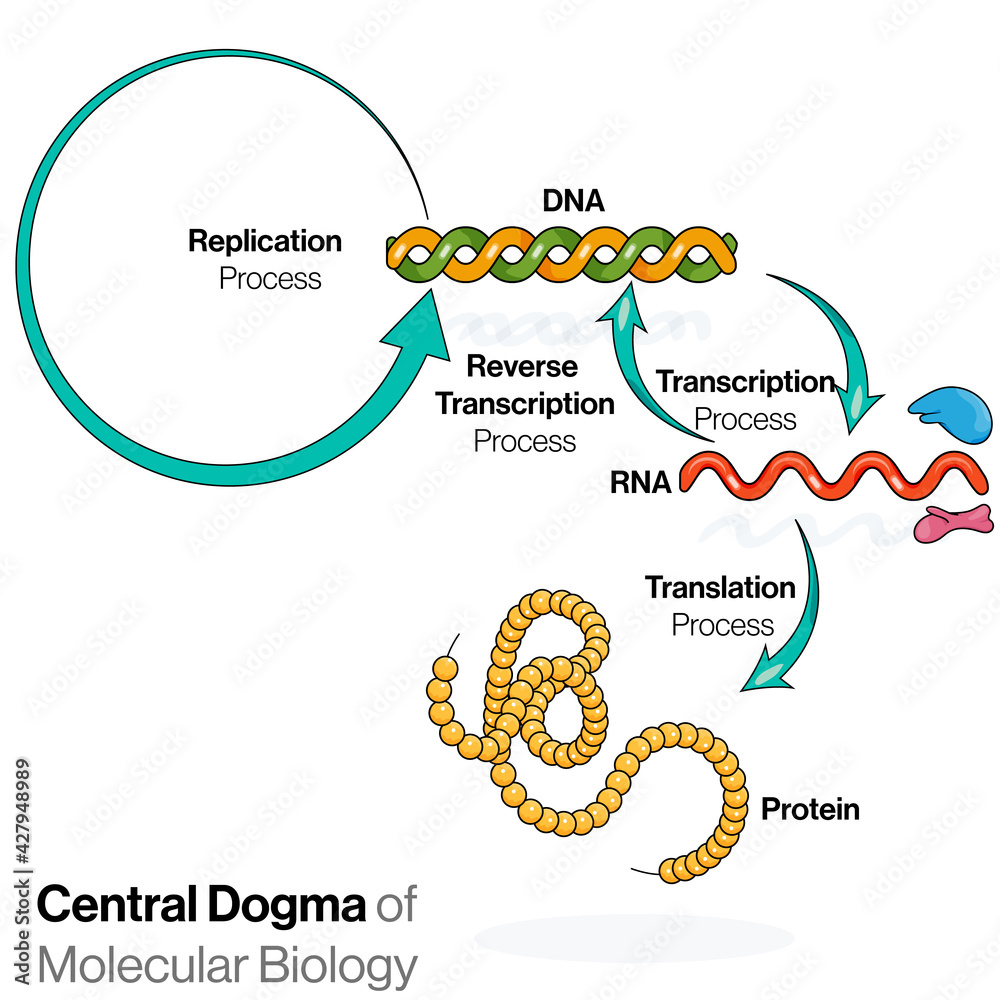
The central dogma describes how genetic information flows through a cell. DNA gets transcribed into RNA, and RNA gets translated into protein. That is the basic pipeline. Francis Crick proposed it in 1958, and it has held up better than most biological hypotheses over the decades. Most people learn it as a neat diagram with arrows pointing in one direction. Reality is messier than that diagram. It is the framework for understanding how the instructions stored in DNA become functional molecules in a cell. The DNA sequence of a gene is copied into messenger RNA by RNA polymerase. That mRNA then travels to a ribosome, where transfer RNAs read the codons and assemble amino acids into a polypeptide chain. The chain folds into a protein. That is the standard flow. DNA to RNA to protein. The standard flow works fine when you are doing textbook genetics. But the moment you start working with actual cell lines, you run into complications pretty quickly. I spent three weeks once trying to figure out why a recombinant protein I was expressing in E. coli was showing up as degraded fragments instead of full-length product. The plasmid sequence looked right. The primers checked out. The issue turned out to be a cryptic internal promoter in the insert that caused runaway transcription, creating antisense RNA that triggered RNA degradation pathways. The central dogma still applied, but the cell was using it against me in ways the textbook diagram never showed.
I ended up switching to a T7-based expression system with tighter promoter control and added a 5' UTR destabilizing element that shut down that aberrant transcription. The yield jumped from near zero to roughly 40 milligrams per liter of culture. It took me about two weeks of troubleshooting to get there, but that workaround is standard practice now for difficult systems. One thing beginners miss is that the central dogma is not a strict one-way street. Reverse transcription exists. RNA-dependent RNA polymerases exist in viruses and in some cellular contexts through RNA interference pathways. Telomerase is a ribonucleoprotein that uses an RNA template to extend DNA. These exceptions do not invalidate the dogma. They just mean the original formulation was intentionally narrow, and Crick himself clarified that it was meant to describe the general flow in normal cells, not every edge case in virology or retrotransposon biology. Another thing people gloss over is the regulatory layer between transcription and translation. Just because a gene is transcribed does not mean protein will be produced at proportional levels. Post-transcriptional modifications like alternative splicing, RNA editing, and microRNA-mediated repression can dramatically change the output. In my experience running qPCR and Western blots in parallel, the correlation between mRNA abundance and protein levels is often around 0.4 to 0.6 in mammalian cell lines. That means mRNA measurements alone can mislead you by a factor of two or three when you are trying to predict actual protein expression. If you need accurate protein quantification, measure the protein, not just the transcript.
The dogma also breaks down in prion biology, where the protein itself becomes the infectious information carrier without any nucleic acid involvement. That is a genuine exception that challenged the framework, though it is fairly rare. For almost everything else in molecular biology, the DNA-to-RNA-to-protein pipeline remains the dominant model for understanding cellular function. If you are designing an experiment around this, the practical takeaway is straightforward. Plan for the exceptions even if you are not studying them directly. Use proper controls for both transcriptional and translational regulation. And when your data do not match the expected flow, check for regulatory complications before questioning the central dogma itself. The dogma is not wrong. Your experimental conditions probably just introduced noise that the simple diagram does not account for.
Get the Full Details