The Equation Itself
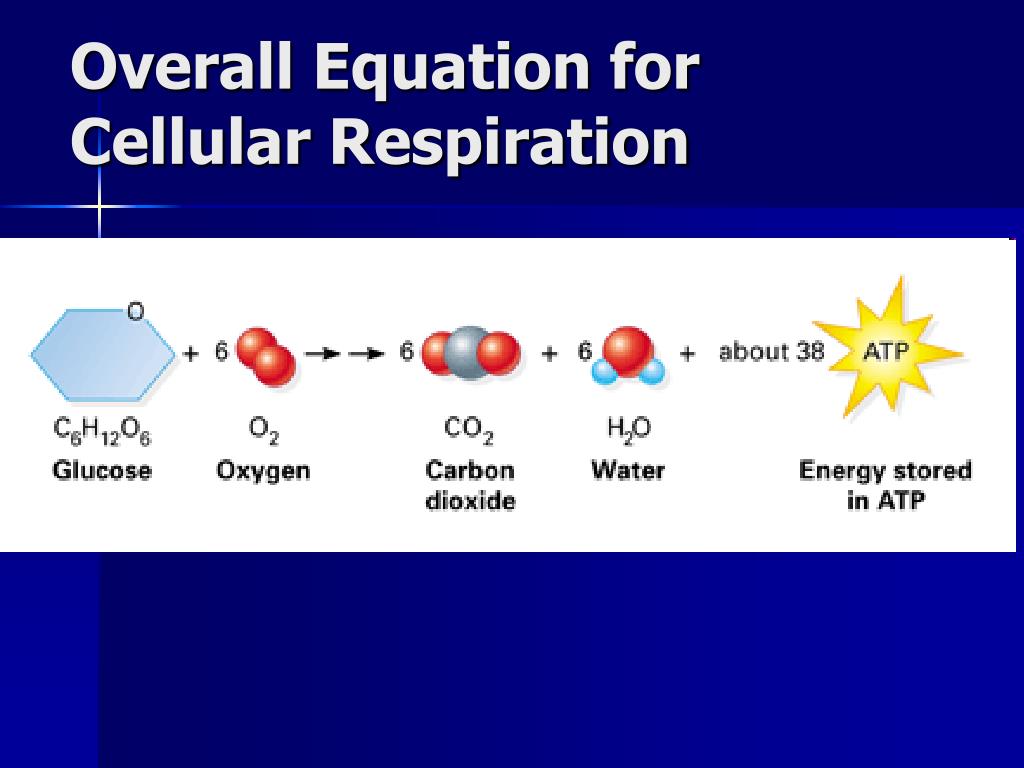
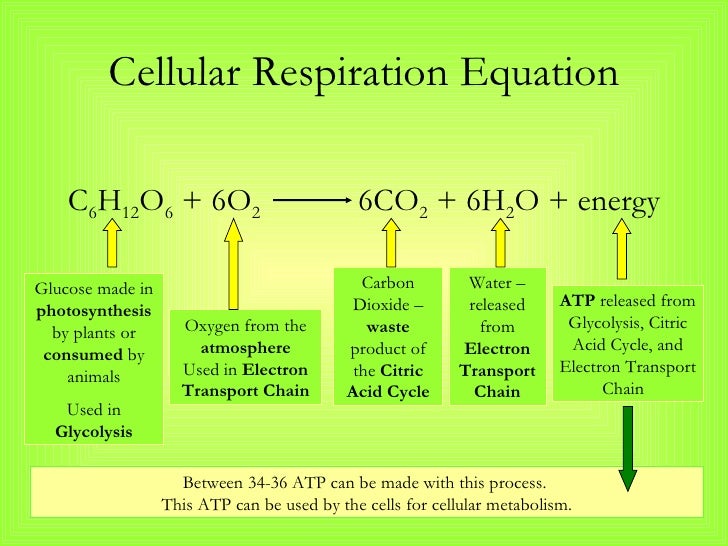
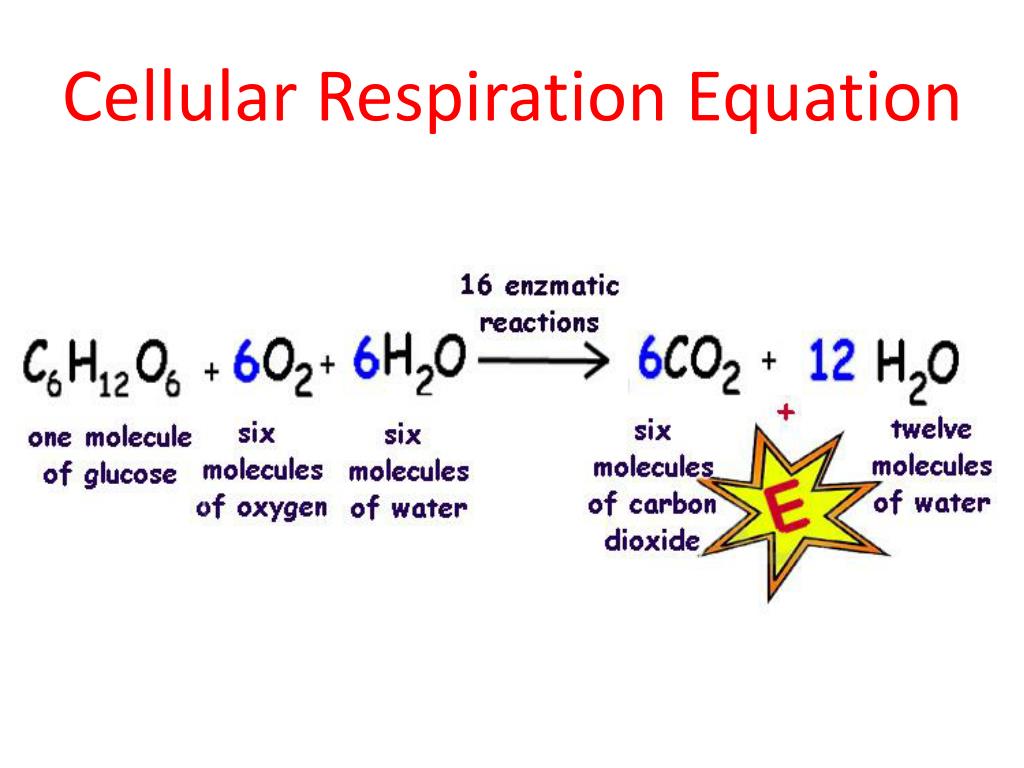
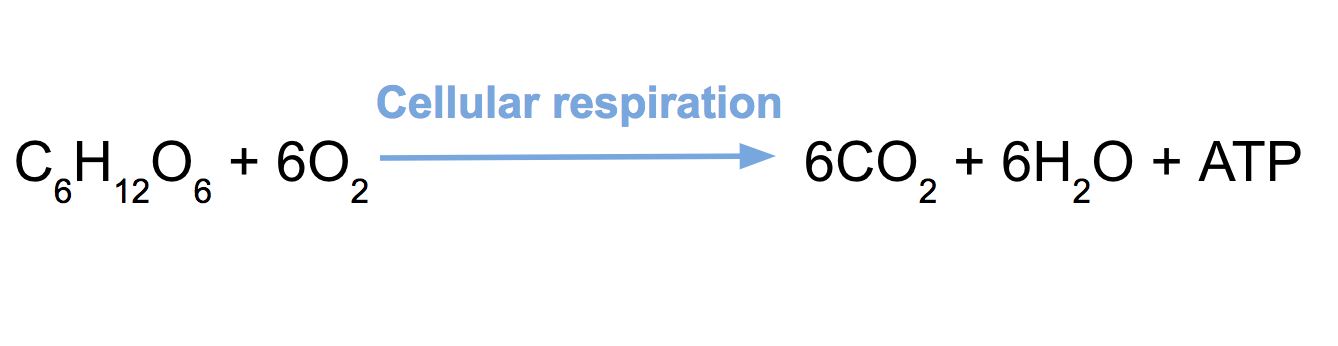
The standard balanced equation for aerobic cellular respiration is C6H12O6 + 6O2 6CO2 + 6H2O + energy (ATP). That's it. Six molecules of glucose react with six molecules of oxygen to produce six molecules of carbon dioxide, six molecules of water, and usable energy stored in ATP. The equation balances cleanly—6 carbons on each side, 12 hydrogens on each side, 18 oxygens on each side. There's also the anaerobic version, which runs through fermentation instead of the electron transport chain. In lactic acid fermentation, the equation simplifies to C6H12O6 2C3H6O3 + energy (2 ATP). In alcoholic fermentation, it's C6H12O6 2C2H5OH + 2CO2 + energy (2 ATP). Notice the dramatically lower ATP yield. This matters in practice because organisms running anaerobic pathways hit a wall fast.
What Is The Chemical Equation For Cellular Respiration
If you're trying to actually use this rather than just memorize it for a test, here's where things get interesting. The balanced equation you see in textbooks represents the net result of a process that involves dozens of individual enzymatic steps. Glycolysis, the Krebs cycle, and oxidative phosphorylation each have their own stoichiometry. When I was running lab work measuring oxygen consumption in yeast cultures, I kept getting inconsistent ATP yield estimates because I wasn't accounting for the proton leak across the mitochondrial membrane. The theoretical maximum is about 30 to 32 ATP per glucose molecule under ideal conditions, but in real cells it's closer to 28 to 30 ATP because some protons slip back through without driving ATP synthase. That gap between the textbook number and reality is where most students get tripped up. Another thing that doesn't get emphasized enough: the equation assumes glucose as the sole substrate. In practice, cells oxidize fatty acids, amino acids, and other sugars through entry points scattered across glycolysis and the Krebs cycle. A palmitate molecule (C16), for example, goes through beta-oxidation and produces roughly 106 ATP. The overall "respiration equation" becomes something completely different when your fuel source isn't glucose. I once spent a week troubleshooting why my respirometer readings didn't match the predicted CO2 output based on the standard equation. The issue turned out to be that the bacterial culture was using an mixed-substrate medium containing both glucose and acetate. Acetate enters metabolism via the glyoxylate shunt, bypassing two decarboxylation steps in the Krebs cycle. That means less CO2 is released per carbon atom oxidized compared to pure glucose respiration. Once I isolated the glucose-only condition, the numbers aligned with the equation again. Mixed-substrate respiration is probably more common in environmental samples than people realize, and it throws off any calculation that assumes a single substrate.
The equation is fundamentally a bookkeeping tool. It tells you the inputs and outputs but nothing about the mechanism, the rate, or the efficiency under any given condition. For that you need kinetics data, enzyme concentrations, membrane potential measurements, and an understanding of how substrate availability limits each stage. The balanced equation is the starting point, not the destination.
Get the Full Details