So You're Asking About Ribosomes
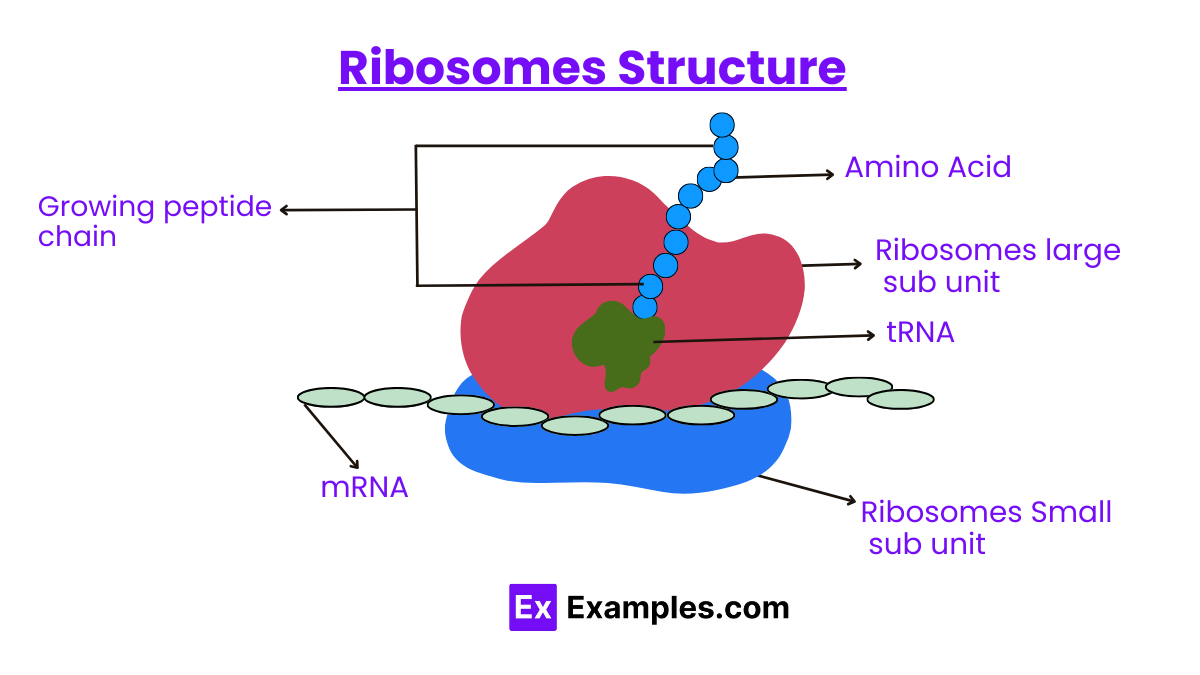
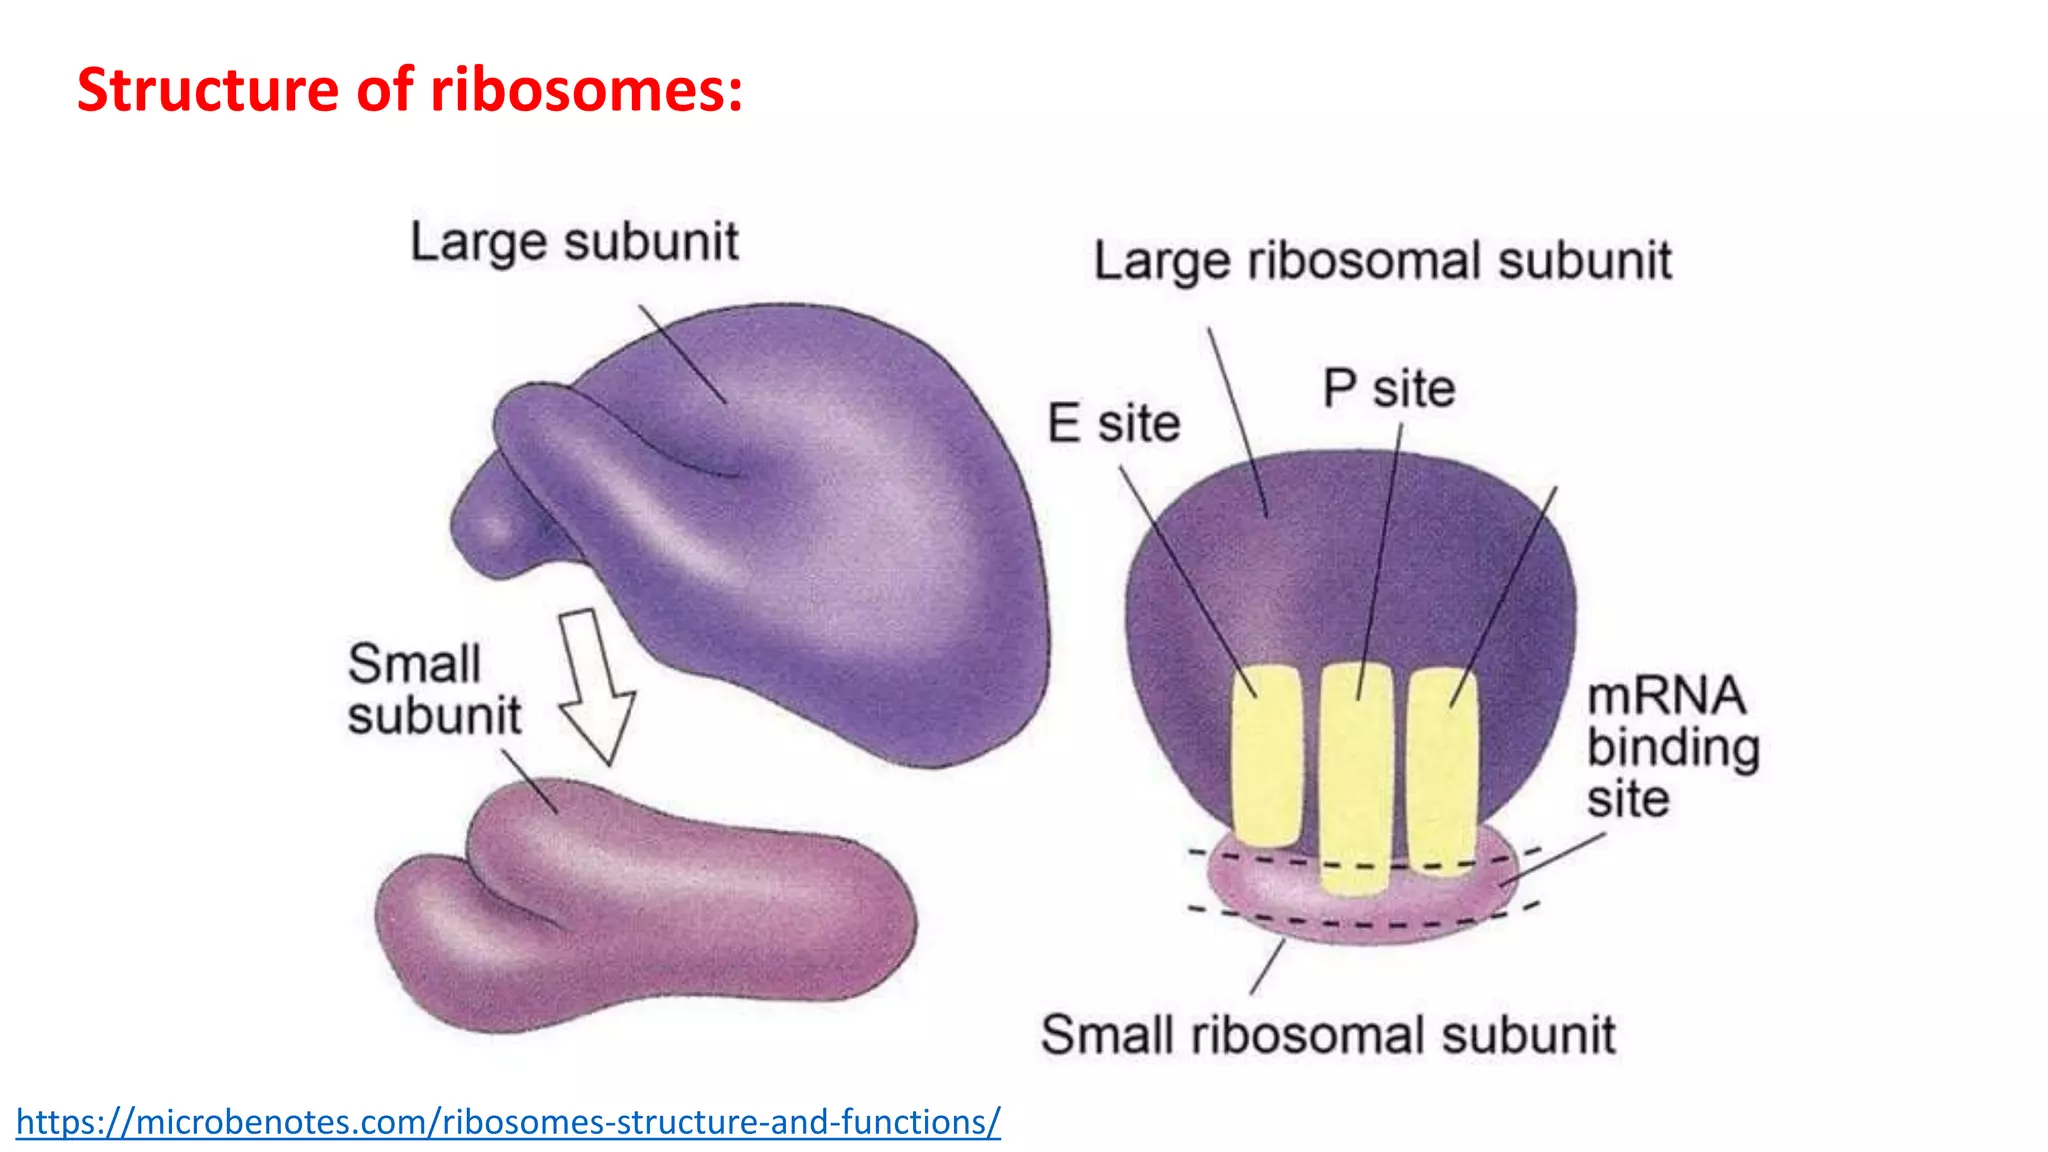
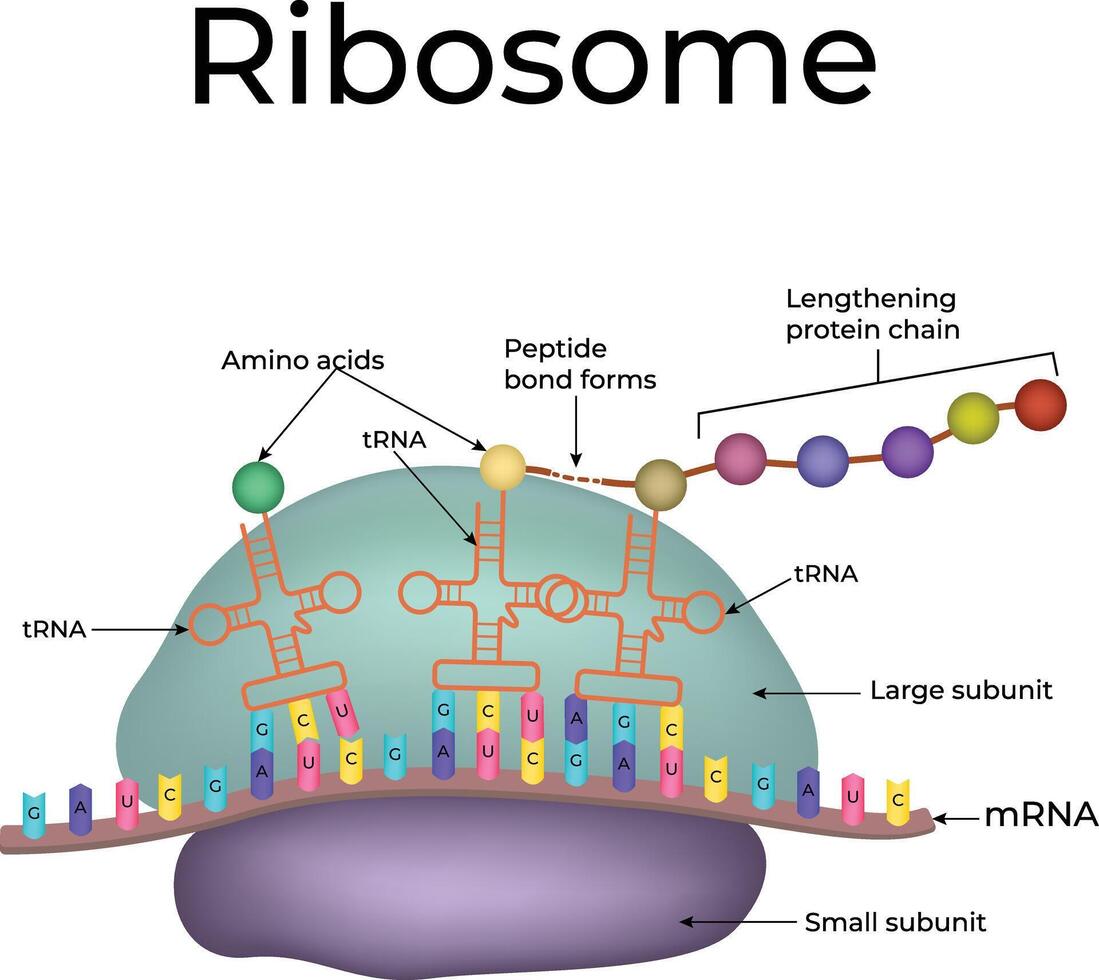
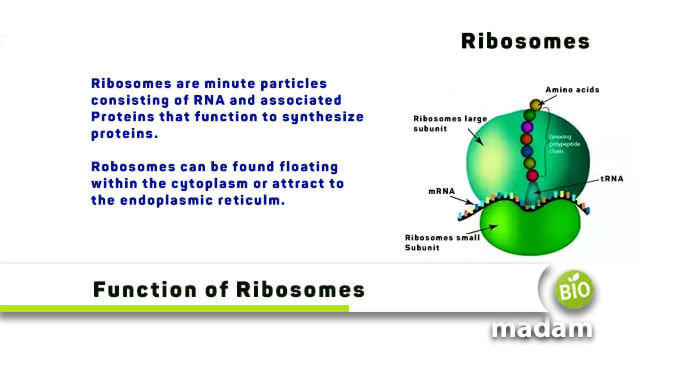
Most people think of ribosomes as tiny protein-making factories, which is technically true but misses half the story. If you're coming from a textbook background, you already know they read mRNA and string amino acids together. What nobody tells you is that ribosomes are way more finicky than that description implies, and if you're working with them in a lab setting, you'll find out the hard way how much they hate being disturbed. The ribosome is a ribonucleoprotein complex that catalyzes peptide bond formation during translation. It's made of two subunits — the small one handles mRNA binding and codon recognition, the large one handles peptidyl transferase activity and nascent chain exit. In bacteria, that's the 30S and 50S making a 70S particle. Eukaryotes have 40S and 60S subunits forming an 80S ribosome. Mitochondria go back to something closer to the bacterial setup, which is why some antibiotics affect them differently. The actual mechanics are straightforward until you try to observe them doing it. A ribosome sits on an mRNA molecule. The tRNA molecules bring amino acids matching each codon. The peptidyl transferase center — which is actually part of the rRNA, not any protein — forms the peptide bond. The ribosome translocates one codon forward, and the whole thing repeats until a stop codon arrives and release factors kick in. That's the basic cycle. It happens at roughly 15 to 20 amino acids per second in bacteria and maybe 6 to 10 in eukaryotes under normal conditions.
I spent way too many hours trying to purify actively translating polysomes back when I was running in vitro translation assays. The problem is that ribosomes are sensitive to salt concentration, Mg2+ levels, and even the order in which you add reagents. If your Mg2+ drops below about 5 millimolar during purification, the subunits dissociate and you're left with inactive fragments. I learned that after ruining three batches of reticulocyte lysate because I used the wrong buffer recipe from a paper that didn't specify the exact Mg2+ concentration they'd optimized for. The workaround was simple once I figured it out: keep MgCl2 at 2 millimolar during the gentle lysis step, then jump it to 10 millimolar for the centrifugation through the sucrose cushion. Everything else fell into place after that. Here's something textbooks gloss over: ribosomes don't just make proteins, they also determine how fast those proteins are made and whether they fold correctly. The speed of translation varies across different regions of an mRNA. Slow codons — the ones with rare tRNAs — cause the ribosome to pause, and those pauses can be critical for proper protein folding. If you overexpress a gene with lots of rare codons in E. coli, you'll often get inclusion bodies instead of soluble protein because the ribosome stalls and the nascent chain misfolds. The fix isn't always just switching to a special strain with extra rare tRNAs, though that helps. Sometimes you need to lower the induction temperature to 16 or 18 degrees Celsius and let the ribosome breathe. I've seen people crank through that problem in a single afternoon by doing exactly that instead of running yet another round of expression condition screening. Another thing that trips people up is the distinction between free and bound ribosomes. Free ribosomes in the cytoplasm make proteins that stay in the cytoplasm or go to the nucleus, peroxisomes, or mitochondria. Bound ribosomes attached to the rough ER make secreted proteins, membrane proteins, and proteins headed for lysosomes. The signal recognition particle grabs the emerging signal sequence on the nascent chain and docks the whole ribosome-mRNA complex to the ER membrane through the translocon. Once that's happening, the polypeptide goes straight into the ER lumen as it's being synthesized. This coupling of translation and translocation is why you can't just stick a secretory protein gene into the cytoplasm and expect it to end up outside the cell. The ribosome has to be physically at the membrane for it to work.
There are also specialized ribosome variations now being studied — things like ribosome heterogeneity, where different cell types or conditions produce ribosomes with slightly different rRNA modifications or ribosomal protein compositions. The idea is called the specialty ribosome hypothesis, and it's still controversial. Some groups have shown that specific ribosomal protein knockouts can selectively affect translation of certain mRNAs over others, which would mean the ribosome isn't just a generic machine. But other groups can't reproduce those findings, and the field is divided. I tend to think there's probably some truth to it but it's being overstated in popular science coverage. The ribosome is still mostly a universal translator, just with some tuning knobs. Antibiotics target bacterial ribosomes specifically because of the structural differences between 70S and 80S particles. Macrolides like erythromycin bind the 50S subunit and block the peptide exit tunnel. Tetracyclines bind the 30S subunit and prevent tRNA entry. Aminoglycosides like streptomycin bind the 30S and cause misreading of the genetic code. Chloramphenicol blocks peptidyl transferase in the 50S. These all work because the bacterial ribosome is different enough from the human version that the drugs pick one over the other. Not perfectly — that's why aminoglycosides can cause ototoxicity and nephrotoxicity at high doses, because they occasionally interact with mitochondrial ribosomes, which are structurally similar to bacterial ones. That's a direct consequence of the endosymbiotic origin of mitochondria. If you're working with ribosomes in practice, here are the things that actually matter that you won't find in the methods section of most papers. First, RNase contamination is your biggest enemy. Ribosomes areRNA-heavy, and RNases are everywhere — on your hands, in the dust, on the surface of everything. Use RNase-free tips, tubes, and water. Wear gloves. Change them frequently. Second, freeze-thaw cycles destroy ribosomal activity. Aliquot everything and never thaw the main stock. Third, if you're doing ribosome profiling or deep sequencing of translated mRNAs, the RNase digestion step has to be carefully titrated. Too much and you digest the mRNA between ribosomes down to nothing. Too little and you get overlapping footprints that make the data unusable. I usually optimize this by running a gel after digestion and looking for a clear ladder pattern — monosome, dimer, trimer — with the inter-ribosomal mRNA completely digested.
Get the Full Details
The function of the ribosome is often taught as a simple concept, but the reality is messier and more interesting. They're not just protein synthesizers — they're regulatory hubs that influence when and how proteins are made, how they fold, and where they end up. They're drug targets, evolutionary puzzles, and still not fully understood. The basics are solid, but if you dig into the details, especially at the experimental level, you'll find plenty of edges and exceptions that the simplified models leave out.