Understanding Inbreeding in Breeding Programs
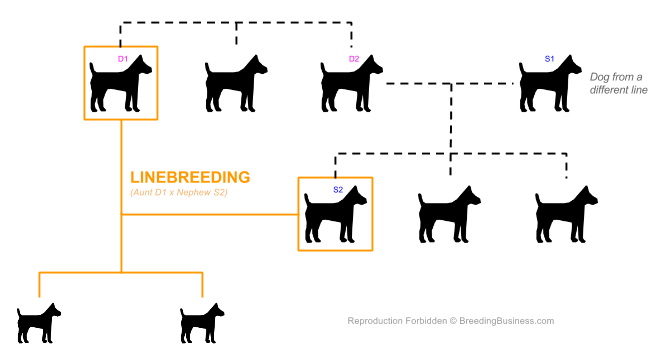
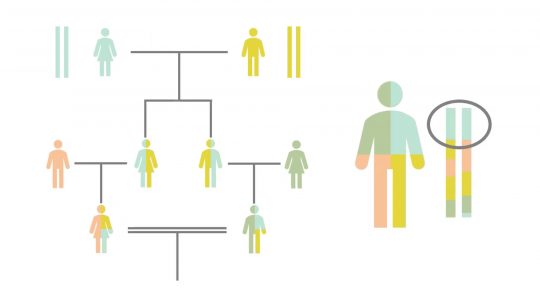
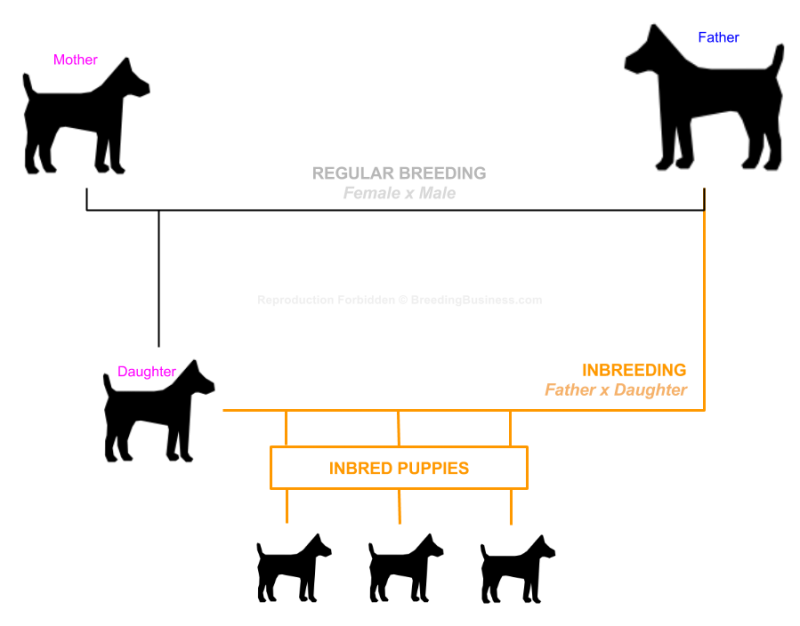
Most people hear the word inbreeding and immediately think of bad outcomes. That is only half true. Inbreeding is simply mating between closely related individuals. That is it. It is a neutral mechanism. How it plays out depends entirely on what you are breeding for and how carefully you manage the results. At its core, inbreeding increases homozygosity. When two relatives mate, their offspring inherit identical copies of genes from a shared ancestor. Over a few generations, the proportion of the genome that is homozyg rises sharply. The exact rate depends on the relationship between the parents. Full siblings or parent-offspring pairings produce roughly a 25 percent inbreeding coefficient in the first generation. First cousins land closer to 6.25 percent. These numbers come from standard Wright coefficients and they track reliably across mammals, birds, plants, and fish. I spent several years running a small poultry breeding program. I started with four foundation lines that had very narrow genetic diversity because the breed was nearly extinct. My first move was intentional inbreeding. I created a closed loop of full-sibling matings across three generations. The goal was not cruelty. It was fixation. I needed certain traits to become predictable so I could then cross those fixed lines into a commercial project. The process took about eighteen months. Without that step, the traits I was selecting for would have shifted every generation.
How Inbreeding Actually Works in Practice
The mechanics are straightforward. Each generation of close mating doubles the chance that both alleles at a locus come from the same ancestor. For a diploid organism, the formula is simple enough to calculate by hand. You do not need specialized software for basic pedigree work. A spreadsheet with parent tags and a recursion function will track the inbreeding coefficient F for any individual in a closed population. What people miss is that inbreeding does not cause problems by itself. It exposes them. Recessive alleles that sit hidden in heterozygous carriers become visible when homozygosity rises. If your population carries lethal or sublethal recessives, those show up quickly. If the population has been purged of those alleles over many generations, the same amount of inbreeding causes much less damage. That is why some lines tolerate close mating while others collapse under identical coefficients. In my poultry work, the third generation of full-sibling mating showed a clear drop in hatchability. Eggs that should have hatched failed early in development. I ran a quick culling protocol: I removed any hen that produced more than two non-viable eggs in a clutch and replaced her from a slightly less related backup line. Hatchability recovered within two generations. The cost was losing about fifteen percent of my original stock, but the resulting line had the trait stability I needed for the crossbreeding phase.
The Purging Effect and Why It Matters
Purging is the process by which deleterious recessive alleles are removed from a population through selection during inbreeding. When homozygosity exposes a harmful allele, individuals carrying it die or fail to reproduce. Those alleles drop out of the gene pool faster than they would in an outbred population where they remain hidden. Purging takes time. It usually requires multiple generations and a fairly large effective population size to avoid the population crashing before purge completes. A counter-intuitive point: moderate inbreeding in a large, diverse population can sometimes improve long-term fitness compared to staying outbred with hidden load. This is not a universal rule. It depends on the specific allele frequencies in your stock and how strong your selection pressure is. If you are working with a small population, purging often fails because drift overwhelms selection. The population just goes extinct before purge finishes.
Get the Full Details
Measuring and Managing Inbreeding
You have several tools available. The pedigree-based inbreeding coefficient F is the traditional metric. It calculates expected homozygosity from known relationships. It works well when your pedigree is accurate and deep. If you skip a few generations, the numbers drift. Modern programs use genomic inbreeding estimates from SNP data. Runs of homozygosity give you a direct measure of actual identity-by-descent segments. ROH length distributions also tell you when inbreeding happened recently versus anciently. Long ROH mean recent close mating. Short ROH mean older shared ancestry. I switched to ROH-based tracking after my initial pedigree work showed inconsistency. The pedigree said my best breeder had an F of 0.12. The genomic data showed F of 0.21 based on ROH sum. The pedigree missed a hidden half-sib relationship in the maternal line going back four generations. That gap cost me one season of misplaced confidence before I caught it. I started requiring SNP data for any animal entering a closed breeding nucleus. The upfront cost is about thirty dollars per sample with standard genotyping arrays, but it pays for itself quickly when you avoid a bad cross.
Common Pitfalls
The biggest mistake I see is treating inbreeding as a problem to avoid at all costs. That leads to populations with high hidden load and unpredictable performance. The second mistake is pushing inbreeding too far without monitoring fitness. I watched a hobbyist breeder run five generations of full-sibling mating in a small rabbit colony. No culling. No tracking. The colony crashed at generation four. Total loss. Inbreeding depression is not a cliff. It is a slope. You can walk it carefully if you measure each step. A third pitfall is assuming that outcrossing always fixes inbreeding problems. Outcrossing introduces new variation, which is good, but it also re-heterozygotes everything you worked to fix. If you spent three generations fixing a desired trait through inbreeding and then outcross broadly, you lose that fixation immediately. The solution is structured crossing. Fix what you need, then cross to a divergent line with complementary traits, then select in the F2 or backcross generation to recover the fixed trait in a new genetic background.
When Inbreeding Should Not Be Used
Certain situations make inbreeding a poor choice. Small endangered populations with fewer than fifty effective individuals should not be pushed into close mating. The risk of drift fixation outweighs any benefit. Conservation breeding programs typically maintain minimum mean kinship instead of pursuing fixation. Commercial livestock operations that prioritize hybrid vigor over trait uniformity also avoid inbreeding in the production population. Inbreeding is reserved for creating the parental lines that will later be crossed for heterosis. If you are working with a species that has high reproductive variance and low effective population size, like many captive reptiles and amphibians, even mild inbreeding can cause problems. I once advised a colleague who was breeding a rare gecko species. He tried a simple full-sibling pair. The clutch was viable, but the offspring showed severe spinal deformities in forty percent of the hatchlings. We stopped immediately and switched to a carefully managed outcross program using the only other available males from a different captive colony. The deformation rate dropped to near zero in the next generation.

Practical Steps if You Are Starting
Begin with a clear goal. Are you fixing a trait, purging load, or building a line for eventual crossing? Your answer determines how close you go and how fast. Calculate your starting pedigree coefficients before you make any matings. Set hard limits on F. For most small-scale projects, keeping the inbreeding coefficient below 0.25 during the fixation phase and then outcrossing is a safe boundary. Monitor fitness traits every generation. Hatchability, survival, fertility, growth rate, whatever is relevant to your species. If you see a decline of more than ten percent in any metric between consecutive generations, pause and reassess. Keep detailed records. Every mating, every outcome, every phenotype. The difference between a controlled inbreeding program and a disaster is usually documentation. I keep spreadsheets going back eight generations for each line. It takes time. It is boring. It also prevented me from accidentally mating two animals with a hidden relationship that would have pushed F above 0.35. That kind of error is easy to miss without a paper trail.
The Bottom Line
Inbreeding is a tool. It creates homozygosity. That homozygosity reveals both the traits you want to fix and the recessive problems you need to eliminate. It is not inherently good or bad. It is a question of how deliberately you use it and how rigorously you monitor the results. The programs that fail treat it as a magic solution or a moral failing. The programs that succeed treat it as a calculated step in a longer breeding strategy.