So You Need To Know What Is The Law Of Independent Assortment
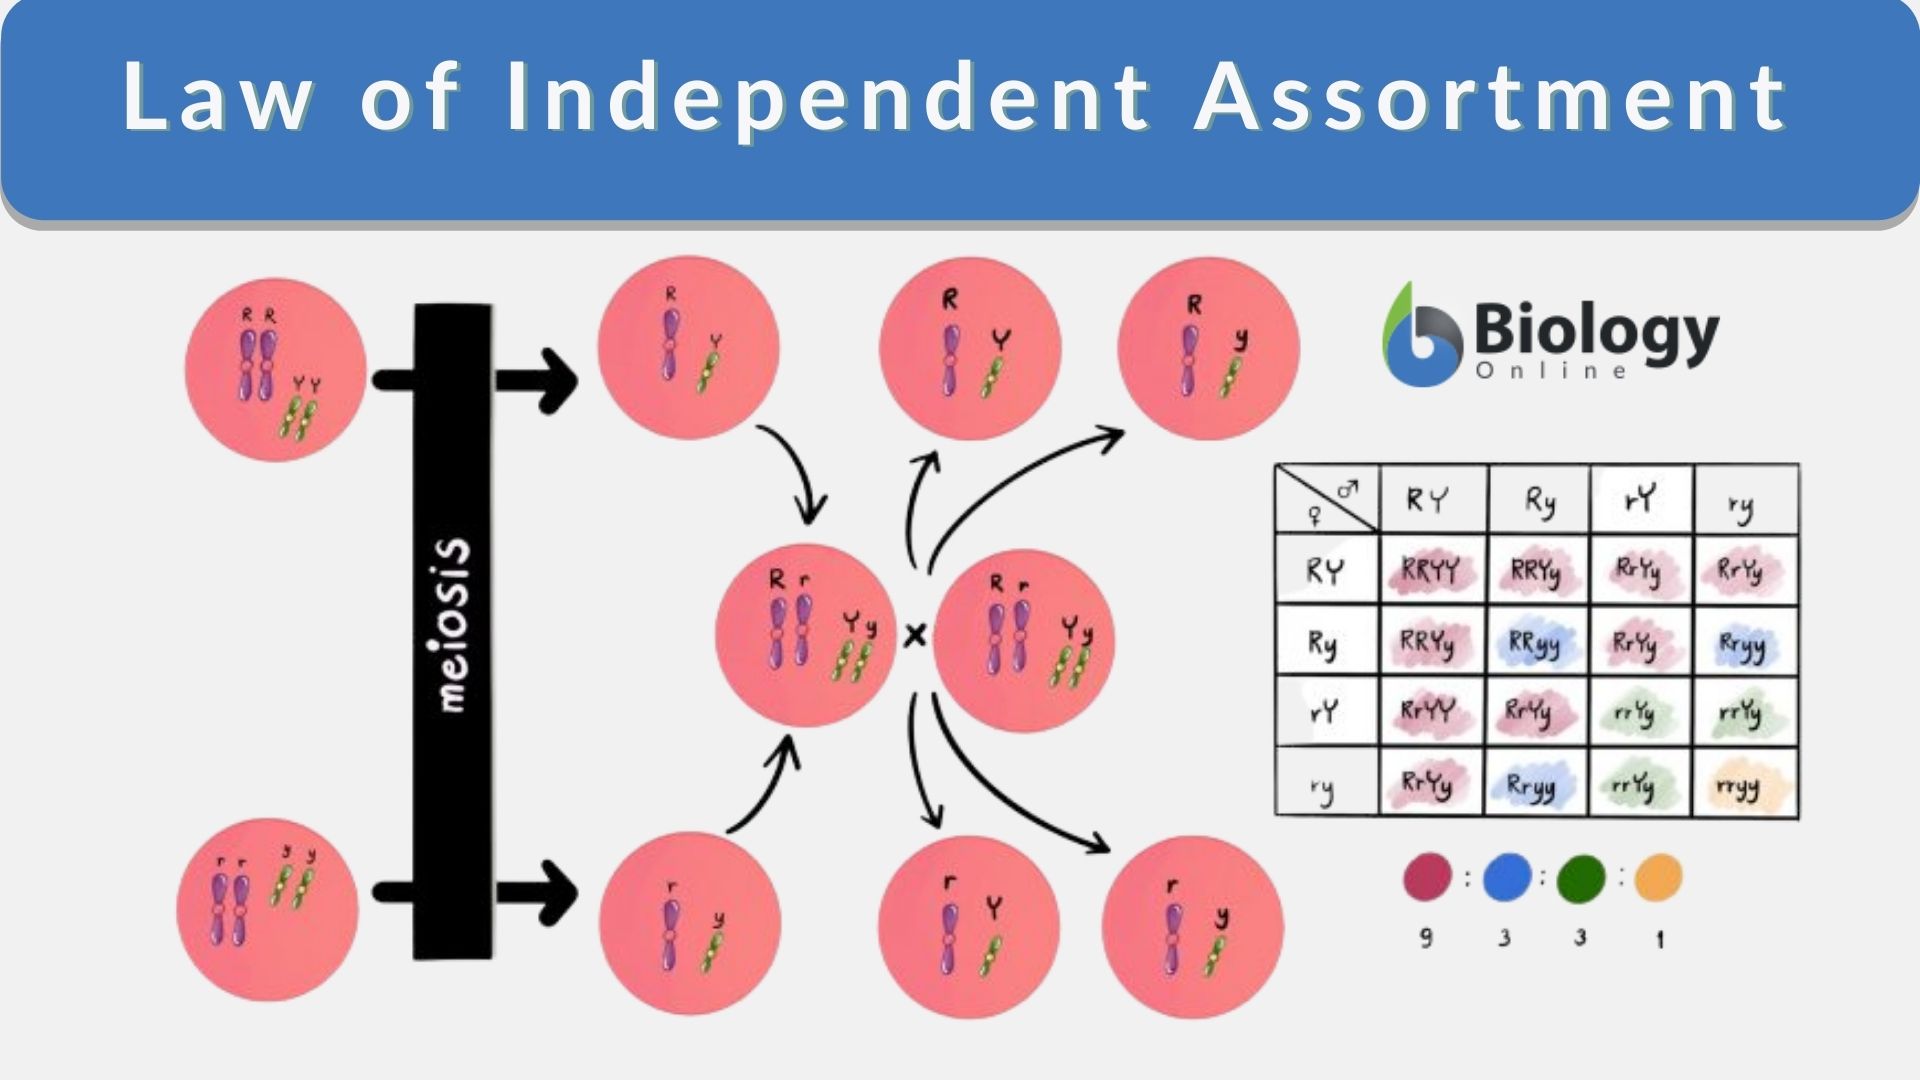
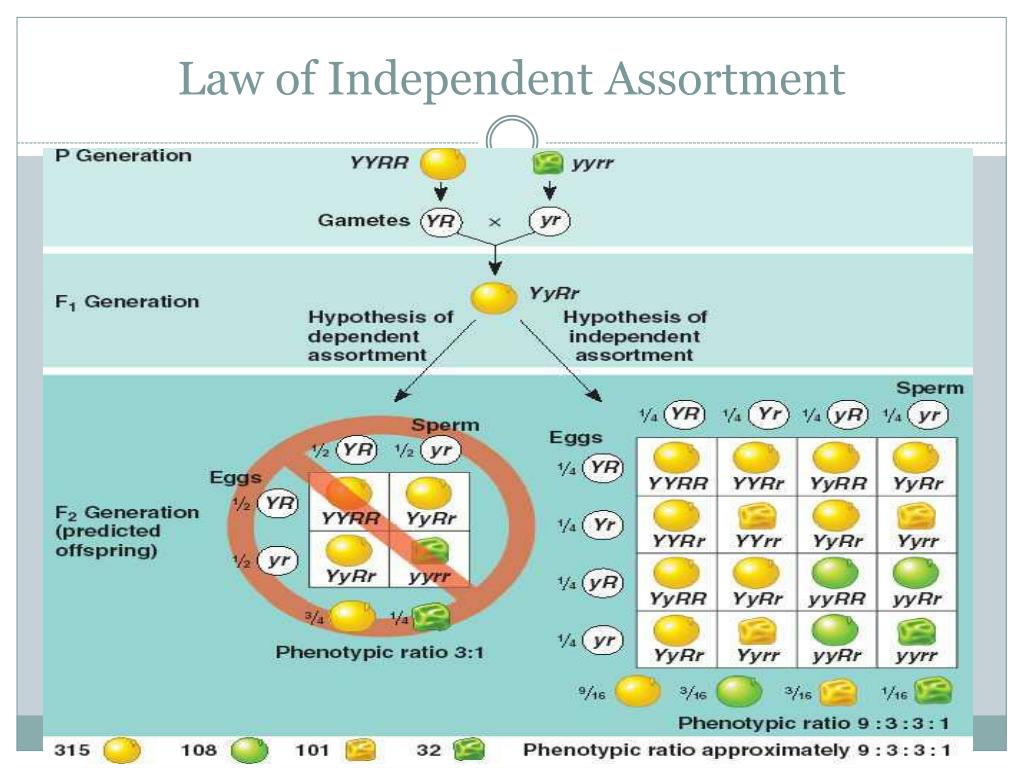
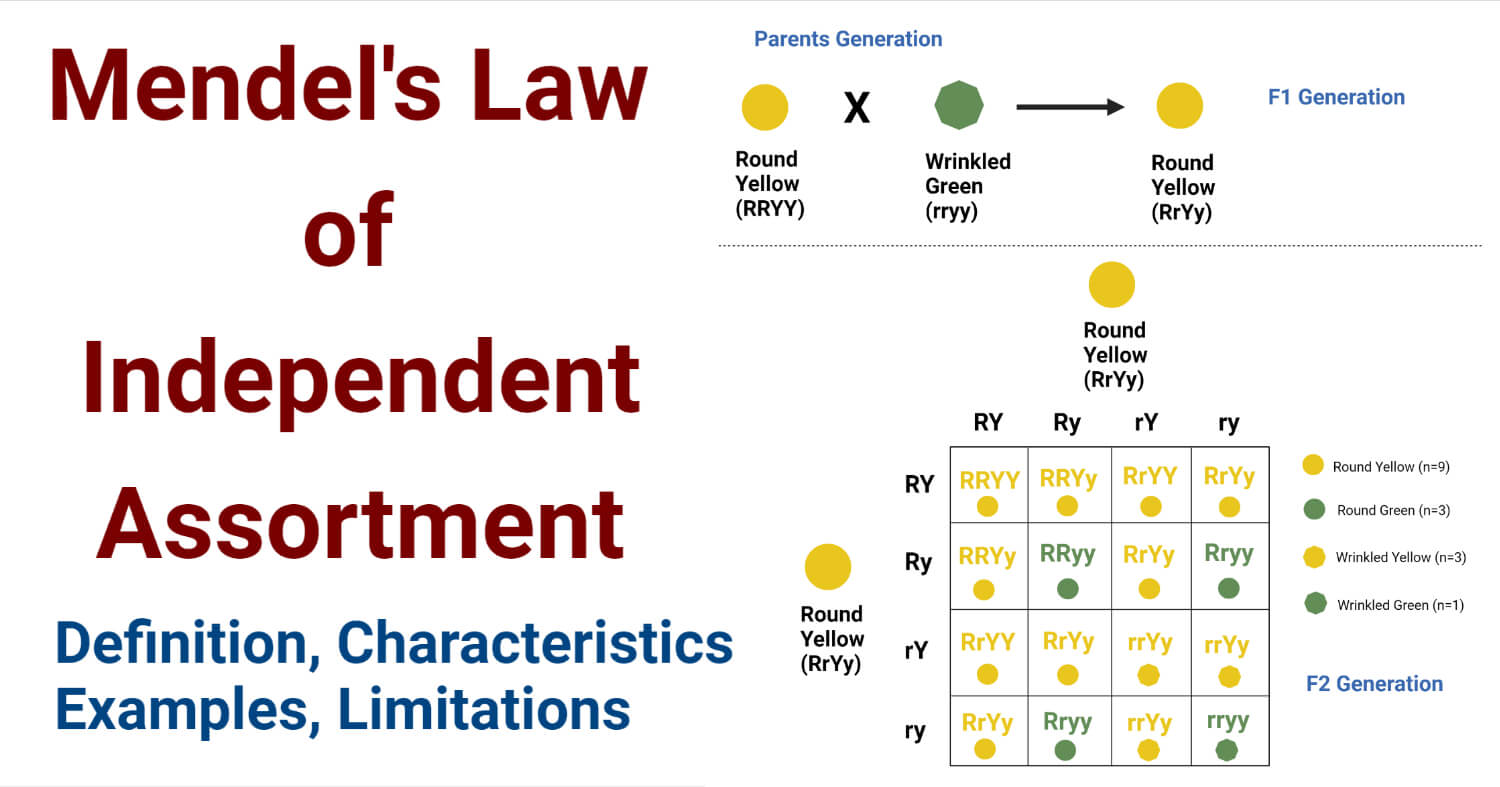
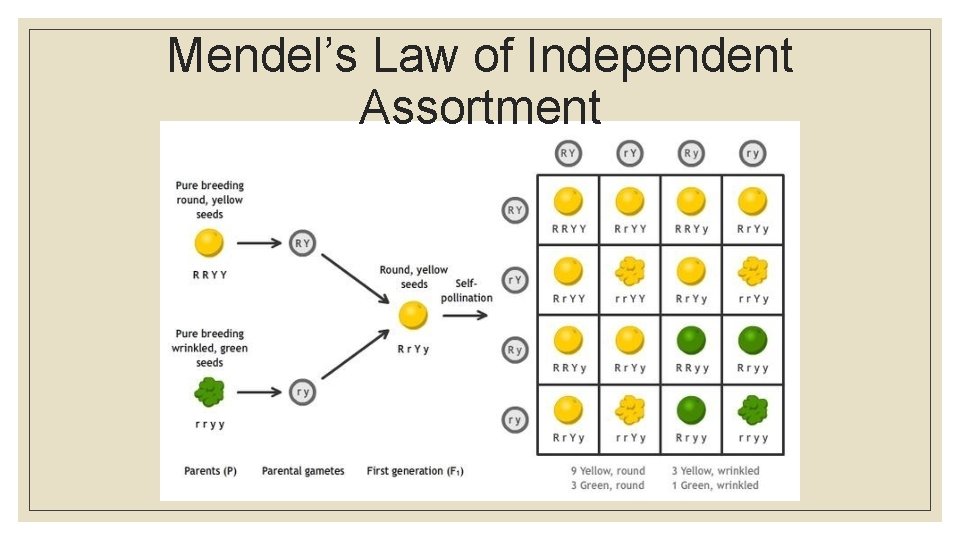
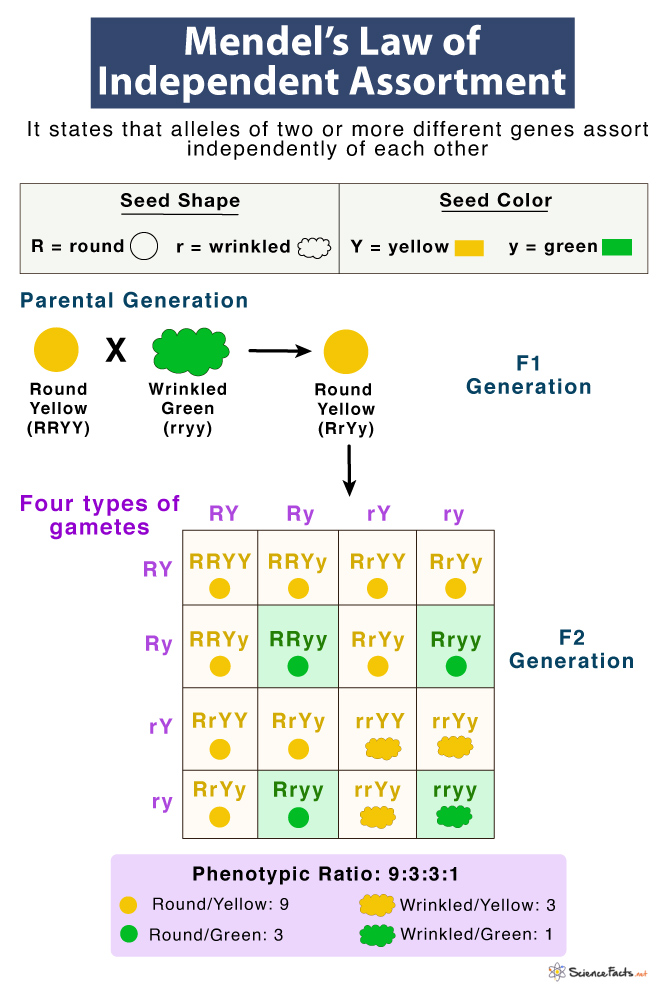
I've seen too many students trip over this in undergrad genetics. It's Mendel's second law and it's straightforward until you actually have to use it. Here's how it works in practice. During gamete formation, the alleles at one locus separate independently of the alleles at another locus. That means the inheritance of trait A doesn't influence the inheritance of trait B. Mendel figured this out by crossing peas that differed in two characteristics at once — seed color and seed shape. Yellow and round crossed with green and wrinkled. The F2 generation gave him that classic 9:3:3:1 phenotypic ratio, and from that he inferred the independent assortment of the two gene pairs. The mechanism behind it is meiosis. Specifically, metaphase I. Homologous chromosome pairs line up at the metaphase plate, and each pair orients randomly relative to the others. One pair might have the maternal chromosome facing one pole while the other pair has the paternal chromosome facing that same pole. This random alignment is what generates the independent assortment. After anaphase I, the resulting gametes carry every possible combination of the parental alleles.
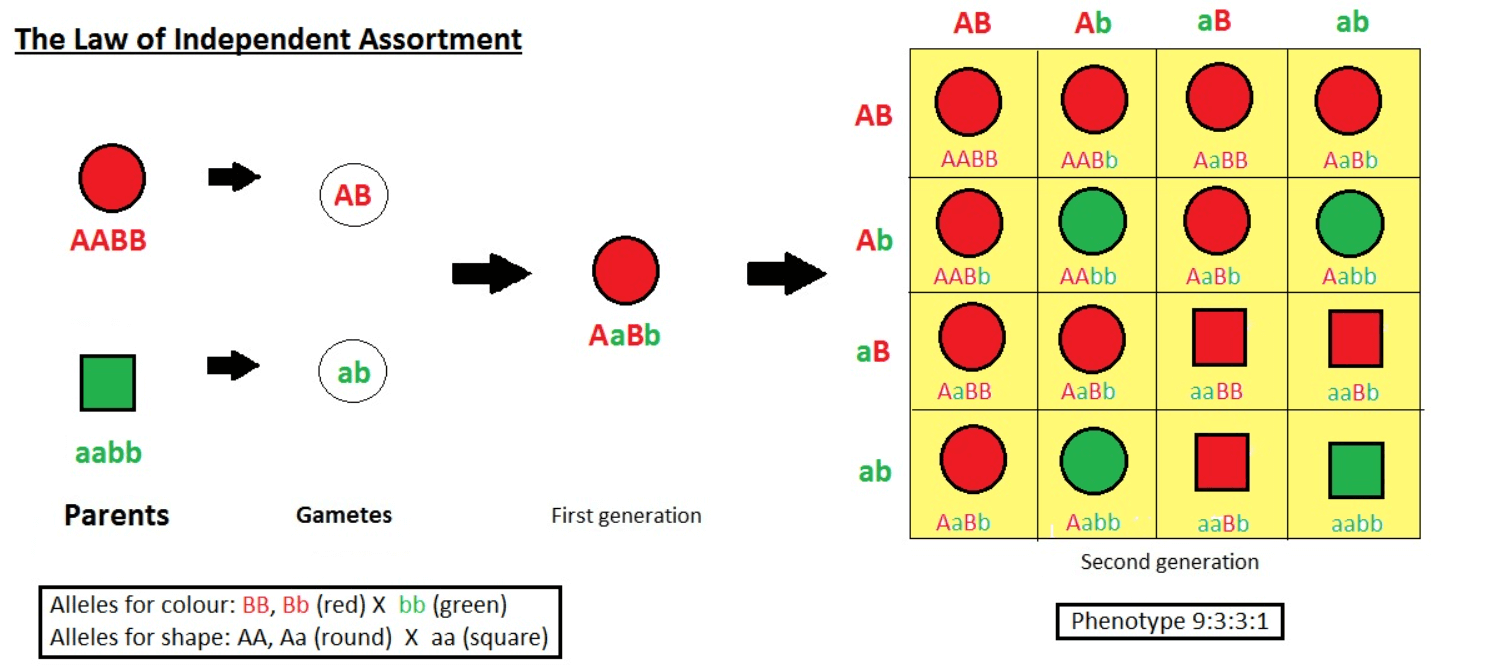
For a dihybrid cross where both parents are heterozygous at two unlinked loci, you get four types of gametes from each parent. Combine them and you're looking at 16 possible genotypes. The math works out neatly when the genes are on different chromosomes or far enough apart on the same chromosome that they behave as if they're unlinked.
Where People Get It Wrong
The biggest mistake is assuming this law applies universally. It doesn't. Genes that are close together on the same chromosome don't assort independently. They're linked. I spent an afternoon in graduate school wrestling with a mapping cross where the observed ratios were nowhere near what independent assortment predicted. The recombination frequency was about 8 percent instead of the 50 percent you'd expect from unlinked genes. Once I realized linkage was the issue, I switched to using a test cross with a homozygous recessive individual and calculated map distances from the recombinant classes instead of forcing the data through a Punnett square that assumed independence. Another pitfall is treating the 9:3:3:1 ratio as a universal constant. It only holds when both parents are heterozygous at both loci, when there's complete dominance at each locus, when the genes are truly unlinked, and when all genotypes have equal viability. Miss any one of those conditions and the numbers shift.
Get the Full Details
Practical Use Cases
If you're doing a genetics problem set and need to figure out gamete types from a given genotype, independent assortment makes it simple. An individual with the genotype AaBb produces four gamete types in equal frequency: AB, Ab, aB, and ab. For a trihybrid like AaBbCc, you get eight gamete types. The general rule is that the number of possible gamete combinations equals 2 to the power of n, where n is the number of heterozygous loci. So three heterozygous loci gives you 2 cubed, which is 8. Four gives you 16. This only works when the genes assort independently. When you're actually planning a breeding experiment, the law matters because it tells you whether you can predict offspring ratios directly or whether you need to account for linkage first. If two genes are linked, you need to determine the recombination frequency before you can make any meaningful predictions. A quick test cross will tell you whether they're linked or not. If the recombinant classes appear at roughly 50 percent, the genes are unlinked and independent assortment applies. If they're significantly less than 50 percent, you're dealing with linkage.
The Limits of This Approach
Independent assortment only describes half the picture. It says nothing about what happens within a single chromosome pair — that's the law of segregation, Mendel's first law. Both laws together give you the foundation, but they don't cover everything. Epistasis, incomplete dominance, codominance, sex linkage, mitochondrial inheritance, and gene conversion all fall outside the scope of independent assortment. If you're working with organisms that have small genomes and tight linkage like Drosophila or Arabidopsis, you'll run into linked genes pretty quickly. The law still describes the principle correctly for unlinked loci, but your actual data won't match the expected ratios unless you factor in recombination. For teaching purposes or basic problem solving, assuming independent assortment is usually fine as a first approximation. But in real research, especially with whole genome data, ignoring linkage when it exists will give you wrong answers every time. The workaround is straightforward: map your loci first, or at minimum check the recombination frequency before applying independent assortment calculations to your crosses.