How Mendel Actually Figured This Out
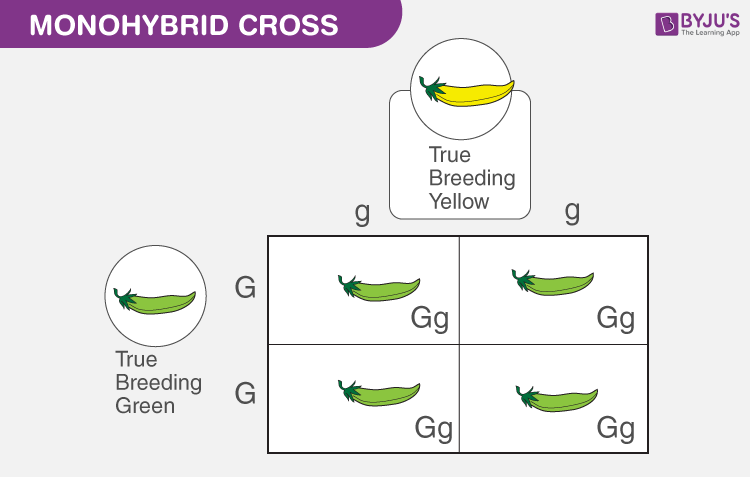
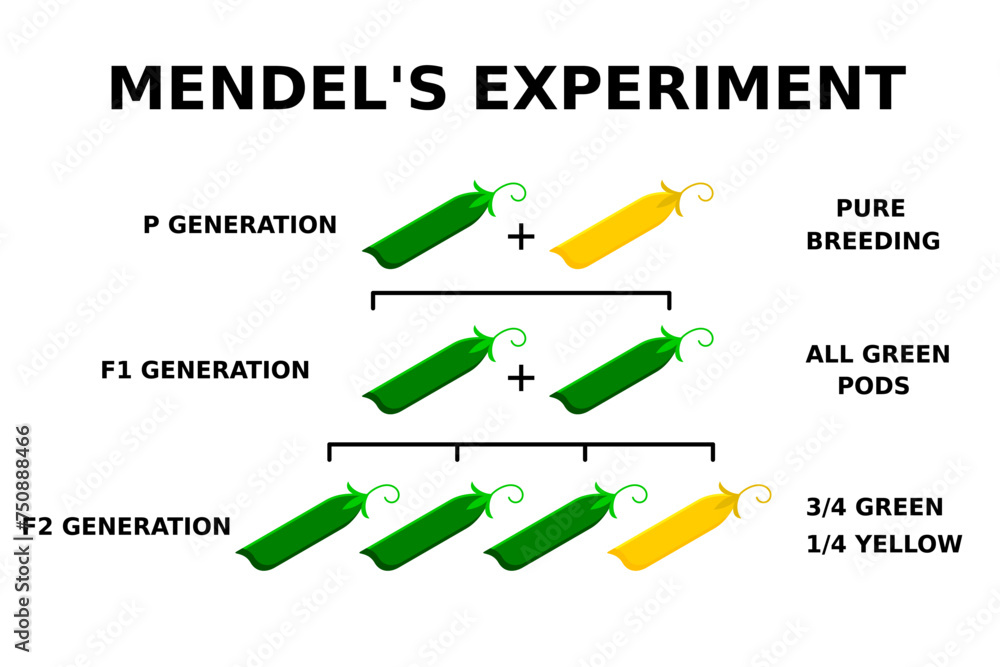
Mendel grew pea plants. He counted thousands of them. That's where the law comes from - not some philosophical insight, just someone doing tedious agricultural counting work and realizing patterns emerged when you track one trait at a time. The formal definition people memorize for exams says that allele pairs separate during gamete formation and randomly unite at fertilization. The practical version is simpler: every organism carries two copies of each gene, and when it makes sperm or eggs, those copies split apart. Each gamete gets exactly one. The offspring then inherits one from each parent, restoring the pair.
What Is The Law Of Segregation In Practice
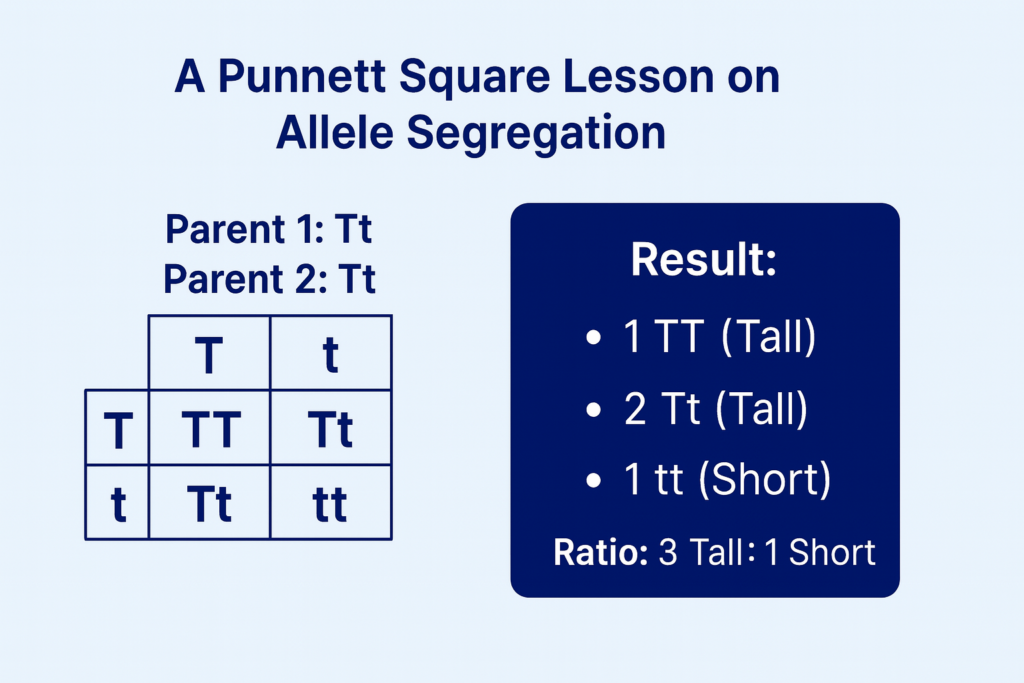
Here's how it actually manifests. Take a heterozygous plant with genotype Aa. When it produces gametes, half carry A and half carry a. Not sometimes, not probabilistically in a way that shifts - exactly half, assuming normal meiosis. Cross two Aa individuals and you get the familiar 3:1 phenotypic ratio in the F2 generation if A is dominant. The ratio breaks down because the law only applies cleanly when you're tracking a single gene with two alleles showing complete dominance. I spent weeks troubleshooting unexpected ratios in Drosophila crosses back in grad school before realizing I'd accidentally set up a cross where the gene was linked to a sex chromosome. The segregation was happening fine, but the phenotypic ratios got skewed because males and females inherited the alleles differently. The law wasn't violated, my reading of the data was just wrong. This is the part most textbooks don't emphasize enough. The law describes what happens to alleles, not what you observe in offspring. You can have perfect segregation and still see distorted ratios due to linkage, epistasis, or selection against certain genotypes. When I see students get confused by ratios that don't match 3:1, I tell them to check whether segregation actually occurred first before blaming the law.
When The Law Doesn't Apply
Mendel's first law works for diploid organisms undergoing sexual reproduction with discrete genes on separate chromosomes. It fails in several common scenarios that appear in lab work and real breeding programs. Meiotic drive is one I encountered practically. In some mouse strains carrying the t-haplotype, the allele manipulates meiosis so that over 90 percent of sperm carry it instead of the expected 50 percent. The alleles still segregate during cell division, but the resulting gamete frequencies are wildly unbalanced. The law of segregation held at the chromosomal level, but the phenotypic expectations based on it were completely wrong. Polyploidy creates another issue. If an organism has three or more copies of a chromosome, like many cultivated wheat varieties, you can't describe inheritance with simple two-allele segregation. Tetraploids produce gametes with two copies of each chromosome, and the math gets complicated fast. I've seen breeding programs try to apply diploid ratios to polyploid crops and waste months on misinterpreted results.
Get the Full Details
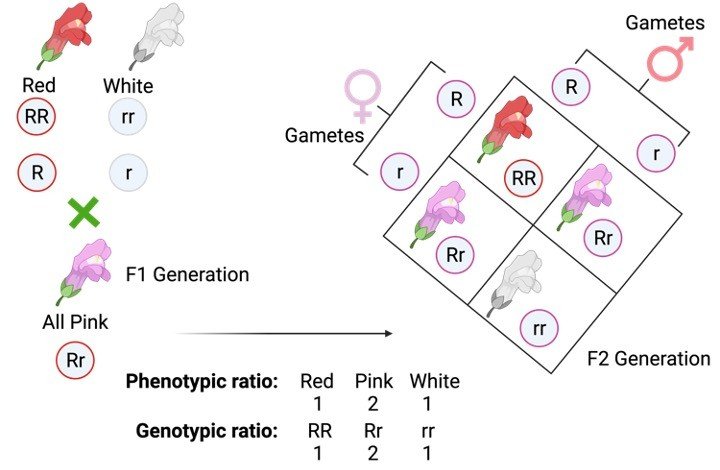
Gene conversion during meiosis is rarer but real. The Holliday junction model shows that homologous recombination doesn't always produce clean 50:50 splits at the DNA level. Sometimes one allele copies over the other during repair, creating transient distortion. This matters more in fungi and plants with large asci where you can actually observe the four products of a single meiosis.
Why Students Get Confused
The confusion usually comes from mixing up three different things: segregation of alleles, assortment of chromosomes, and independent inheritance of traits. The law of segregation deals with alleles at one locus. The law of independent assortment deals with alleles at different loci on different chromosomes. People conflate them constantly. Another source of trouble is thinking segregation happens during fertilization. It doesn't. It happens during meiosis, specifically anaphase I when homologous chromosomes separate. Fertilization is just the random meeting of already-segregated gametes. When I grade exams and see students write that segregation creates genetic diversity, I mark it wrong. Segregation maintains the status quo of allele distribution. Recombination and random union of gametes create the diversity. The practical implication for anyone working with pedigrees or breeding data is to verify that you're dealing with simple Mendelian inheritance before applying these laws. Real populations have incomplete dominance, codominance, lethal alleles, and penetrance issues that make clean ratios disappear. I once spent three weeks trying to fit a segregation model to a family's neuromuscular disorder data before accepting that reduced penetrance was masking the true inheritance pattern. The law wasn't wrong, the model was just too simple for the biology.
Testing Whether Segregation Actually Occurred
In practice, you test this with a chi-square goodness-of-fit test. Count your offspring phenotypes, calculate expected numbers from the predicted ratio, and see whether the deviation is statistically significant. A typical cutoff is p
0.05, meaning if you'd see this kind of deviation by chance less than 5 percent of the time under the null hypothesis, you reject the model. Sample size matters a lot. With only ten offspring, random drift can easily produce ratios that look wrong. I usually tell people to aim for at least twenty to thirty individuals per cross before trusting the statistics. A 3:1 ratio in twelve offspring could be 8:4 or 9:3, and both fall within normal sampling variation. The law doesn't care about your small sample size. Tie-breakers come up when you're working with plants or microorganisms where you can do testcrosses. Crossing an unknown genotype to a homozygous recessive individual reveals the unknown's alleles directly because the recessive parent contributes only recessive alleles. If the unknown is heterozygous, half the offspring show the dominant phenotype and half show recessive. If homozygous dominant, all show dominant. This is the standard verification method in genetics labs and still works reliably after a century.

The main limitation is that testcrosses require the organism to be sexually reproducible and the recessive phenotype to be distinguishable. Many human genetic conditions lack clear homozygous recessive controls, which is why we rely on segregation analysis and linkage mapping rather than direct crosses. The principle is the same, the methodology just gets indirect.