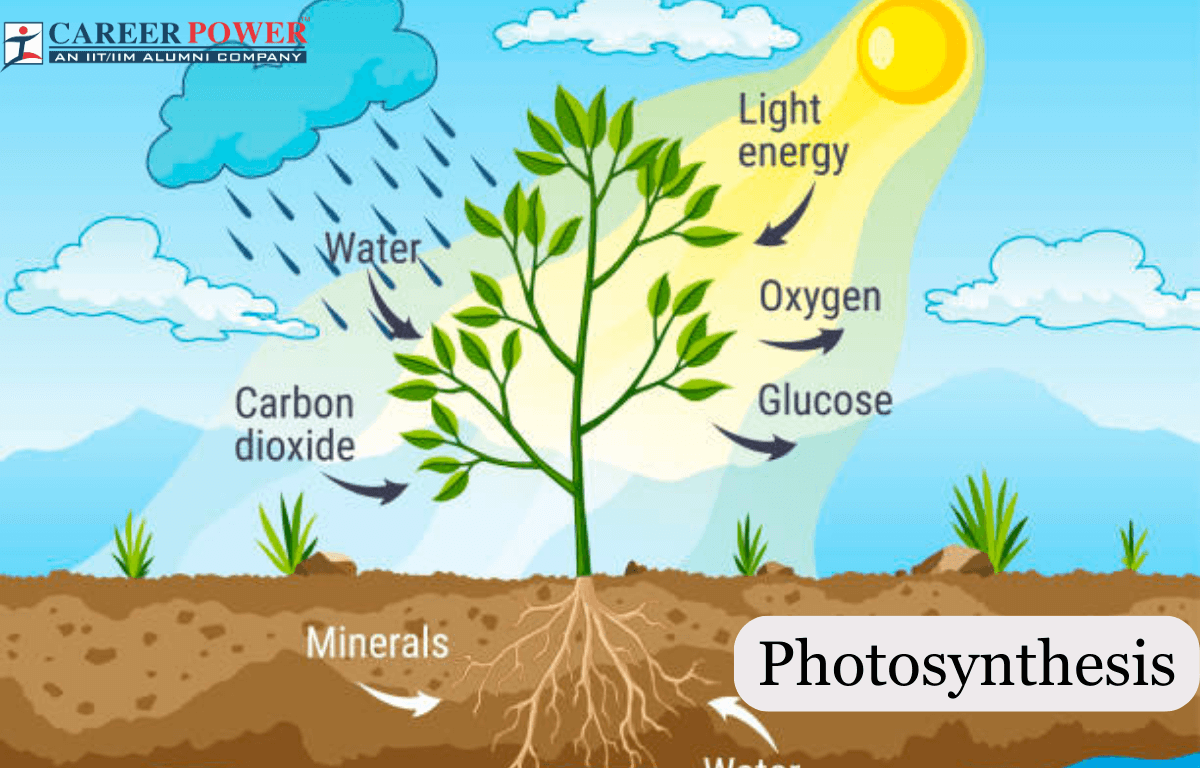
Let's Talk About How Plants Actually Work
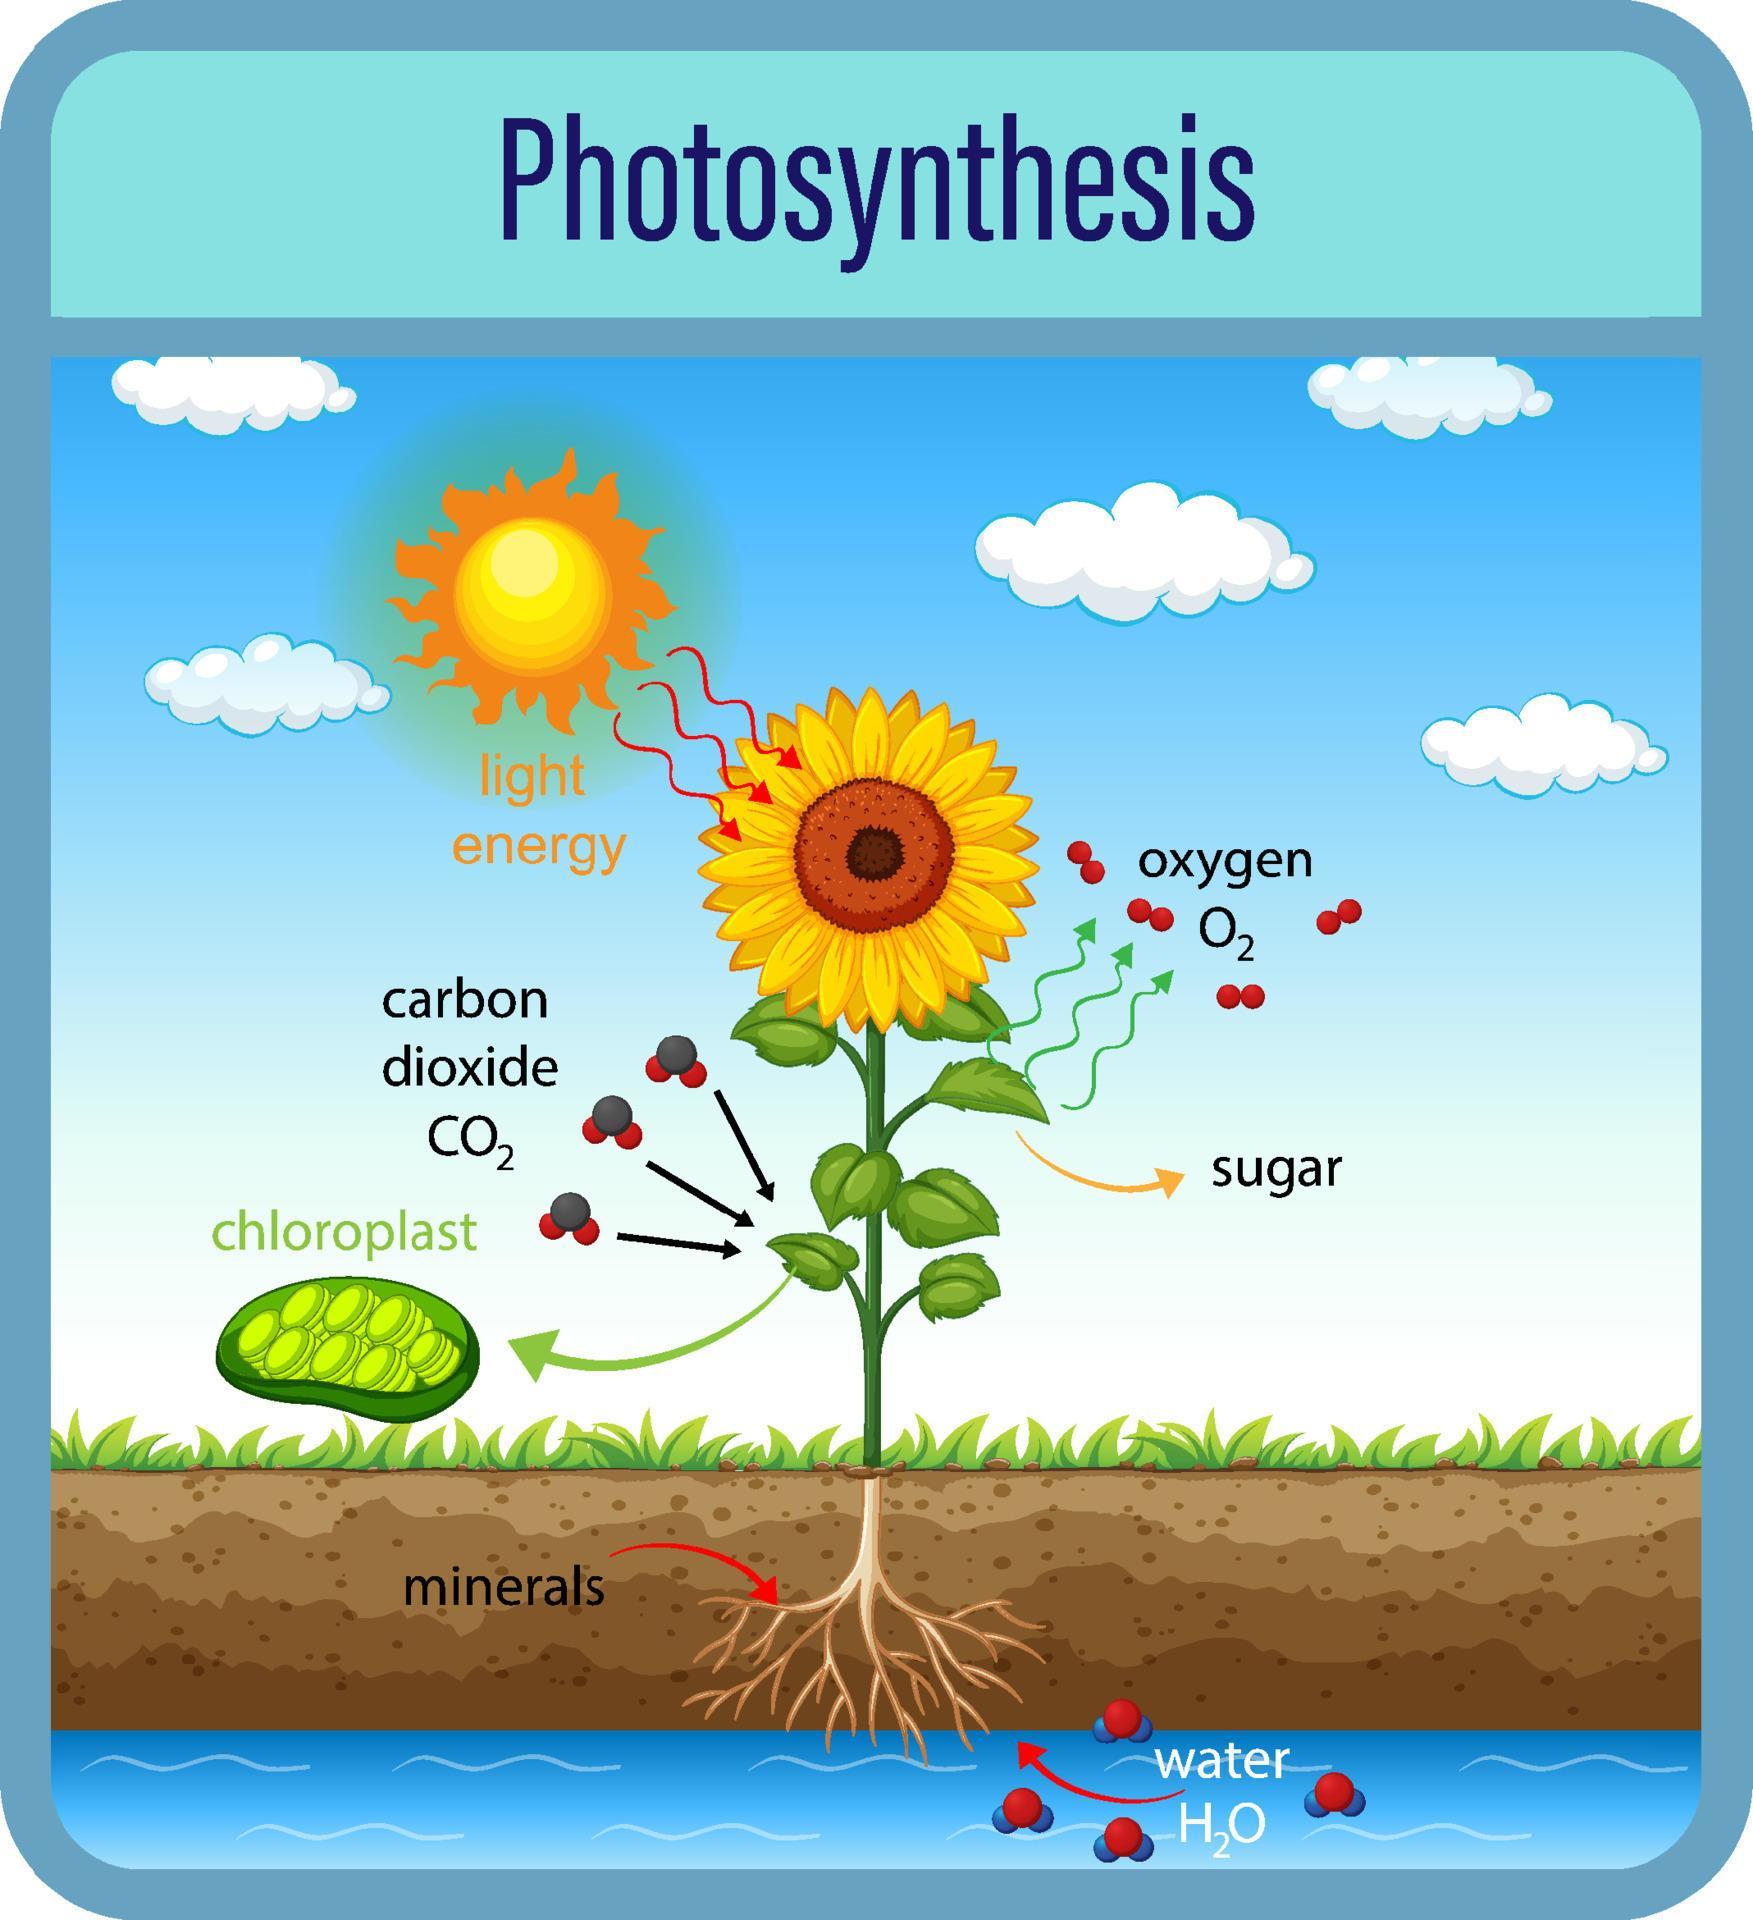
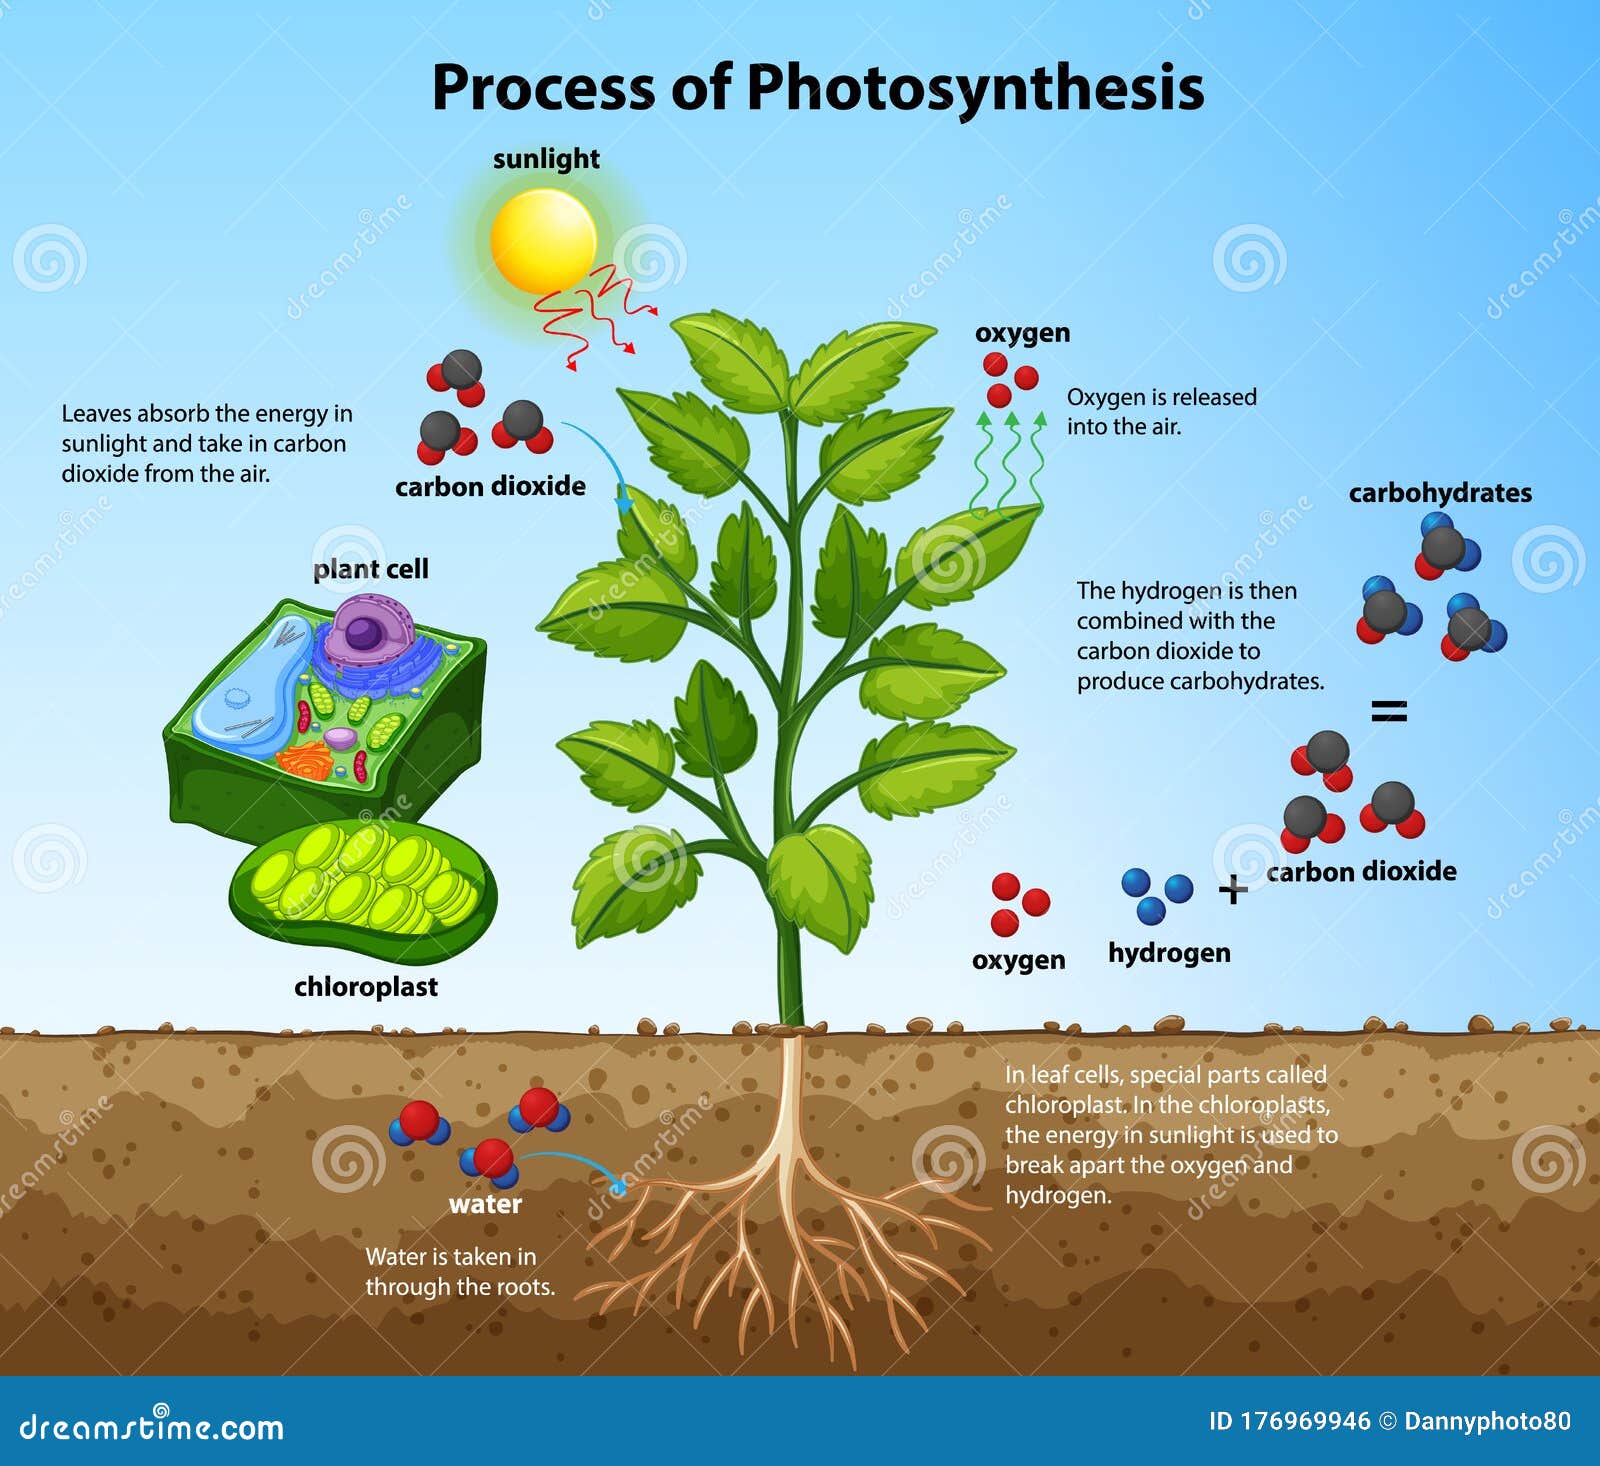
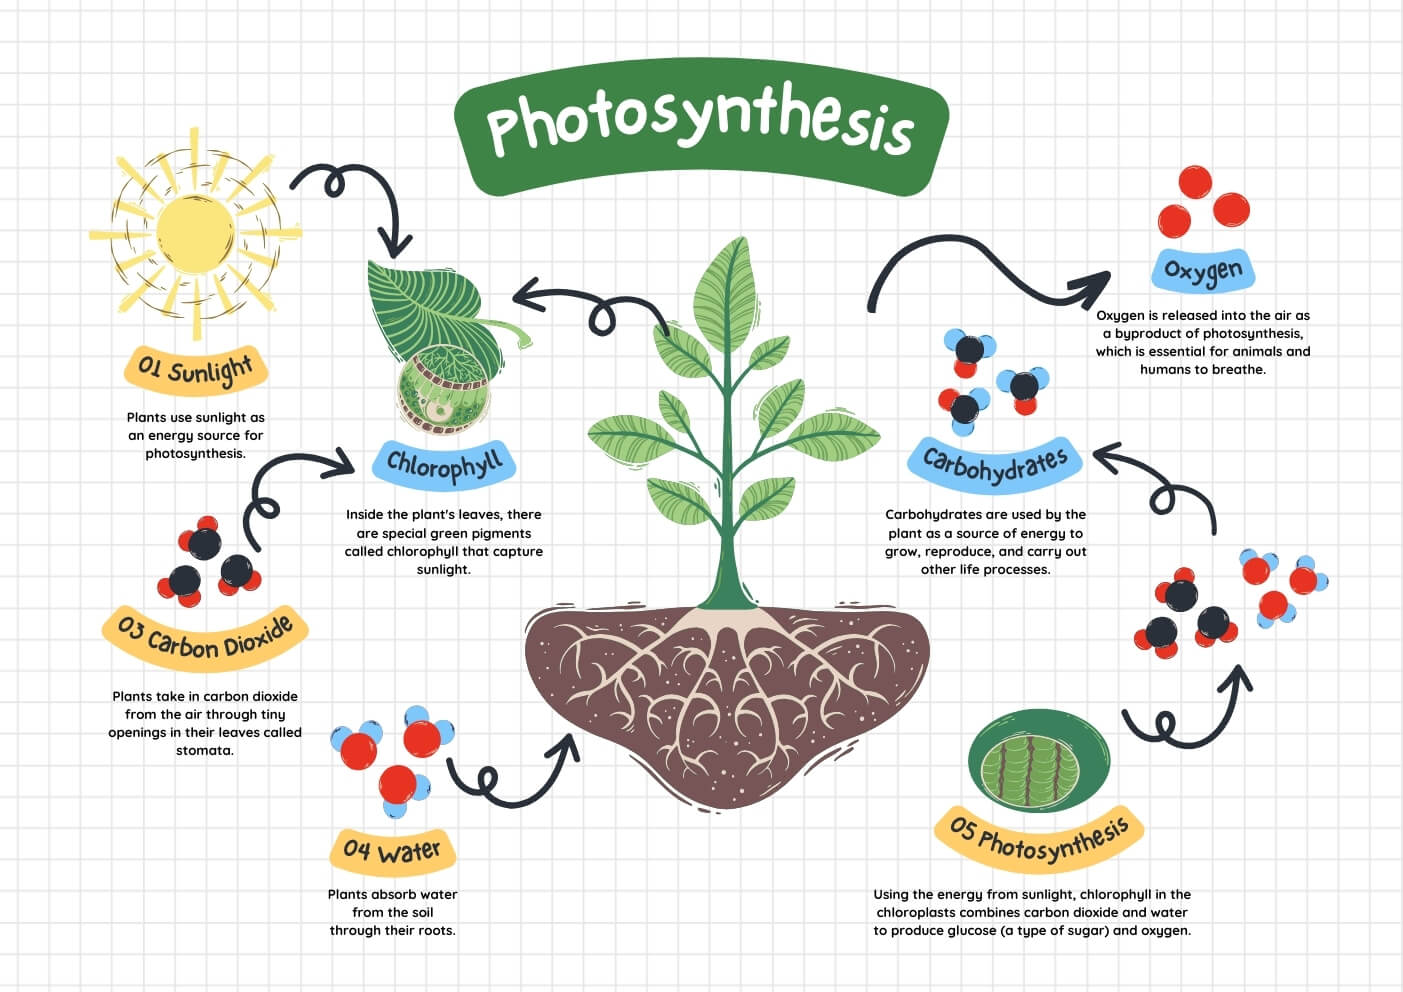
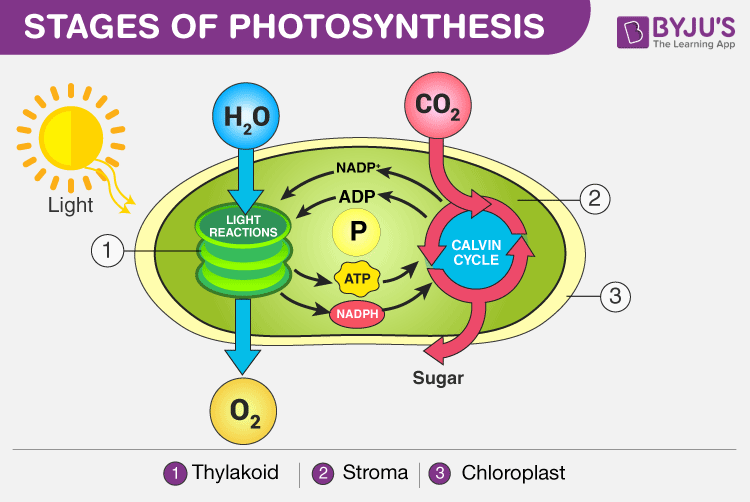
Photosynthesis is the process by which plants, algae, and some bacteria convert light energy into chemical energy stored in glucose. The overall equation is straightforward: carbon dioxide and water, using light energy, produce glucose and oxygen. But the actual mechanism is layered and involves two distinct stages—the light-dependent reactions and the Calvin cycle—that most people gloss over because they're trying to memorize a single balanced equation for a biology test. The purpose, stripped of textbook poetry, is energy conversion and biomass production. Plants capture photons and use that energy to build carbohydrate molecules from inorganic precursors. That's it. Everything else—oxygen as a byproduct, the elaborate pigment systems, the thylakoid membranes—is just engineering built around that core function. The oxygen we breathe is a waste product from splitting water molecules. Plants don't care about us breathing; they care about making sugar. I've spent years working with plant physiology data, and one thing always surprises newcomers: the Calvin cycle doesn't actually need darkness. Despite being called the "light-independent reactions," it runs continuously during the day whenever ATP and NADPH are available from the light reactions. The naming convention is misleading and causes a lot of confusion in undergraduate courses. Plants don't pause their carbon fixation at night just because the name suggests they might. Some plants, like CAM species (cacti, pineapples), do separate the processes temporally, but that's a specialized adaptation, not the rule.
The light-dependent reactions happen in the thylakoid membranes of chloroplasts. Photosystems II and I absorb photons through pigment clusters—chlorophyll a, chlorophyll b, and carotenoids. Electrons get excited, travel through the electron transport chain, and the resulting proton gradient drives ATP synthase. Water is split to replace the lost electrons, releasing oxygen as a byproduct. NADP+ picks up electrons at the end of the chain to become NADPH. This process generates roughly 3 ATP and 2 NADPH per molecule of CO2 fixed in the standard C3 pathway. Here's something most sources don't emphasize enough: C3 photosynthesis, the most common pathway, has a significant flaw. The enzyme RuBisCO, which catalyzes the first major step of carbon fixation, can also bind oxygen instead of carbon dioxide. When it does, you get photorespiration—a wasteful process that consumes energy and releases previously fixed CO2 without producing any sugar. In hot, dry conditions, plants close their stomata to conserve water, which causes CO2 levels inside the leaf to drop and O2 levels to rise. RuBisCO grabs oxygen more often, and photosynthetic efficiency can drop by 30 to 50 percent. This is why C4 and CAM plants evolved—they've built workarounds for this fundamental enzymatic weakness. I ran into a real problem once while calibrating gas exchange measurements on tomato plants under controlled environment conditions. The initial readings showed wildly inconsistent net photosynthesis rates across replicates grown under identical light and temperature. We spent two weeks troubleshooting before realizing the issue was stomatal limitation caused by a slight humidity gradient across the growth chamber. The plants on the drier side were partially closing their stomata, which restricted CO2 intake and made the photosynthetic rates look pathological when they were actually just a environmental artifact. The workaround was running a vapor pressure deficit calculation for each leaf compartment and normalizing the gas exchange data against actual stomatal conductance rather than assuming uniform opening. Once we did that, the variability dropped significantly and the true photosynthetic differences between treatments became clear. It's a detail that rarely comes up outside of actual lab work.
The efficiency of photosynthesis as an energy conversion process is surprisingly low. Only about 1 to 2 percent of incoming solar energy is typically converted into chemical energy in plant biomass. The rest is reflected, transmitted, or lost as heat. Even under optimal laboratory conditions, the theoretical maximum quantum efficiency of photosynthesis caps out around 4 to 6 percent for C3 plants. This isn't because plants are poorly designed—it's because of the thermodynamic constraints of capturing diffuse, low-energy photons and converting them into high-energy chemical bonds. One counter-intuitive point worth noting: more light doesn't always mean more photosynthesis. Beyond the light saturation point, which varies by species, additional photons don't increase the rate of carbon fixation. Instead, excess light energy can damage the photosynthetic apparatus, particularly Photosystem II. Plants have photoprotective mechanisms—non-photochemical quenching, the xanthophyll cycle—to dissipate excess energy as heat, but these mechanisms themselves consume resources and reduce overall efficiency. In agricultural settings, this is why dense crop canopies often have lower per-leaf productivity than sparsely planted crops. The upper leaves are light-saturated and wasting energy, while the lower leaves are light-limited and struggling to fix carbon. There are also practical limits to how much we can push photosynthetic efficiency through genetic modification. Researchers have been working on engineering RuBisCO variants with better specificity for CO2 over O2, and some progress has been made, but the results in field conditions have been underwhelming. The enzyme is deeply embedded in complex regulatory networks, and improving one property often degrades another. There's no simple fix for a problem that evolved over billions of years.
Get the Full Details
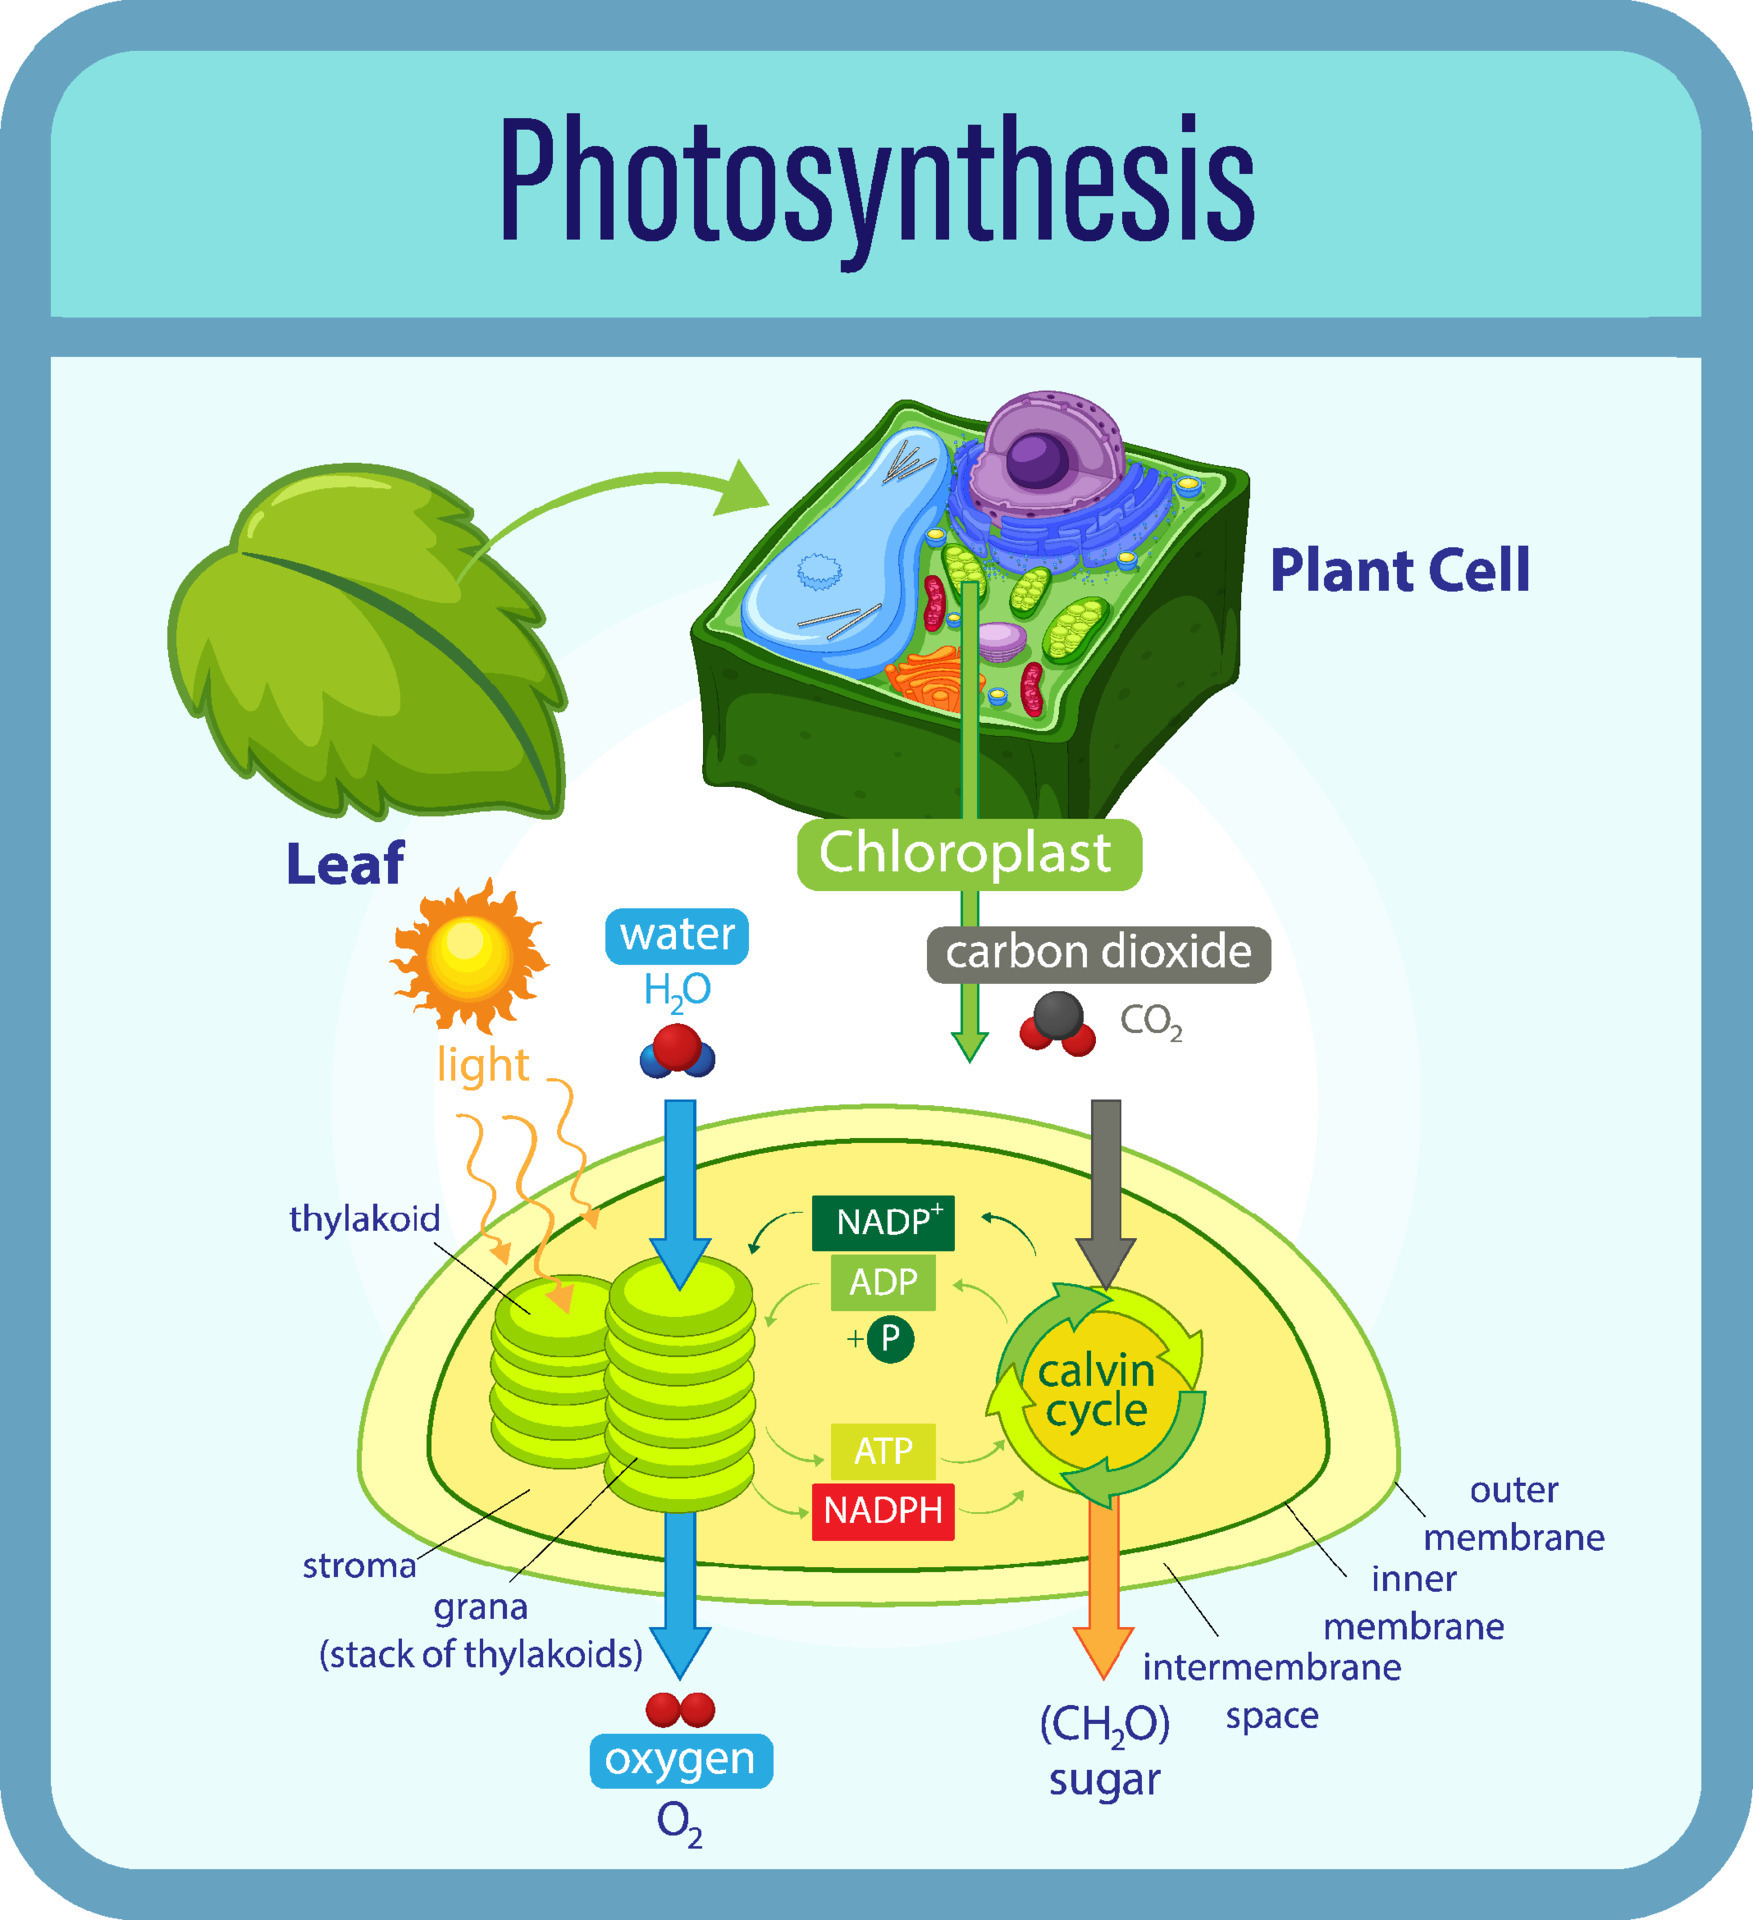
The broader ecological purpose of photosynthesis extends well beyond individual plants. It's the foundation of nearly all terrestrial and marine food webs. The glucose produced feeds everything from herbivores to decomposers. The oxygen it generates maintains the atmospheric composition that aerobic organisms depend on. Carbon fixation through photosynthesis removes roughly 120 gigatons of carbon from the atmosphere annually, playing a critical role in regulating global climate. When you're studying this for practical purposes—whether that's agriculture, ecology, or just understanding how the natural world works—focus less on memorizing the reaction equation and more on understanding the constraints. The limitations of RuBisCO, the trade-offs between water conservation and carbon intake, the efficiency losses at every step—these are what determine how plants grow and where they can survive. The chemistry is elegant but messy, and that messiness is what makes it interesting.