Understanding Wobble Base Pairing in Codon-Anticodon Recognition
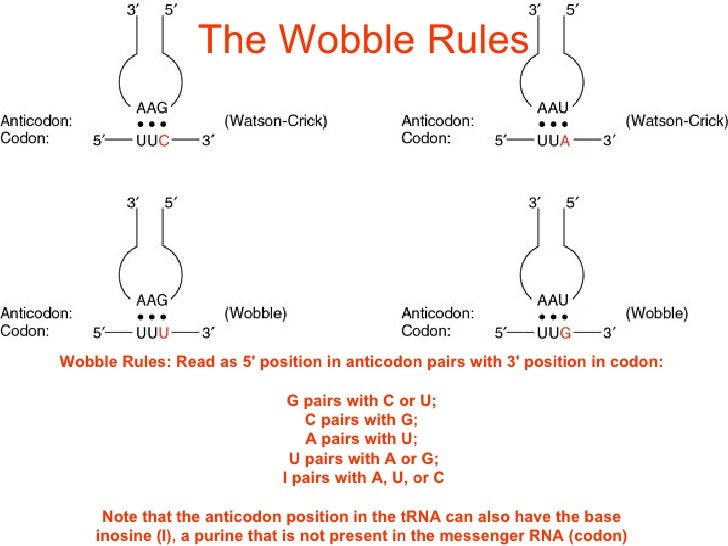
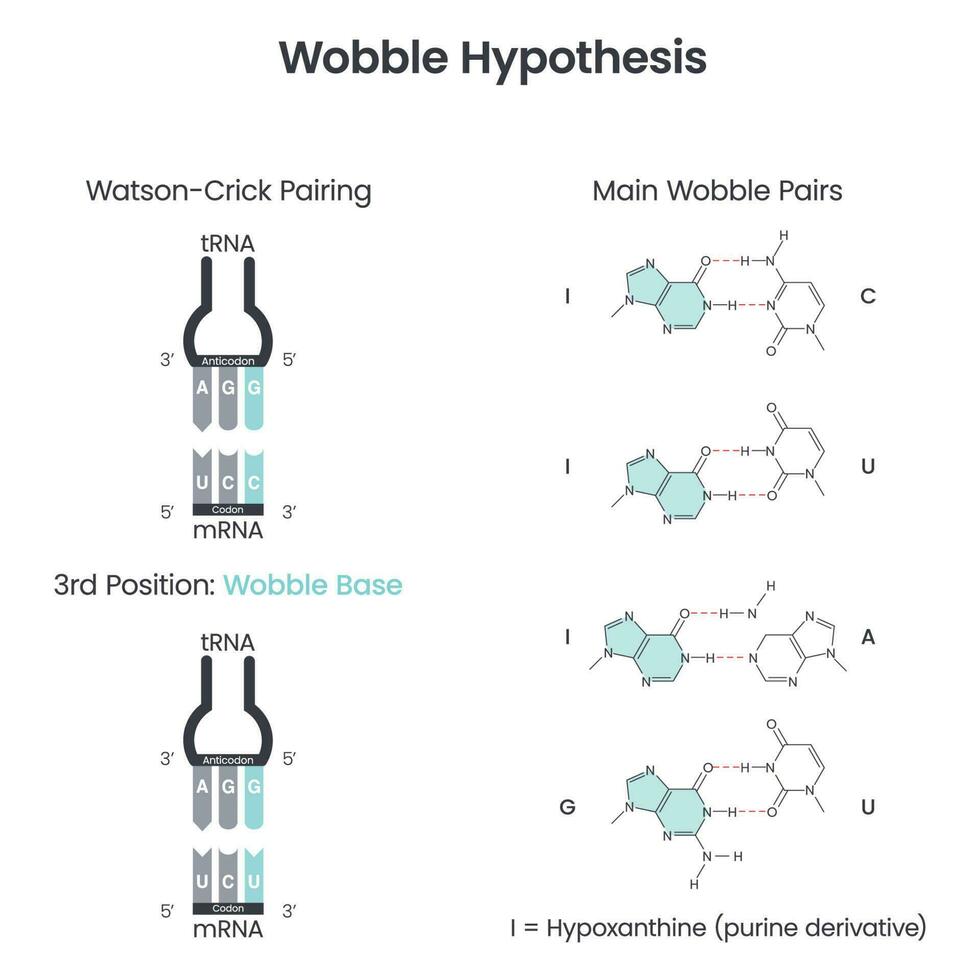
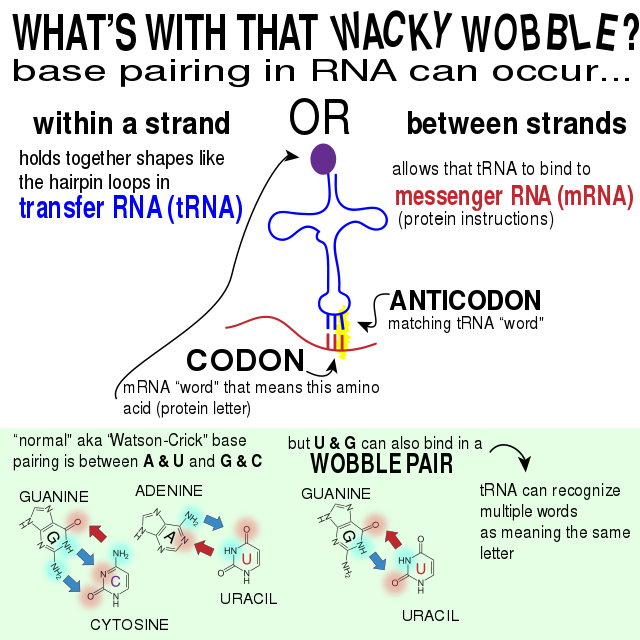
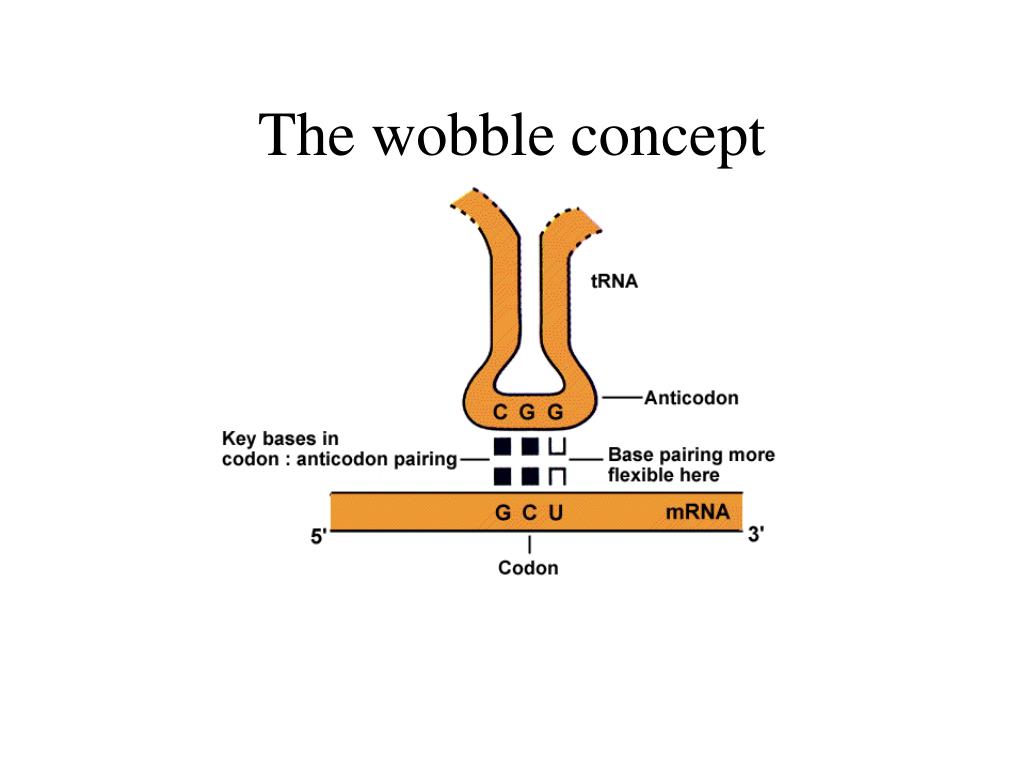
The genetic code uses three-nucleotide codons to specify amino acids during translation. There are 64 possible codons but only about 45-60 distinct tRNA types in most organisms. The math doesn't add up unless you account for non-standard base pairing at the third codon position. That mechanism is wobble, first proposed by Francis Crick in 1966, and it explains how a single tRNA can recognize multiple synonymous codons. What Is Wobble In Biology — at its core, it refers to relaxed pairing rules at the third position of the mRNA codon (positions 1 and 2 maintain strict Watson-Crick geometry). The wobble position is the 5' end of the anticodon on the tRNA, which pairs with the 3' end of the codon on the mRNA. Because the ribosome's A-site is more permissive here, certain non-canonical pairs form without disrupting the reading frame or stalling translation. The standard wobble pairs are: G in the anticodon wobble position can pair with either U or C in the codon. U in the anticodon can pair with A or G. Inosine (I), which is a modified adenine found in many tRNAs, is the most flexible — it can pair with U, C, or A. Modified uridines like queuosine (Q) or 5-methoxyuridine (mo5U) expand pairing capacity further. These modifications are added by specific enzymes after the tRNA is transcribed, and losing them through mutation or stress dramatically reduces translation efficiency.
I ran into this problem directly when I was designing synthetic codon-optimized genes for expression in E. coli. I blindly followed a standard codon usage table and assumed the software had accounted for tRNA availability. The construct expressed at less than 5% of expected levels. I spent about three weeks troubleshooting before I realized the issue wasn't promoter strength or mRNA stability — it was that my optimized sequence happened to cluster several rare arginine codons (AGA and AGG) back-to-back, and the host strain didn't carry enough ArgU tRNAs to handle the demand. Switching to a Rosetta or BL21-CodonPlus strain fixed it immediately. Wobble matters less when your organism has the right tRNAs to match whatever codon combination you throw at it, but if you're doing something non-standard, the wobble rules become the bottleneck. Here's something most textbooks don't emphasize: wobble isn't just about degeneracy. It actively shapes the fidelity of translation. The ribosome checks geometry at positions 1 and 2 of the codon-anticodon helix but not at position 3. This means misincorporation rates at the wobble position are genuinely higher — perhaps 1 in 100 to 1 in 1,000 depending on the organism and context. Most of the time this is harmless because the wobble pairs still encode the same amino acid. But when a near-cognate tRNA slips through, it causes missense errors that can aggregate into misfolded proteins. Cells counter this with quality control pathways like the ribosome-associated quality control (RQC) complex and chaperone systems, but these come at an energetic cost that scales with error rate. Another overlooked point is that wobble rules vary significantly between organisms. Bacterial systems generally follow the classical Crick wobble model fairly strictly. Eukaryotes, especially mammals, use far more elaborate modifications at the wobble position — there are over 30 known nucleoside modifications at position 34 of tRNAs. Some of these, like L-nucleosides or thiolated uridines, actually restrict pairing rather than expand it, serving as a fidelity checkpoint. The same codon will have different decoding efficiencies across species because the available tRNA modifications differ.
There are real limits to what wobble can do. It doesn't work well when you're dealing with frameshift-prone sequences or when RNA secondary structure occludes the wobble position. I've seen people try to use wobble-based degeneracy in primer design for PCR and end up with off-target amplification because they underestimated how much mismatch tolerance existed at the 3' end of primers. The wobble zone in a primer is precisely where you need the most stringency, not the least. If you're designing degenerate primers, put the degeneracy at the 5' end and keep the 3' terminal bases strictly matched. In practical terms, understanding wobble means you stop treating the genetic code as a rigid one-to-one mapping and start thinking about it as a constrained many-to-one system with biological tradeoffs baked in. The redundancy isn't an accident — it's what allows organisms to tolerate mutations at the third codon position without changing the protein. That's why silent mutations aren't always silent, and why codon optimization is more nuanced than swapping in preferred codons without considering the tRNA modification landscape and the cellular economy of tRNA synthesis.
Get the Full Details