Molecule Transport Across Cell Membranes: What Actually Gets Through
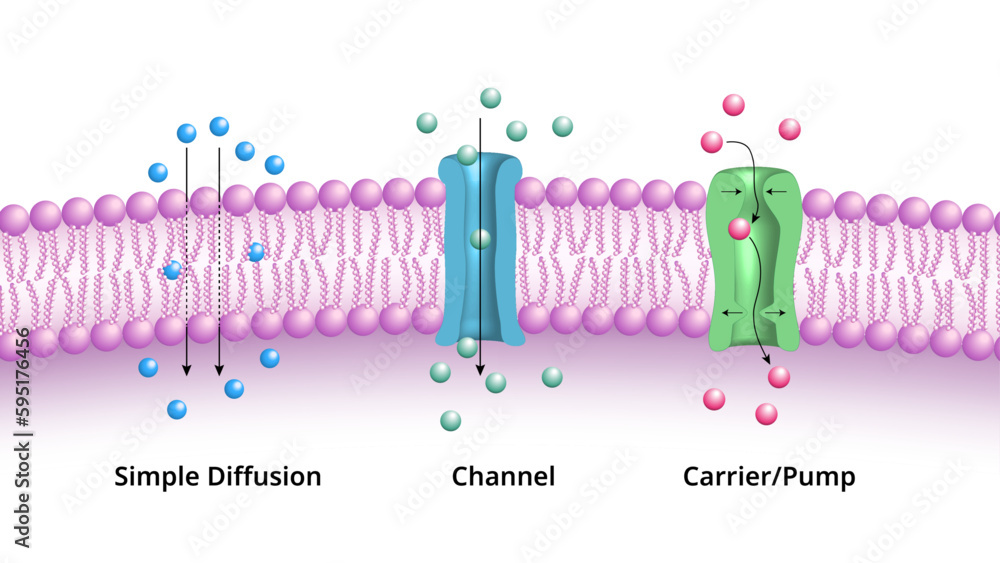
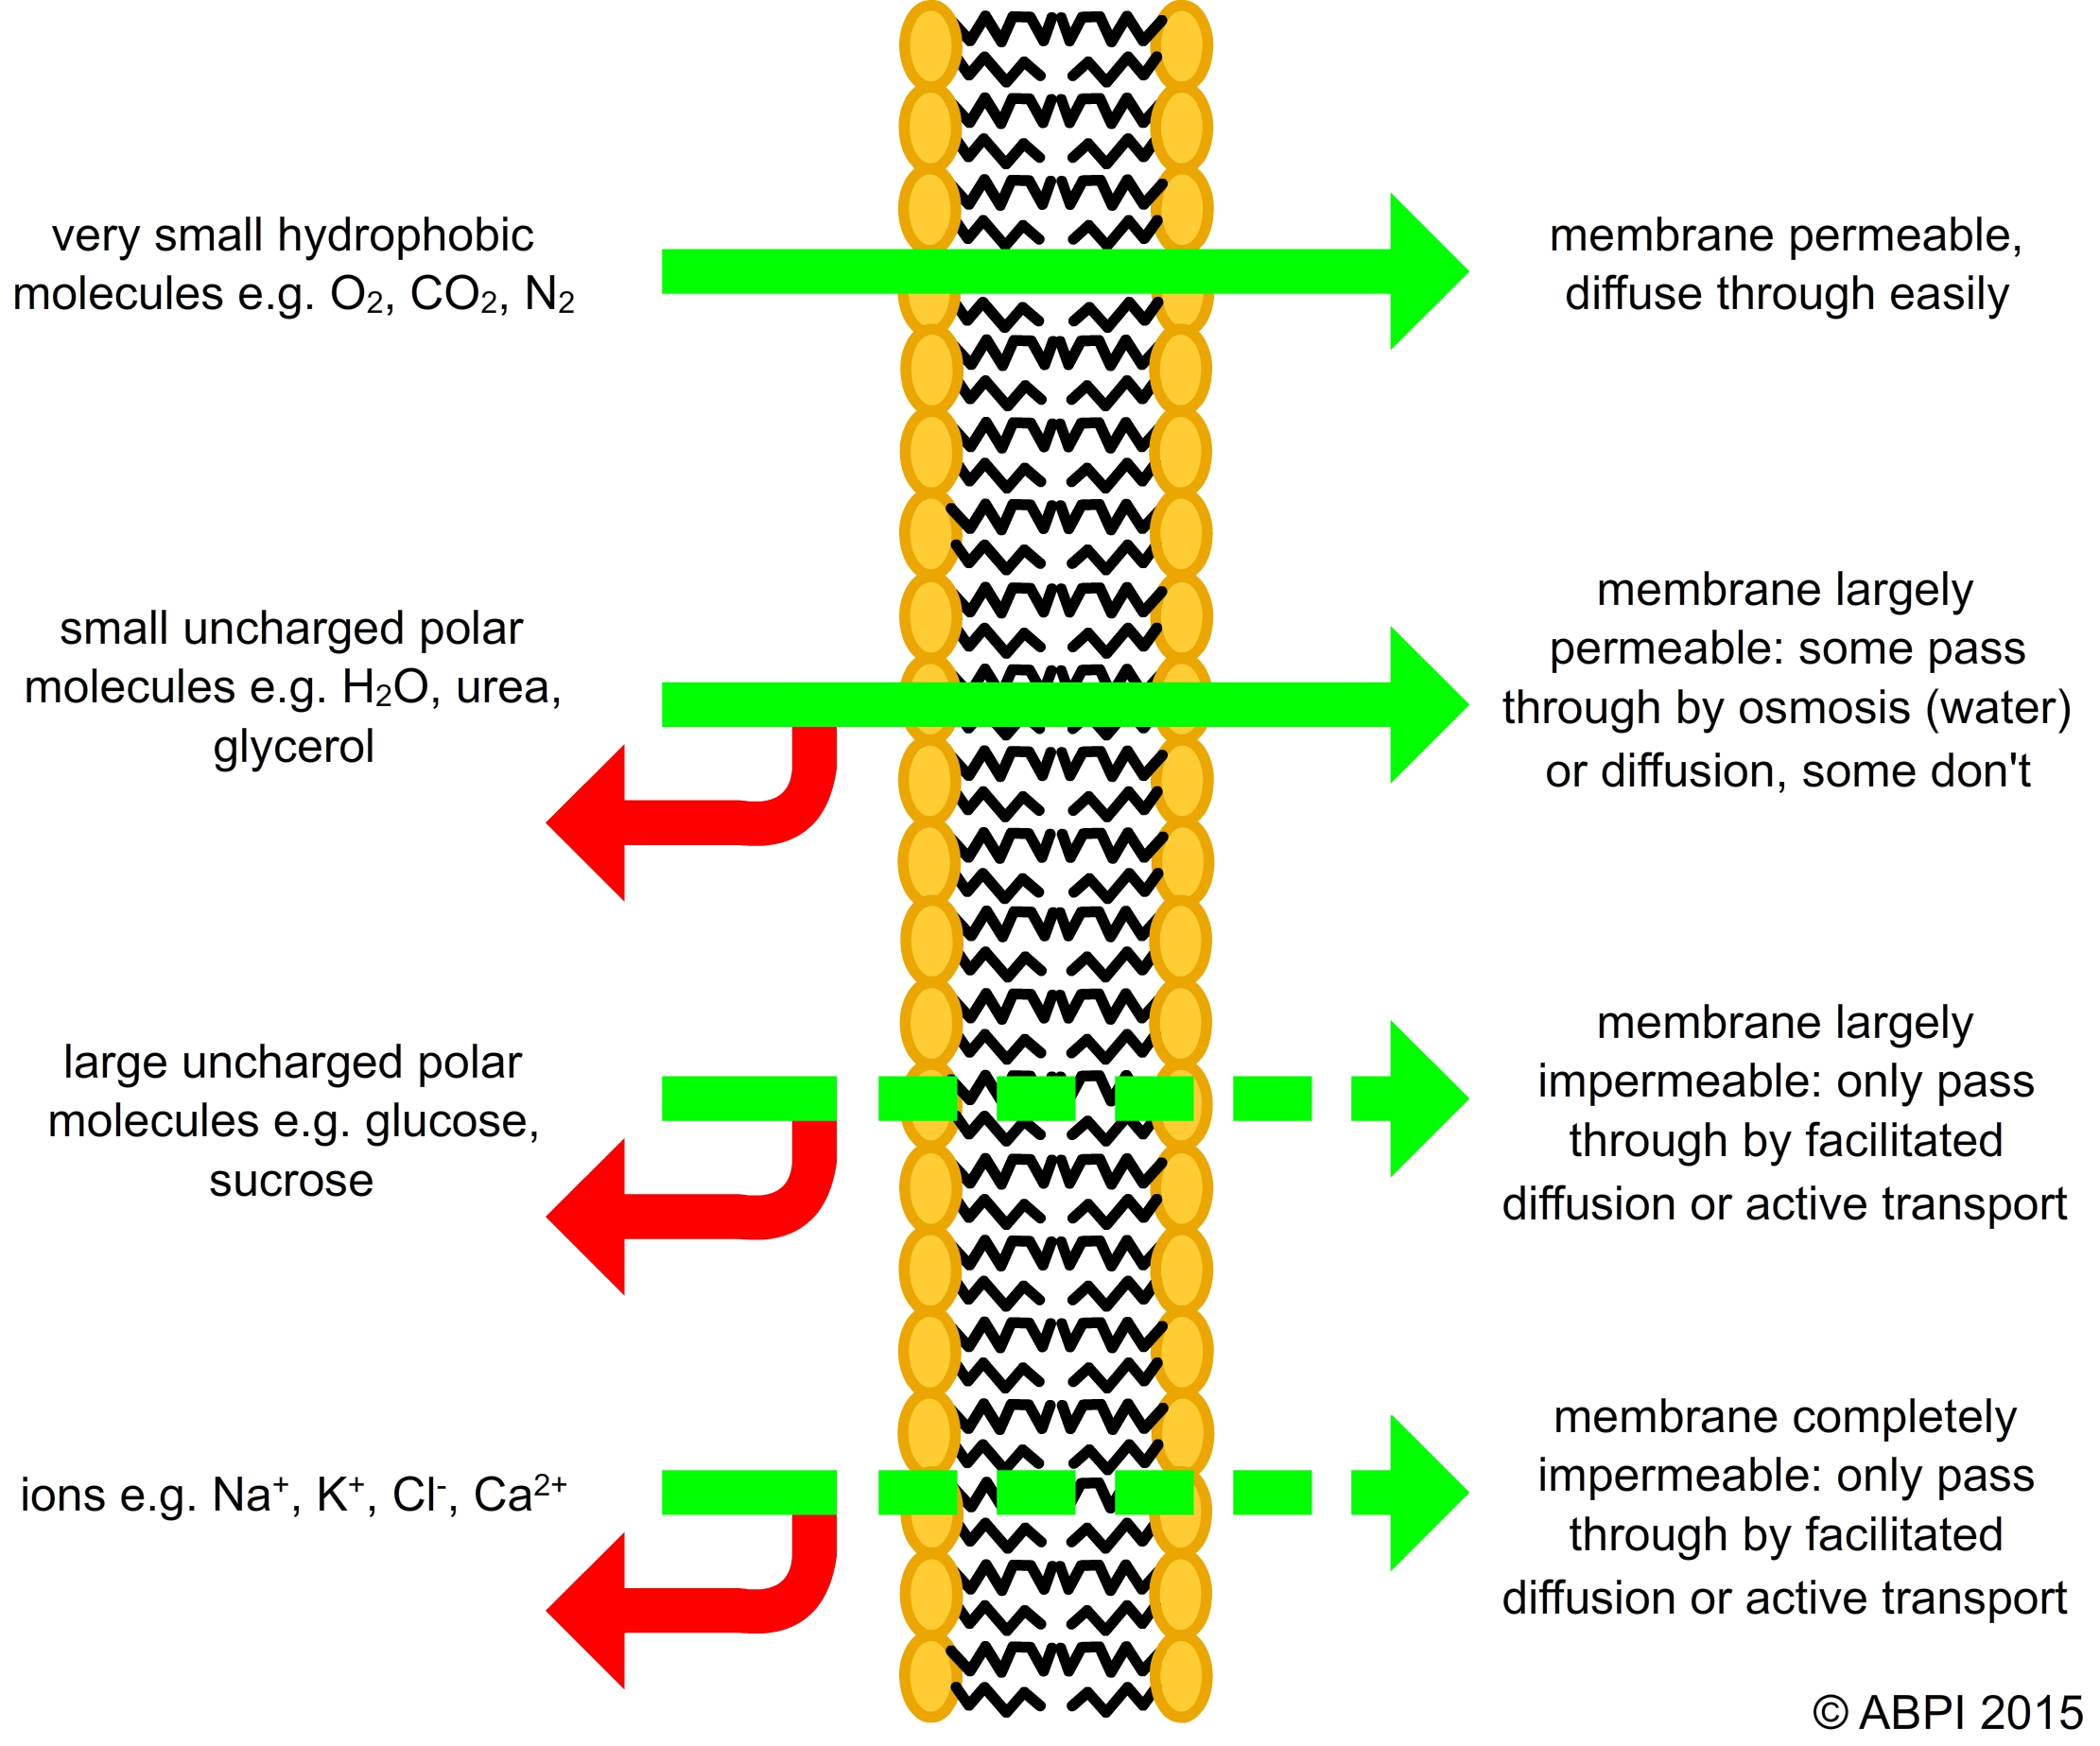
Most people learn diffusion in biology class and then never really understand it afterward. You memorize that small nonpolar molecules cross freely, large polar ones don't, and ions are blocked entirely. Then you hit a real lab scenario and realize your understanding was way too simplified. Here is what actually happens.The core mechanism of simple diffusion through a lipid bilayer depends on three things: molecule size, polarity, and charge. A molecule needs to be small enough to slip between phospholipid tails and nonpolar enough to dissolve into that hydrophobic core without getting rejected. That is the basic rule, but the exceptions are where it gets interesting. Small nonpolar molecules are the clear winners here. Oxygen and carbon dioxide glide right through without any assistance. Nitrogen does the same. These are gases at room temperature and their tiny molecular weight means they zip across membranes at rates that depend mostly on the concentration gradient on either side. I have measured O2 flux in cell suspensions and the numbers match what Fick's law predicts almost exactly when the cells are healthy and the membrane is intact. Small uncharged polar molecules can cross too, but with caveats. Water is the big one. It crosses through the bilayer itself, just much more slowly than you might expect, and organisms use aquaporins to speed things up dramatically when they need to. Ethanol and urea also make it through via simple diffusion. Glycerol is borderline — small enough in theory but polar enough that it moves quite slowly without transport proteins helping it along.
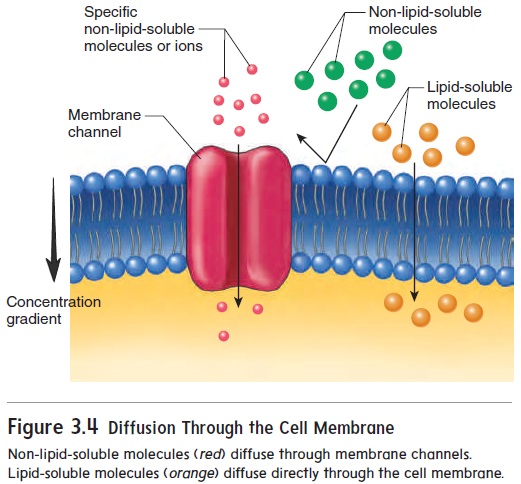
Lipid-soluble molecules are another category worth noting. Steroid hormones like testosterone, estrogen, and cortisol are all small enough and nonpolar enough to diffuse directly through the membrane. That is why they do not need surface receptors — they get inside the cell and bind to intracellular receptors instead. This is functionally important and often tested, so pay attention to it. Charged ions and large polar molecules like glucose and amino acids cannot cross by simple diffusion at any meaningful rate. The hydrophobic interior of the membrane is essentially a wall to them. They need channels, carriers, or pumps. Endothelin, for instance, is far too large and polar to slip through on its own. Here is something most textbooks gloss over: the concept of "small enough" is not a fixed number. A molecule around 100 Daltons or less tends to cross reasonably well if it is also nonpolar. But once you get past roughly 200 Daltons, even a nonpolar molecule starts having trouble. I worked with a compound around 180 Daltons that was mostly nonpolar and it still crossed far slower than expected because of subtle polar groups on its surface. Molecular weight charts give you a general idea, but surface chemistry matters just as much.
Another thing people miss is that temperature affects diffusion rates significantly. Raise the temperature and the phospholipids gain kinetic energy, the membrane becomes more fluid, and molecules cross faster. Drop it and things slow down. I ran an experiment where I compared O2 diffusion at 37 degrees Celsius versus 25 degrees and the rate dropped by roughly forty percent. The membrane had literally become tighter and more ordered at the lower temperature. Membrane composition also plays a role that beginner courses rarely emphasize. Cholesterol content changes membrane fluidity. More cholesterol at body temperature makes the membrane less fluid and slightly harder for molecules to penetrate. At low temperatures, cholesterol actually prevents the membrane from becoming too rigid, which maintains some level of permeability. Saturated fatty acid tails pack tighter and reduce permeability compared to unsaturated tails with their kinks. If you are working with cells and notice unexpected permeability changes, check what the cells have been fed — the lipid composition of their membranes adapts to their environment. My own experience with this came when I was troubleshooting a drug delivery project. We had a candidate molecule that looked perfect on paper — small, mostly nonpolar, should diffuse right through cell membranes. It did not work in practice. Turns out the molecule had a lone hydrogen bond donor that made it interact unfavorably with the hydrophobic core despite its overall nonpolar appearance. We spent three weeks trying to figure out why the cellular uptake was ten times lower than predicted before we realized the issue. The workaround was adding a methyl group to block that problematic position, which increased membrane permeability by about fivefold. Simple structural tweak, huge functional difference.
Get the Full Details
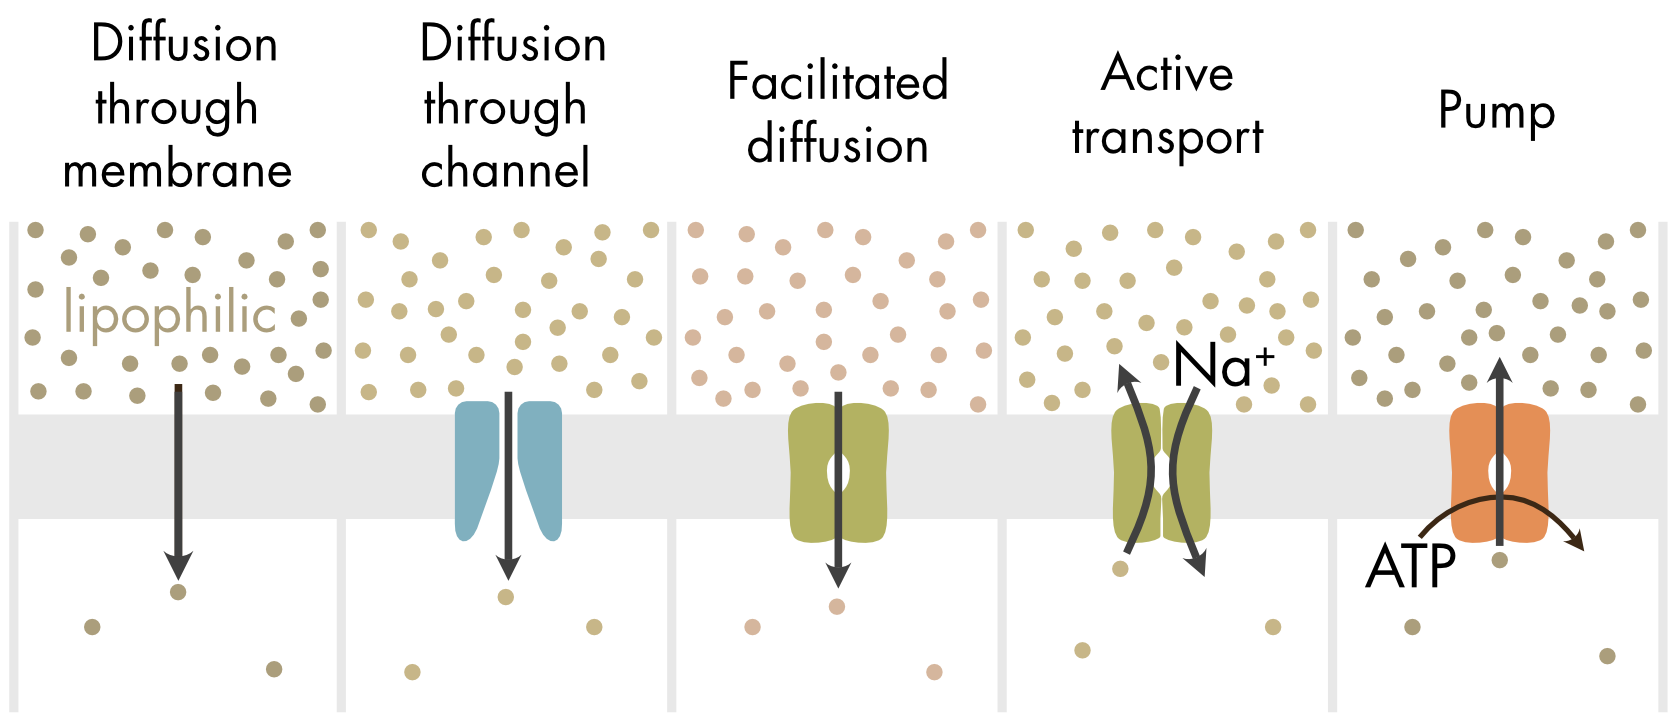
Facilitated diffusion is a separate mechanism from simple diffusion and it is important not to conflate them. Facilitated diffusion still moves molecules down their concentration gradient without energy input, but it requires a protein — either a channel or a carrier. Glucose enters cells this way via GLUT transporters. Aquaporins facilitate water movement. The molecules move faster than they would by simple diffusion alone, but the driving force is still just the concentration gradient. No ATP required. Active transport is completely different. It moves molecules against their gradient and requires energy, usually from ATP hydrolysis. The sodium-potassium pump is the classic example, moving three sodium ions out and two potassium ions in per cycle. This is not diffusion at all, but students frequently mix it up because all three processes involve molecules crossing membranes. There is a practical limitation worth acknowledging: simple diffusion only works effectively over very short distances. In a cell, the membrane is thin enough — about five nanometers — that diffusion across it is nearly instantaneous. But if you are talking about diffusion through tissue or across a thick barrier, the time scale changes dramatically. A molecule might cross a membrane in microseconds but take hours to diffuse through a millimeter of tissue. This is why multicellular organisms need circulatory systems. Diffusion alone cannot support large bodies.
Another limitation is that simple diffusion cannot concentrate molecules. It only moves things from high to low concentration until equilibrium is reached. If a cell needs to accumulate a substance against a gradient, simple diffusion will never accomplish that. You need active transport for that. This is a fundamental constraint and it applies to every living system. The rate of diffusion across a membrane follows Fick's first law, which relates flux to the concentration gradient, the diffusion coefficient, the membrane area, and membrane thickness. The equation is straightforward: flux equals the diffusion coefficient times the area times the concentration difference divided by the thickness. In practice, the diffusion coefficient varies enormously depending on the molecule and the membrane composition, so predictive calculations often require empirical measurement rather than theoretical estimation. I should also mention that some molecules cross by a mechanism called transcytosis, which involves vesicle formation and fusion. This is neither simple diffusion nor facilitated diffusion and it is used for large molecules like proteins and peptides. Insulin crossing the blood-brain barrier is an example, though the specific transporter involved is still debated in the literature.
If you are studying this for an exam, focus on the categories: small nonpolar gases pass freely, small uncharged polar molecules pass slowly, lipids and steroid hormones pass readily, and everything charged or large is blocked without assistance. For practical lab work, remember that membrane composition, temperature, and subtle molecular features like hydrogen bonding capacity can all shift permeability in ways that pure textbook rules do not predict.