Understanding Passive Movement Across Membranes
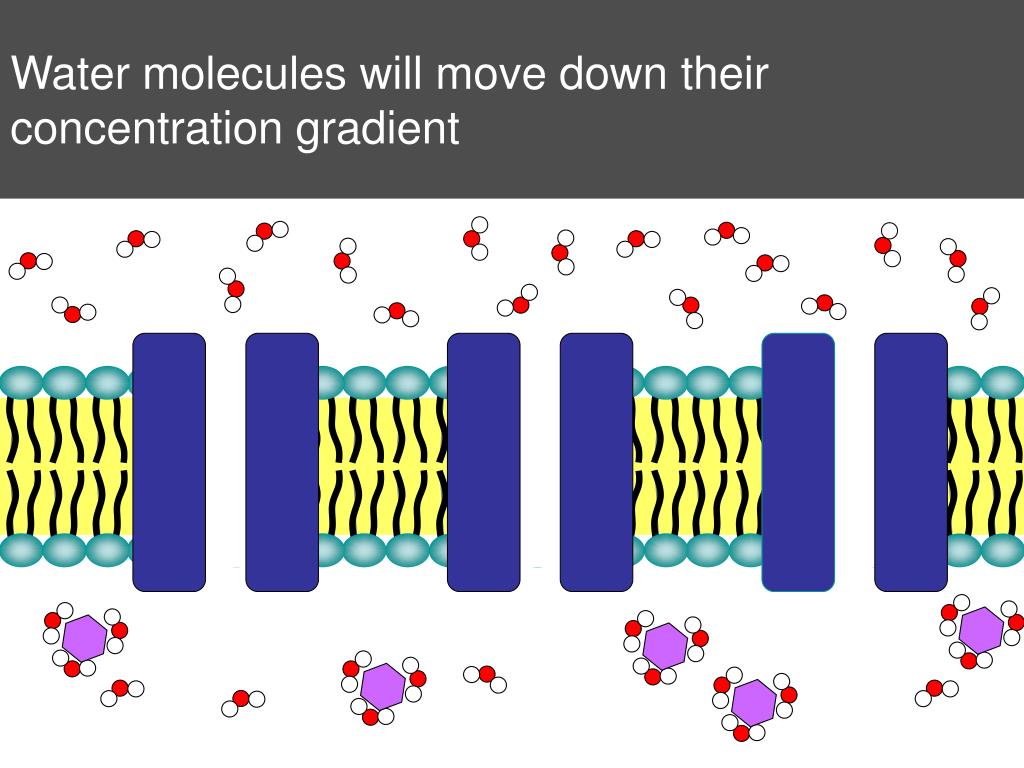
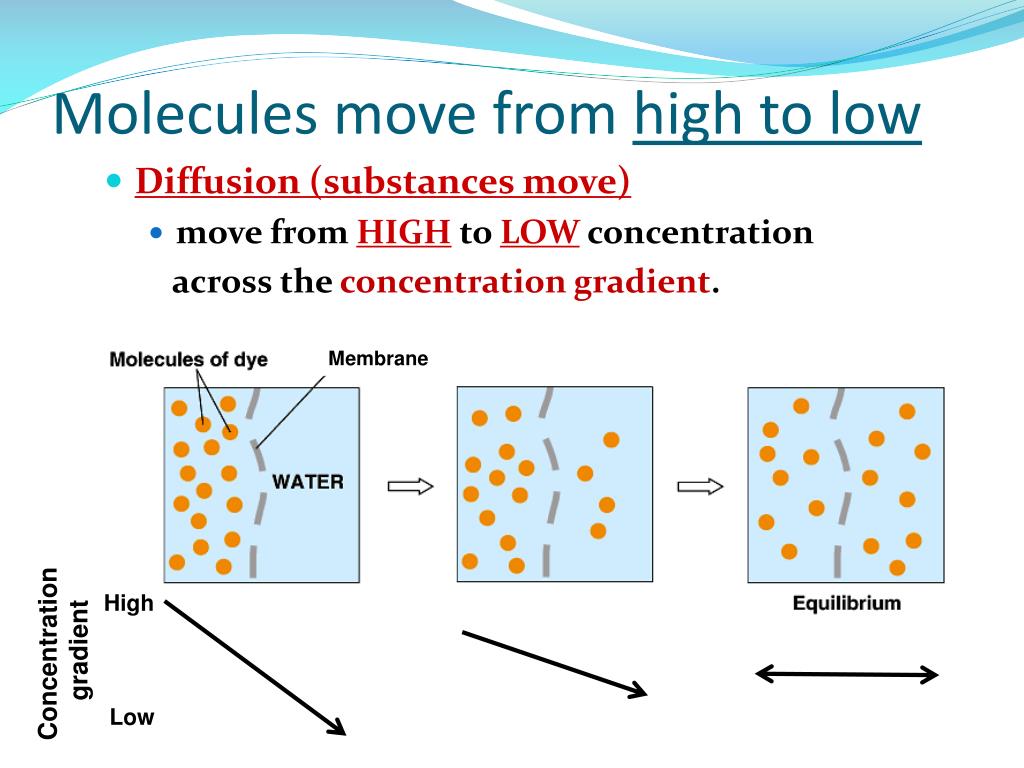
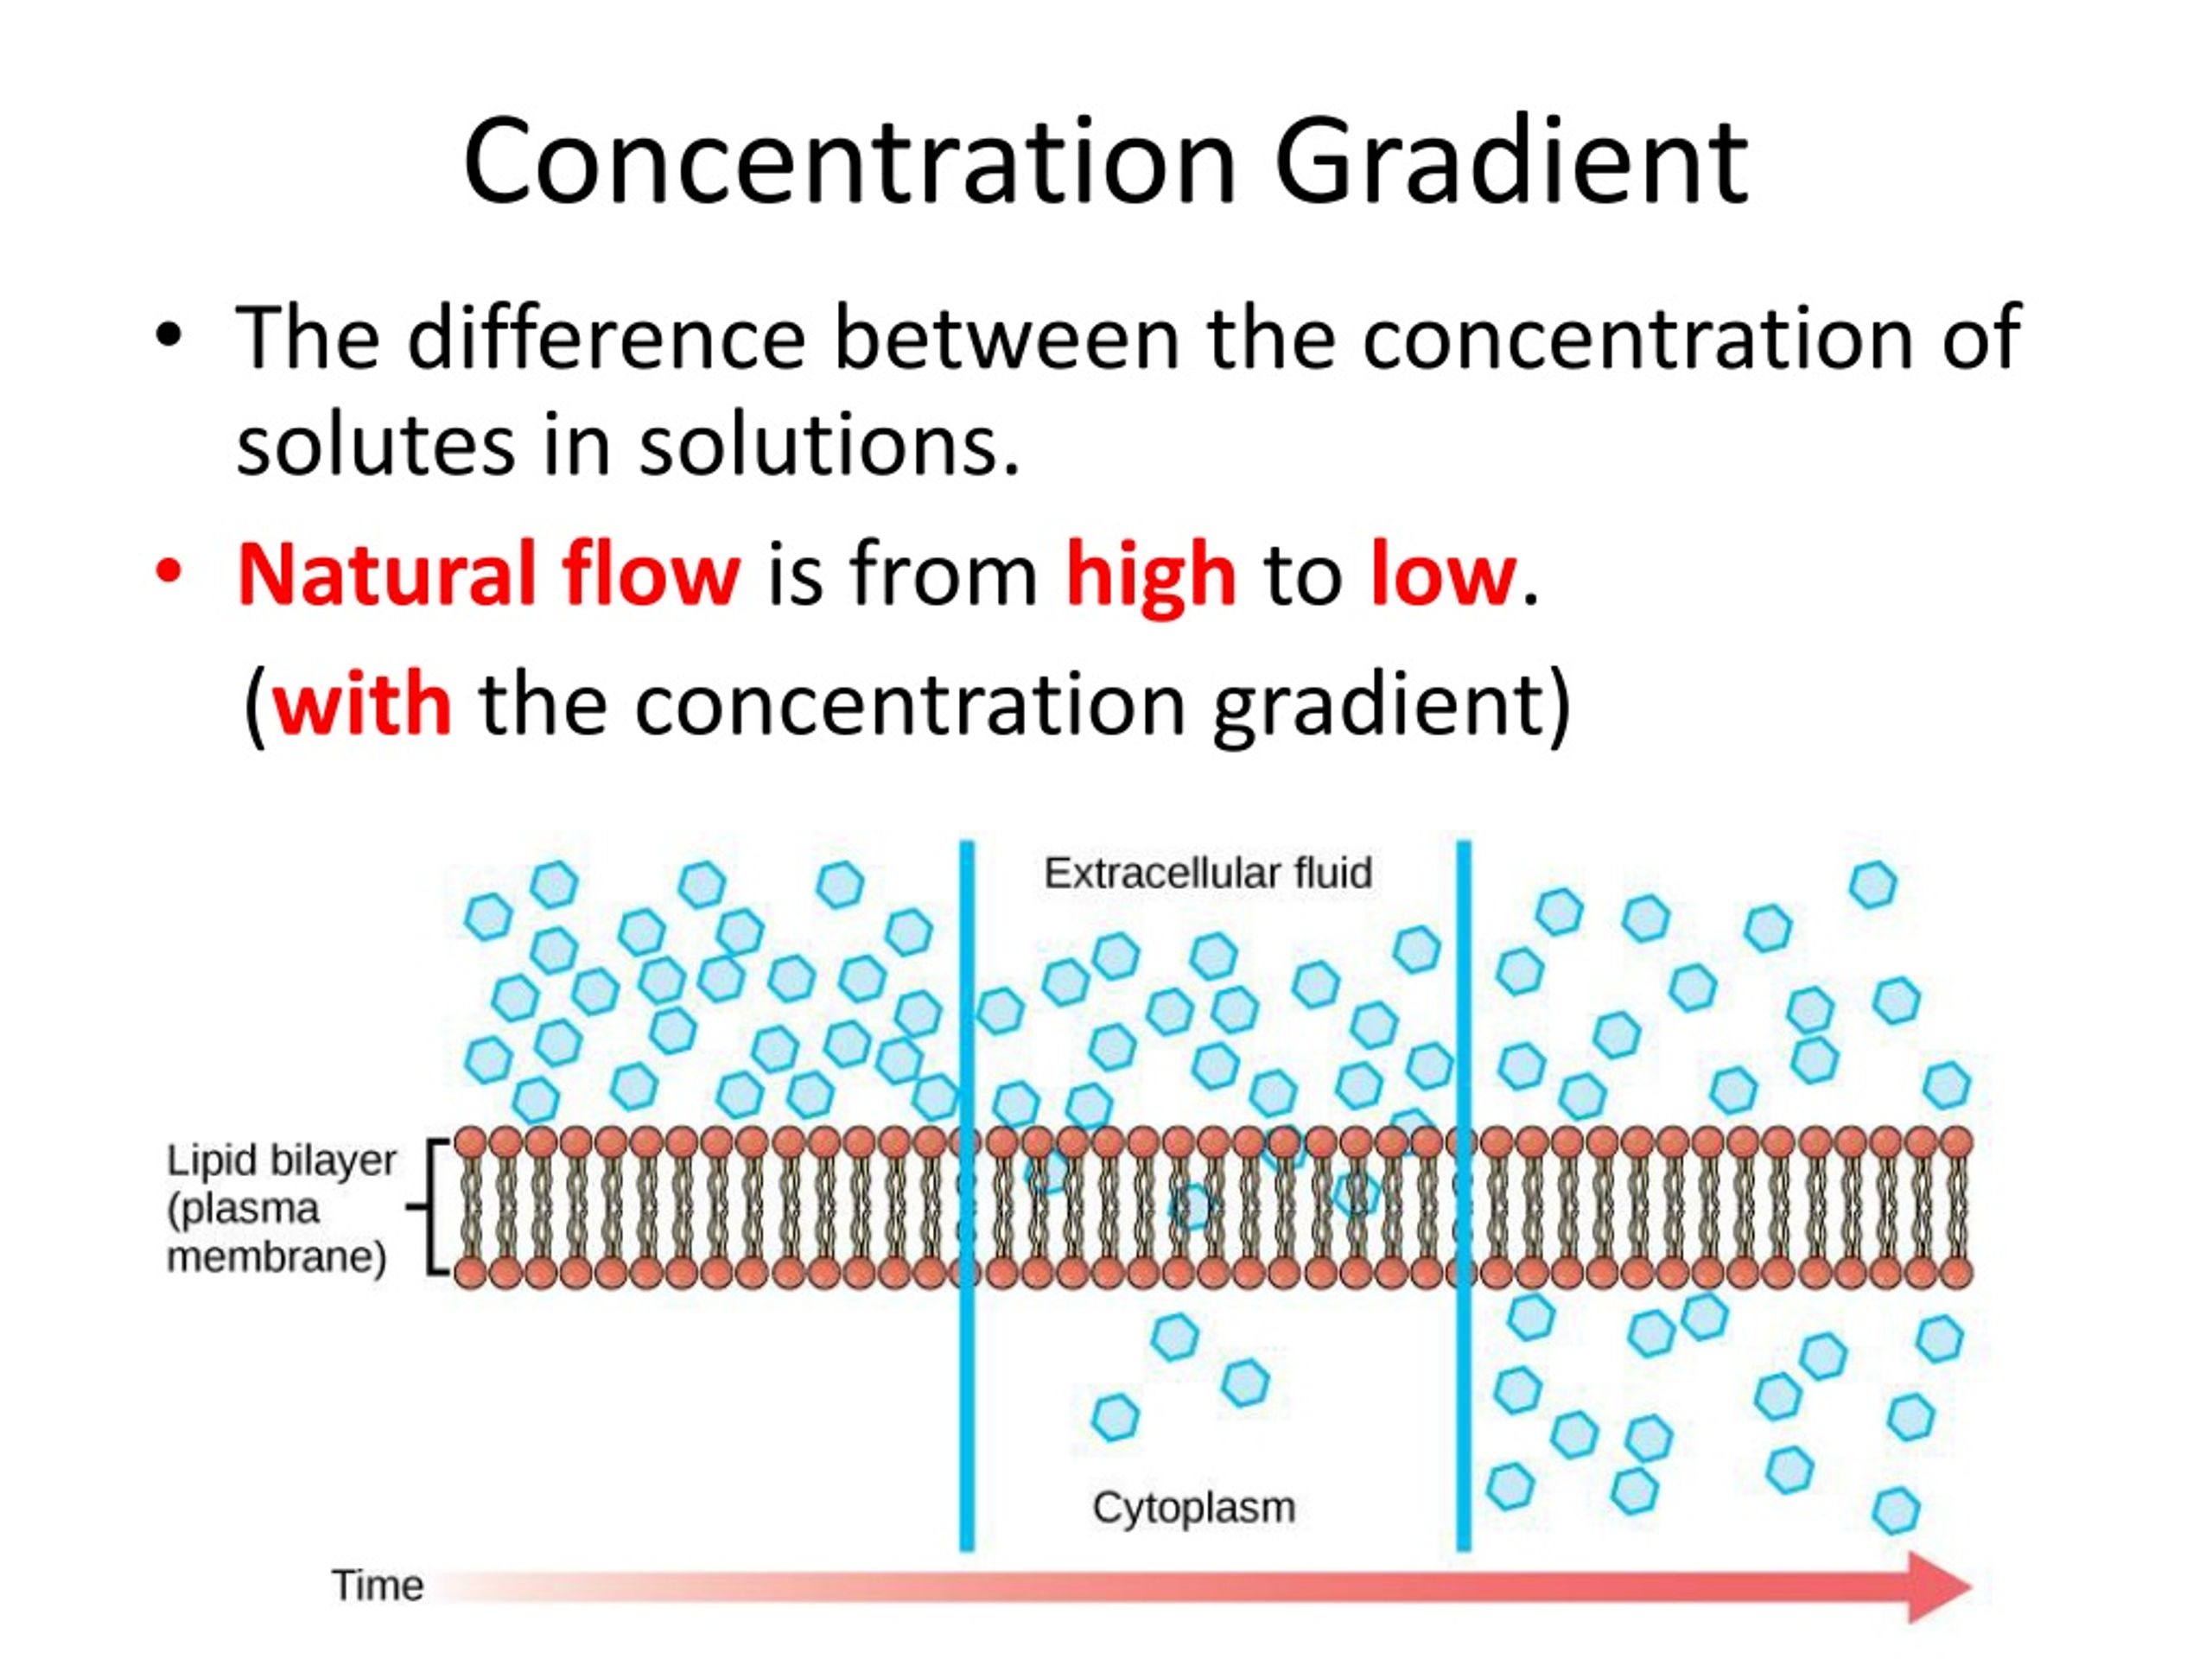
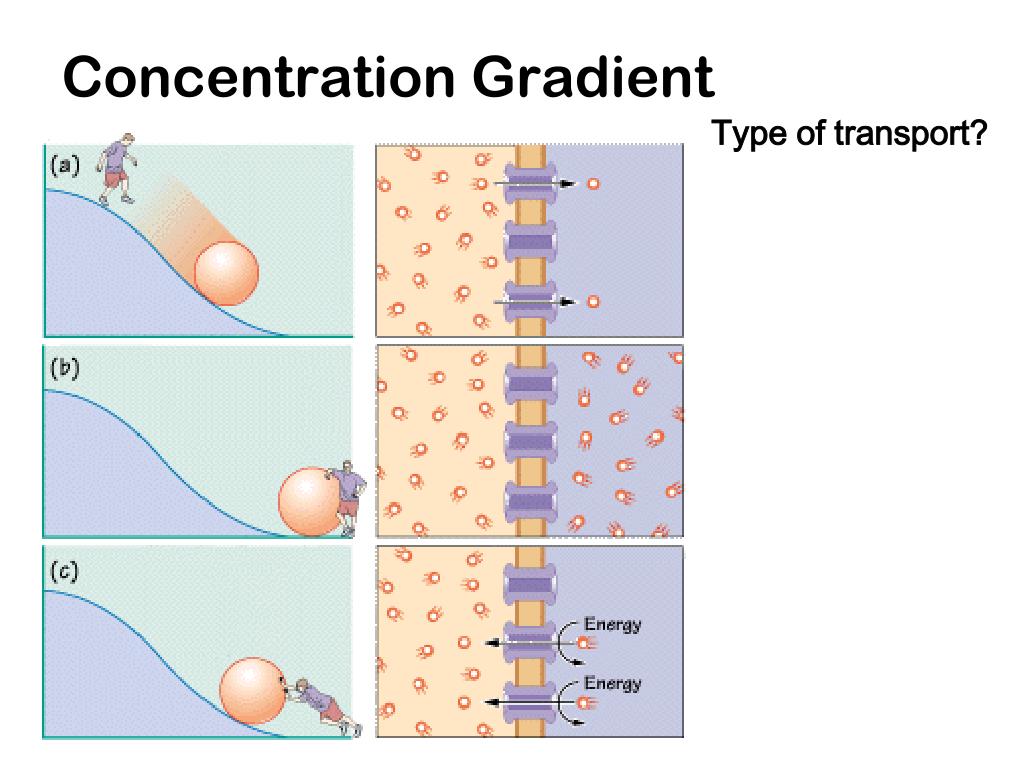
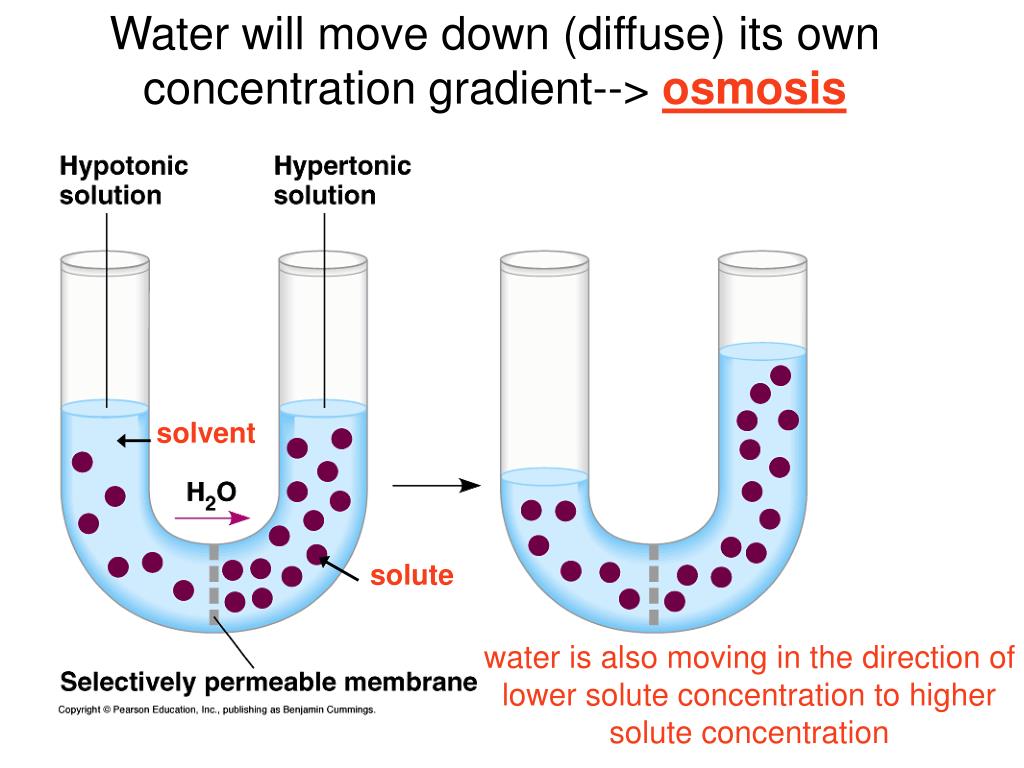
Molecules moving down their concentration gradient is the simplest mechanism cells use to exchange materials. No energy input required. The solute just travels from wherever it is more concentrated to wherever it is less concentrated until equilibrium is reached. That is it. It sounds trivial but people constantly overcomplicate it in lab settings and on exams. This is called passive transport, and there are two main types. Simple diffusion happens when small nonpolar molecules like oxygen or carbon dioxide slip straight through the lipid bilayer. Facilitated diffusion is what happens when larger or charged molecules need a helping hand from a channel or carrier protein. Glucose entering a cell through GLUT4 is a classic example. Water is its own category in many textbooks — osmosis — but it is still moving down a concentration gradient of water itself, from low solute concentration to high solute concentration. I spent three weeks troubleshooting why a fluorescence recovery after photobleaching assay kept giving inconsistent permeability values for a membrane protein I was studying. The problem turned out to be that the buffer's ionic strength was shifting the surface potential near the membrane, which subtly altered the effective concentration gradient without changing the bulk measurement. I ended up switching to a lower-salt buffer and re-running everything. The FRAP curves normalized within two days of doing that. Most people would have just blamed pipetting error or protein degradation. The gradient on the membrane surface is not the same as the gradient in the beaker.
The Mechanism in Practice
Here is how it actually works at the molecular level. Molecules are in constant random thermal motion. In a region of high concentration, there are simply more molecules bouncing around. Statistically, more of them will cross into the low-concentration region than vice versa. Net movement occurs. Not because the molecules "know" where they need to go. Because probability favors the direction from crowded to sparse. The rate of diffusion depends on several factors. Temperature matters — higher temperature means more kinetic energy and faster movement. Molecular size matters — bigger molecules move slower. The steepness of the gradient matters — a larger difference in concentration produces faster net movement. And for facilitated diffusion, the number and availability of transport proteins is the limiting factor, not the gradient itself. Once all the carriers are saturated, adding more solute outside the cell does nothing to increase the rate. I once had a student run a transport experiment where they doubled the external glucose concentration and expected double the uptake rate. It did not happen. The transporters were already working at Vmax. This is one of those things that is intuitive until you actually look at the data. Saturation kinetics are real and they show up in every facilitated diffusion system. If your rate plateaus while the gradient is still increasing, you are hitting transporter capacity, not breaking the model.
Where People Get It Wrong
The biggest misconception is that equilibrium means molecules stop moving. They do not. At equilibrium, molecules are still crossing the membrane in both directions. The net flux is zero because the rates are equal. Think of it as a busy doorway where as many people exit as enter. The crowd density stays constant even though individuals are constantly swapping sides. Another common mistake is confusing this with active transport. Active transport moves molecules against their gradient and requires ATP or some other energy source. Passive transport never does that. If you see a pump involved, it is active. If you see a channel or carrier with no energy input, it is passive. The distinction matters because the thermodynamics are completely different. Downhill movement releases free energy. Uphill movement consumes it. Fick's laws of diffusion give you the mathematical framework. The first law states that flux is proportional to the concentration gradient and the diffusion coefficient. The second law describes how concentration changes over time in a given space. In a lab setting, if you need to predict how long it takes for a substance to diffuse across a known distance, you can plug numbers into these equations. For cell-scale distances on the order of micrometers, diffusion is fast — milliseconds to seconds for small molecules. For anything larger than a millimeter, passive diffusion alone is insufficient, which is why multicellular organisms evolved circulatory systems.
Get the Full Details
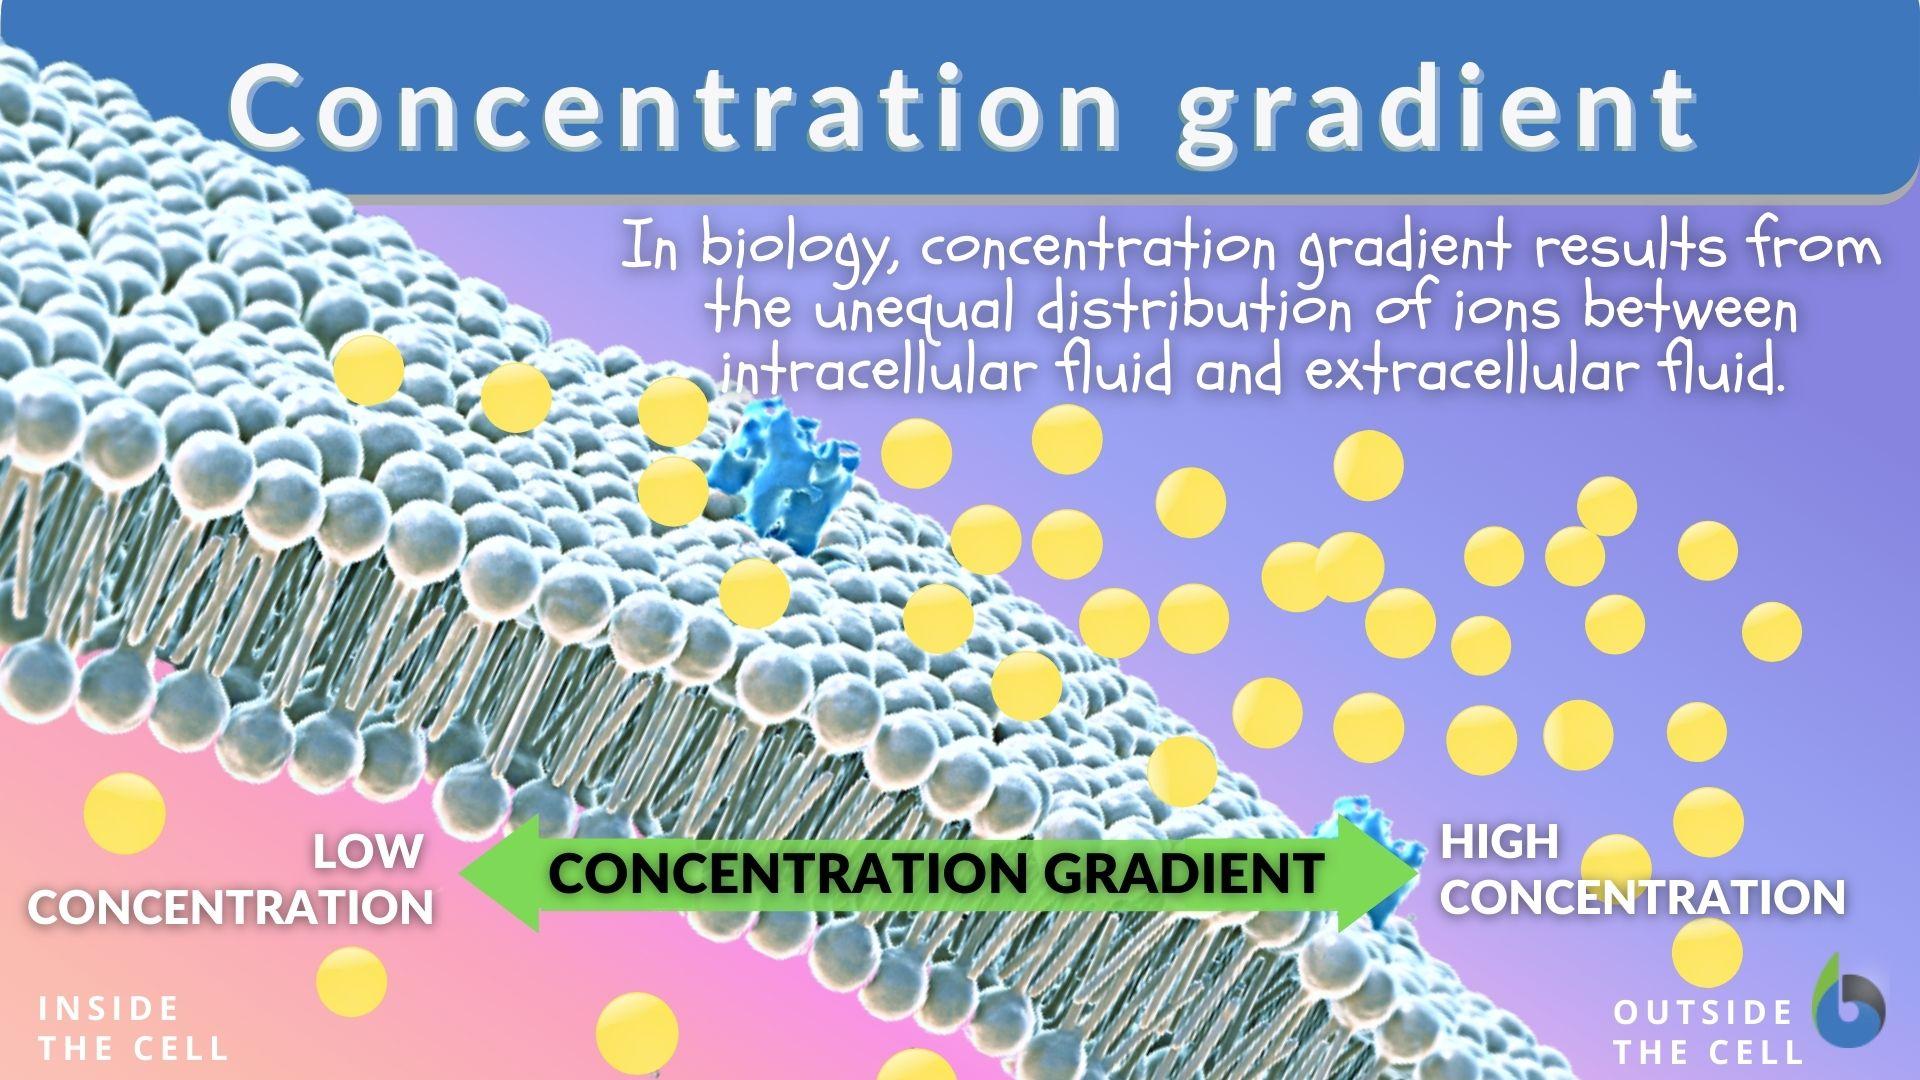
There is also the matter of membrane composition. A membrane rich in cholesterol is less fluid and slows diffusion of small molecules through the bilayer. Saturated fatty acids do the same. Unsaturated fatty acids with kinks in their tails keep things looser and allow faster passage. If you are comparing transport rates across different cell types, the lipid environment is a variable you cannot ignore. Ion channels add another layer of complexity. Even though ions are moving down their electrochemical gradient, the electrical component matters. A positive ion might be attracted into a cell by a negative membrane potential even if its concentration is already higher inside. The Nernst equation quantifies the equilibrium potential for any given ion. When the membrane potential equals the Nernst potential for that ion, there is no net movement regardless of what the concentration gradient says. This is why saying "down the concentration gradient" is sometimes incomplete. It is down the electrochemical gradient that really matters for charged species.
Real Applications
Oxygen delivery in the lungs is essentially passive diffusion from alveoli into capillary blood. Carbon dioxide exits blood into alveoli the same way. Gas exchange in your lungs right now is happening without any cellular energy expenditure on the part of the gases themselves. The blood flow and ventilation maintain the gradients, but the actual crossing of the respiratory membrane is purely downhill. Drug delivery systems exploit this principle. Lipid-soluble drugs pass through membranes by simple diffusion. That is why formulation chemists care so much about lipophilicity. A drug that cannot cross the lipid bilayer will not reach its intracellular target regardless of how potent it is. PEGylation and other modifications that reduce membrane permeability are intentional choices made to keep certain therapeutics in the bloodstream longer. In experimental biology, measuring permeability coefficients is standard practice. You set up a barrier with known concentrations on each side, monitor concentration change over time, and calculate the permeability coefficient P from the slope. This number tells you how readily a substance crosses a particular membrane. It is used in everything from designing controlled-release formulations to predicting how toxic compounds enter cells. The method is straightforward but getting reliable data requires tight control of temperature and stirring conditions. Unstirred layers near the membrane can become rate-limiting and make a highly permeable substance appear less permeable than it actually is.
I have seen this artifact ruin data sets before. A thin layer of stagnant solution next to the membrane acts as an extra barrier. Agitating the solution reduces the unstirred layer thickness and usually increases the apparent permeability. If you are comparing permeability values from different papers, check whether they reported stirring rates. Differences in hydrodynamics can account for orders of magnitude variation between studies that are otherwise measuring the same thing.
Limitations to Keep in Mind
Passive transport only works when a gradient exists. Remove the gradient and the net movement stops. Cells expend significant energy maintaining concentration differences across their membranes precisely because those gradients are useful. Sodium and potassium gradients power nerve impulses. Proton gradients drive ATP synthesis. All of it rests on the fact that you can build up a gradient and then let molecules flow back down it in a controlled manner. The process also cannot concentrate a substance beyond the starting level. If you want molecules on the dilute side to accumulate to a higher concentration than on the source side, you need active transport. Passive mechanisms will always equalize, never amplify. This is a hard thermodynamic constraint, not a technical limitation that better technology can overcome. For large polar molecules and ions, simple diffusion through the lipid bilayer is effectively impossible. The hydrophobic core repels them. They require protein-mediated pathways. And those pathways have finite capacity. If a cell needs to absorb massive amounts of a nutrient quickly, it may upregulate the expression of transport proteins rather than relying on the existing complement. This is a regulatory response that connects passive transport mechanics to gene expression, which is worth keeping in mind when you are looking at dose-response curves that shift over hours rather than minutes.
The principle itself is foundational. Everything from oxygen breathing to neurotransmitter reuptake inhibition traces back to molecules moving from high to low concentration. Understanding it thoroughly removes the mystery from a lot of physiology and pharmacology. You do not need to memorize every transporter subtype to get value from this. You just need to recognize the pattern whenever you encounter a transport phenomenon and ask whether energy is being consumed or whether the molecule is simply going with the flow.