The Quick Answer
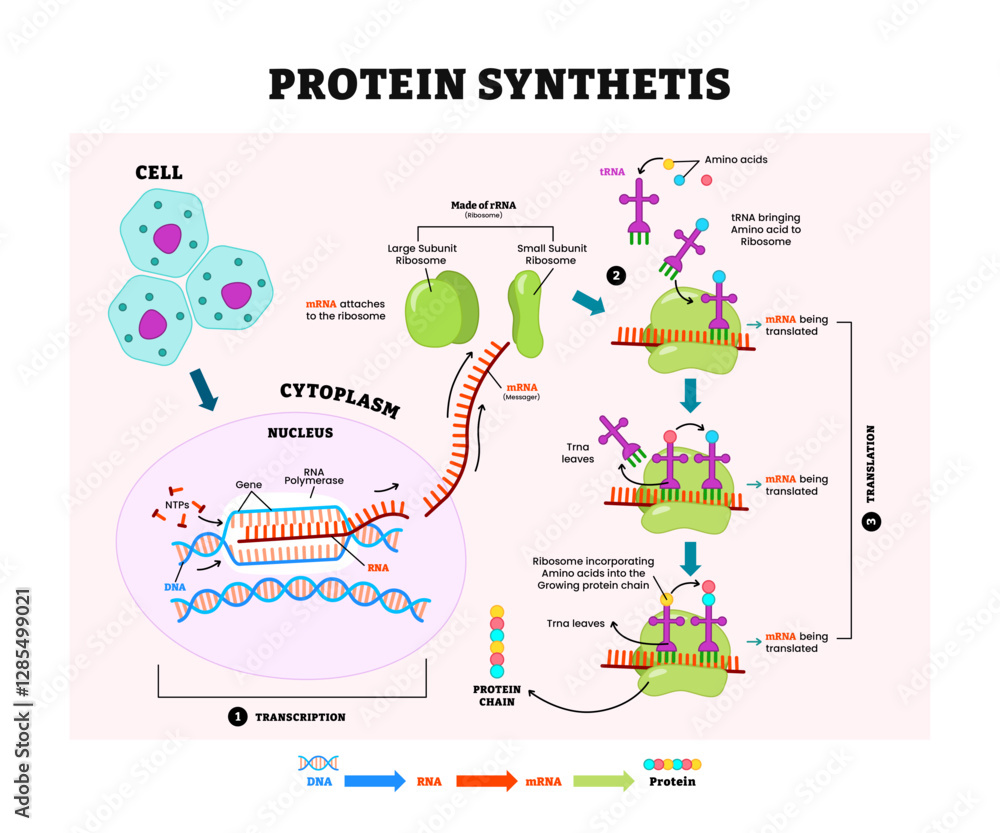
Protein synthesis happens in ribosomes. Transcription takes place in the nucleus for eukaryotic cells, then the mRNA moves out to the cytoplasm where ribosomes read it and build proteins. That's the basic map. The reality is messier than that simplified version usually lets on. Here's what you need to know if you're trying to work with this practically rather than just memorize it for a test. Translation — the actual reading of mRNA and assembly of amino acids — occurs on ribosomes. Ribosomes exist in two states. Some float freely in the cytoplasm. Others attach to the rough endoplasmic reticulum. The destination of the final protein determines which ribosome handles it. If the protein needs to go somewhere outside the cell or be embedded in a membrane, the ribosome docks onto the ER. If it stays inside the cytoplasm, a free ribosome does the work. Transcription is where it starts. RNA polymerase reads the DNA template strand in the nucleus and builds a complementary mRNA strand. The mRNA gets capped, polyadenylated, and spliced before it leaves through nuclear pores. You can't skip the splicing step cleanly. Introns have to be removed or you end up with garbled instructions downstream.
I've seen students and even some junior researchers conflate transcription and translation as if they happen at the same time in the same place. They don't. In eukaryotes they're physically separated by the nuclear envelope. Prokaryotes don't have that luxury, which is why their transcription and translation can couple together — ribosomes start assembling proteins while the mRNA is still being transcribed. That's a genuinely important difference and it's the reason certain antibiotics work on bacteria but not human cells. Things like tetracycline and erythromycin target the bacterial ribosome specifically because of structural differences in the 30S and 50S subunits compared to the 40S and 60S subunits in eukaryotes.
The Step-by-Step Process
I'll walk through it in order because the sequence matters more than people realize. First is initiation. The small ribosomal subunit binds to the mRNA near the 5' cap and scans until it finds the start codon, AUG. The initiator tRNA carrying methionine pairs with that codon. Then the large subunit joins and you have a complete ribosome ready to go. This step is where a lot of regulation happens. Availability of initiation factors, the structure of the mRNA's 5' UTR, even the presence of upstream open reading frames can all slow this down or block it entirely. If you're doing anything involving gene expression analysis, you need to account for this. It's not just a simple on switch. Second is elongation. The ribosome moves along the mRNA three nucleotides at a time. Each codon recruits a matching tRNA. Peptide bonds form between the growing chain and the incoming amino acid. The ribosome has three sites — A, P, and E — and tRNAs cycle through them. A for aminoacyl, P for peptidyl, E for exit. Simple enough until you consider that each bond formation takes roughly 15 to 20 milliseconds in a typical eukaryotic cell. That's fast, but it's also where bottlenecks show up if certain tRNAs are scarce or if the mRNA has problematic sequences.
Get the Full Details

Third is termination. The ribosome hits a stop codon — UAA, UAG, or UGA — and release factors bind instead of a tRNA. The polypeptide chain is cleaved from the tRNA in the P site. The ribosome falls apart into its subunits. The new protein may need further modification. Glycosylation in the ER, folding with chaperone assistance, cleavage of signal peptides. These post-translational steps aren't optional in most cases. A protein that hasn't been properly folded or modified is usually nonfunctional or gets tagged for degradation.
Common Pitfalls and What Actually Goes Wrong
People tend to think of protein synthesis as a straightforward assembly line. It's not. Here are some things that will trip you up. Co-translational folding. Proteins start folding while they're still being synthesized. The N-terminal end may be properly folded and functional while the C-terminal end is still coming off the ribosome. This means the sequence and the rate of translation both matter. Slow down at certain codons and you can alter the final 3D structure. That's one reason codon usage bias exists — it's not just about speed, it's about giving the protein time to fold correctly as it emerges. Misfolded protein response. When proteins misfold in the ER, the cell triggers the unfolded protein response. This slows down general translation and ramps up chaperone production. If the stress is severe, it can trigger apoptosis. I ran into this issue once while working with a recombinant protein that kept precipitating. We were expressing it at 37 degrees and getting inclusion bodies — clumps of misfolded protein. Switching to a lower expression temperature and using a strain with extra chaperone genes fixed it. The protein itself was fine. The synthesis conditions were the problem.
Subcellular targeting is critical. Proteins destined for the mitochondria, lysosomes, nucleus, or cell surface all have specific signal sequences. A nuclear localization signal, a signal peptide for the ER, a KDEL sequence for ER retention. Miss one of these and the protein ends up in the wrong place and does nothing or causes problems. I've lost count of how many times I've seen someone clone a gene without its targeting sequence and wonder why the protein wasn't where it should be.

Prokaryotes vs Eukaryotes — The Practical Differences
If you're working in a lab setting, knowing the difference between how bacteria and human cells handle protein synthesis will save you time. Bacteria don't have a nucleus, so transcription and translation are coupled. mRNA doesn't need processing like splicing or capping in the same way. It's faster but also less regulated. Eukaryotic protein synthesis is slower, more complex, and subject to many more layers of control. This is also why expressing eukaryotic proteins in bacterial systems sometimes fails. The bacteria won't add the right post-translational modifications. Glycosylation patterns differ. Disulfide bond formation in the bacterial cytoplasm is unreliable because the environment is reducing rather than oxidizing. When I needed proper glycosylation for a project, I switched to insect cells using the baculovirus system. It took longer to set up but the product was actually functional. Ribosome profiling is a technique that maps exactly where ribosomes are sitting on mRNA at any given moment. It's useful for detecting translation pauses, alternative start sites, and non-canonical translation events. If you're doing anything advanced with gene expression, it's worth knowing this exists. Standard RNA-seq tells you how much mRNA is present. Ribosome profiling tells you how much of that mRNA is actually being translated. The two datasets can disagree significantly.
When Protein Synthesis Fails Completely
It's worth being honest about the limitations. Protein synthesis is energy-intensive. A single round of translation consumes GTP at multiple steps — initiation, elongation, and termination all require energy. The cell can't sustain maximum output indefinitely. Nutrient starvation, energy depletion, or stress conditions will shut translation down. This isn't a bug, it's a feature. The cell conserves resources when conditions are bad. Certain toxins specifically target protein synthesis. Ricin removes an adenine from the 28S rRNA in the 60S subunit, permanently disabling it. Diphtheria toxin ADP-ribosylates EF-2, blocking translocation. These are lethal because there's no workaround — once the ribosome is compromised, the cell can't make proteins and dies. Anticoagulants and chemotherapy drugs often work through similar mechanisms, which is why they have side effects. They're not perfectly selective. The main takeaway is that protein synthesis is a regulated, multi-layered process happening across different compartments. Where it happens depends on what the protein is supposed to do. The ribosome is the factory, but the blueprint, the quality control, and the shipping instructions are scattered throughout the cell. Treat it like a system with multiple checkpoints rather than a simple production line and you'll understand why things go wrong when they do.