The Basic Answer
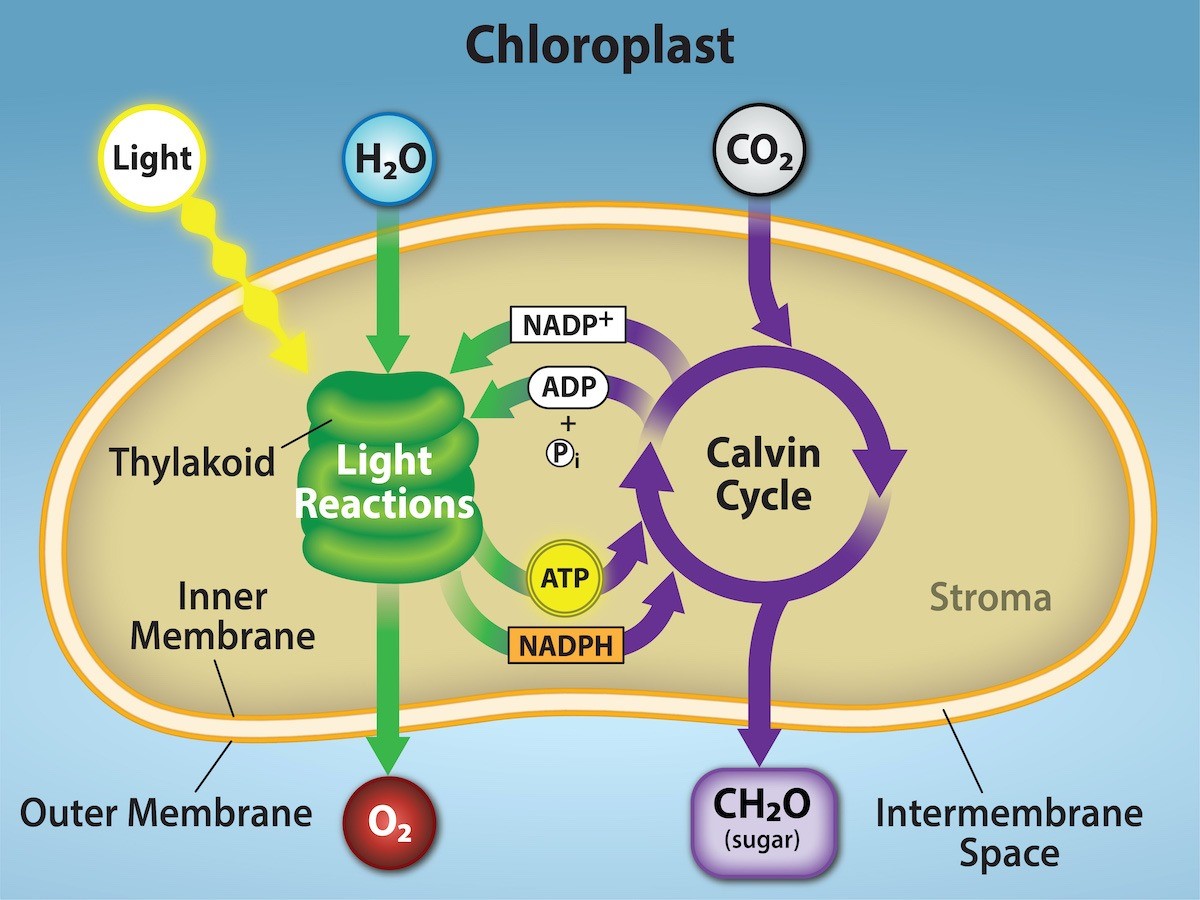
The light-dependent reactions happen in the thylakoid membranes inside chloroplasts. That's it. The thylakoids are those little internal sac structures stacked into grana, and they're where all the photosystems, electron transport chains, and ATP synthase complexes live. Water gets split there, NADPH gets made, and a proton gradient builds up across the membrane. The whole thing runs during daylight hours and feeds the Calvin cycle in the stroma.If you need a quick study answer, that's all most people need. But if you're actually working with this stuff or teaching it, the details get messy fast. It's in the thylakoid membrane, specifically. Not the whole chloroplast. The stroma is where the light-independent reactions happen, so some people conflate the two. They're separate processes in separate compartments, connected by the products that shuttle between them—ATP and NADPH move out of the thylakoid space and into the stroma, while ADP and NADP+ drift back in. The thylakoid membrane itself is protein-dense. It's got photosystem II on one side, photosystem I further down the chain, and the cytochrome b6f complex between them. ATP synthase sits in the membrane too, usually clustered away from the photosystems. This arrangement matters because the spatial organization creates distinct compartments: the lumen inside the thylakoid, which becomes highly acidic during active photosynthesis, and the stroma outside, which stays relatively alkaline.
What Actually Happens There
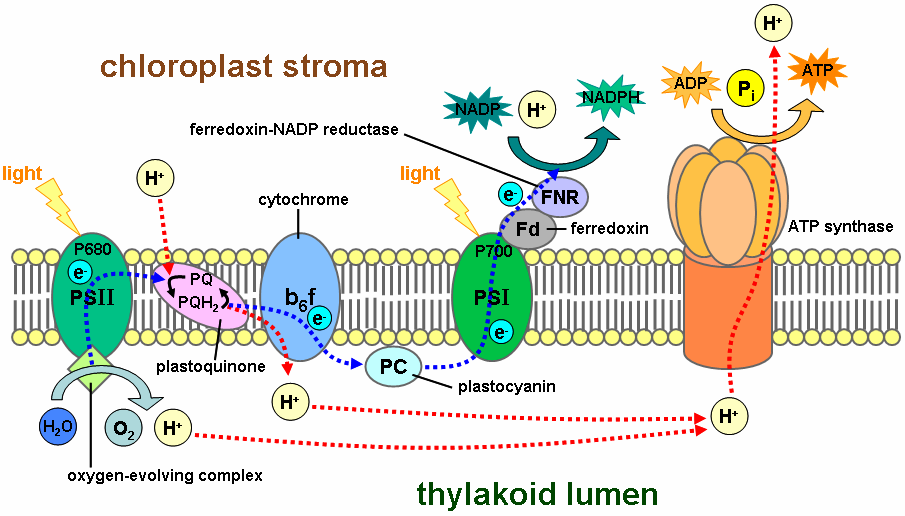
Photons hit PSII first. P680 gets excited, loses an electron, and water gets split to replace it—that's the oxygen-evolving step. The electron moves through plastoquinone, then the cytochrome b6f complex, then plastocyanin, then over to PSI. P700 in PSI gets another photon boost, the electron gets passed to ferredoxin, and finally reduces NADP+ to NADPH. Meanwhile, protons are being pumped into the lumen at cyto b6f, creating that gradient ATP synthase uses. The whole linear electron flow chain takes microseconds from photon absorption to NADPH production. It's efficient, but it's not simple, and that's where people trip up.
Common Mistakes I See All the Time
One big one: people think the light reactions happen in the grana stacks and the Calvin cycle happens in the stroma, so the two are completely separated. They're not. The grana and stroma lamellae are all connected. Electrons and protons move between regions freely. And cyclic electron flow around PSI can happen in the stroma lamellae where PSII isn't present, producing ATP without any NADPH or oxygen evolution. That's a completely separate pathway from the linear flow most textbooks focus on. Another frequent error is assuming the thylakoid lumen stays at a constant pH. It doesn't. During peak light, the lumen can drop to pH 4.5 or lower while the stroma sits around pH 8. That's a ten-thousand-fold difference in proton concentration across a membrane maybe 5 nanometers thick. The plant uses this gradient for both ATP synthesis and photoprotection through non-photochemical quenching.
Get the Full Details

A Real Problem I Encountered
I was calibrating a pulse-amplitude modulation (PAM) fluorometer for a physiology lab once, trying to measure maximum quantum yield (Fv/Fm) in shade-adapted leaves. The values came out weird—sometimes above 0.85, which is basically impossible for healthy plants. Turned out the leaves had been stored in near-darkness for about twelve hours before testing, and the dark adaptation period we were using—thirty minutes—wasn't enough to fully relax the xanthophyll cycle. The qE component of NPQ was still partially active, inflating the variable fluorescence reading. The fix was straightforward once we figured it out: extend the dark adaptation to at least two hours, or better yet, measure the leaves directly on the plant in the field with the clamp-on probe after a fifteen-minute shading period. Field measurements avoided the whole storage problem. It was a minor logistical headache but it cost us about a day of wasted data before we caught it.
Counter-Intuitive Things Nobody Tells You
First, the light-dependent reactions don't actually require light all the time in a continuous sense. They can run in brief flashes. A single saturating flash can drive the entire electron transport chain through one complete turn. The intermediates then sit in reduced or oxidized states until the next photon arrives. This is why flash photolysis experiments work and why plants can do photochemistry even at very low light intensities—the system doesn't need constant illumination, it needs individual photons. Second, plants under high light don't just ramp up the light reactions indefinitely. They actively down-regulate them. State transitions, where LHCII phosphorylation shifts antenna complexes between PSII and PSI, is one mechanism. But more importantly, excess light energy gets safely dissipated as heat through the xanthophyll cycle—violaxanthin converting to zeaxanthin via antheraxanthin. This isn't a backup system. It's the primary mode of operation at midday in full sun. The light reactions are routinely running well below maximum capacity because the plant is deliberately holding back.
When This Whole System Breaks Down
It breaks under stress. Drought closes stomata, CO2 drops, the Calvin cycle slows, and the light reactions keep getting excited electrons with nowhere productive to send them. You get singlet oxygen formation at PSII, lipid peroxidation in the thylakoid membrane, and photoinhibition. The plant repairs D1 protein in PSII continuously under normal conditions, but under stress the damage rate exceeds the repair rate and photosynthetic capacity collapses. There's no workaround for this except giving the plant what it needs—water, appropriate light levels, functional stomata. Nothing you do externally fixes damaged thylakoid membranes. The best you can do is prevent the damage in the first place.
Bottom Line
The light-dependent reactions occur in the thylakoid membranes of chloroplasts. They convert light energy into chemical energy in the form of ATP and NADPH, using water as an electron source and releasing oxygen as a byproduct. The spatial organization of the membrane, the proton gradient across it, and the regulatory mechanisms that prevent damage are all part of what makes this work. If you're studying for a basic exam, the thylakoid membrane is your answer. If you're doing actual research or working with living plants, pay attention to the regulation and the edge cases, because that's where things get interesting.