Understanding What Actually Comes Out of the Citric Acid Cycle
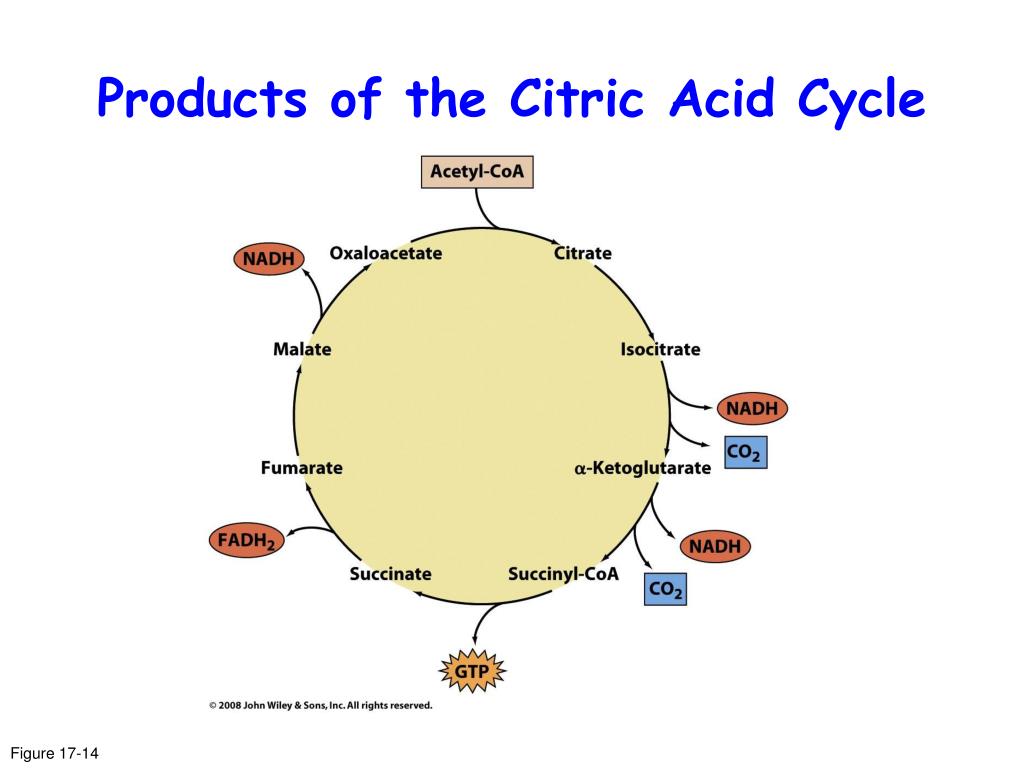
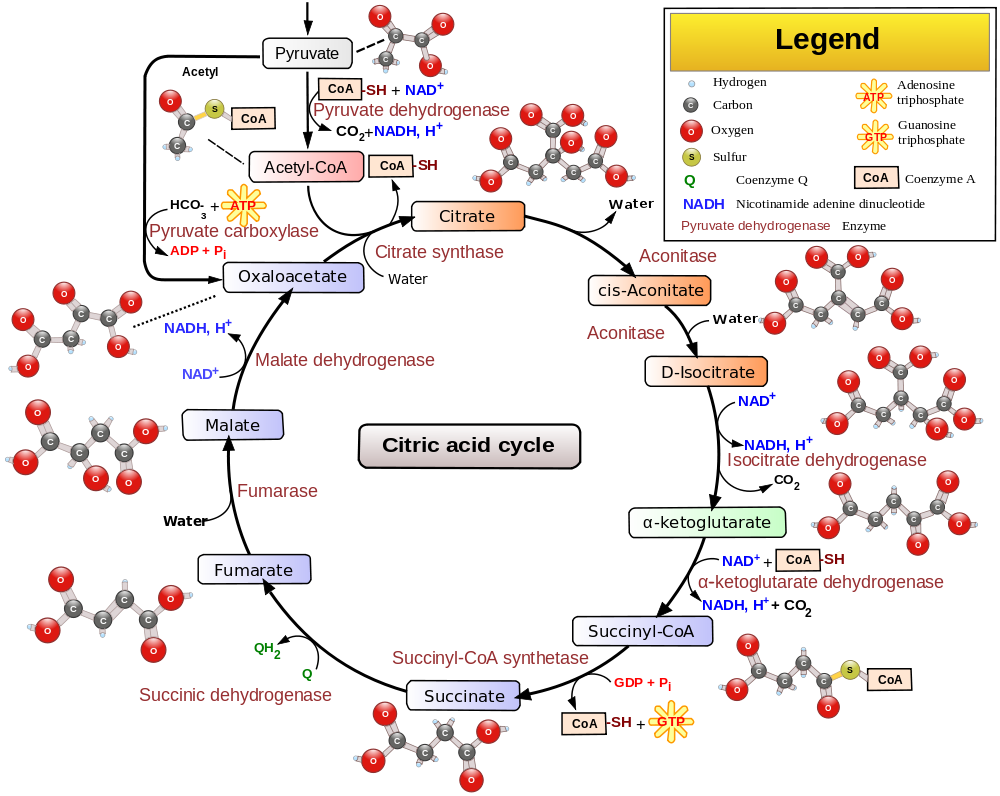
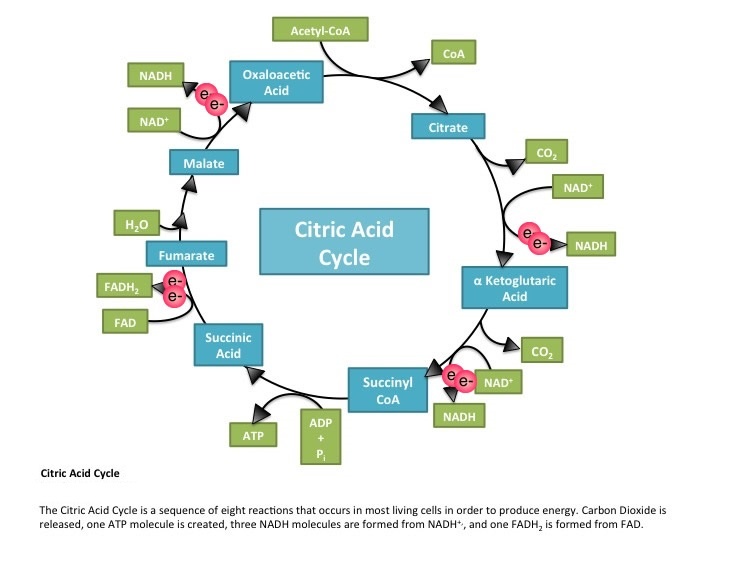
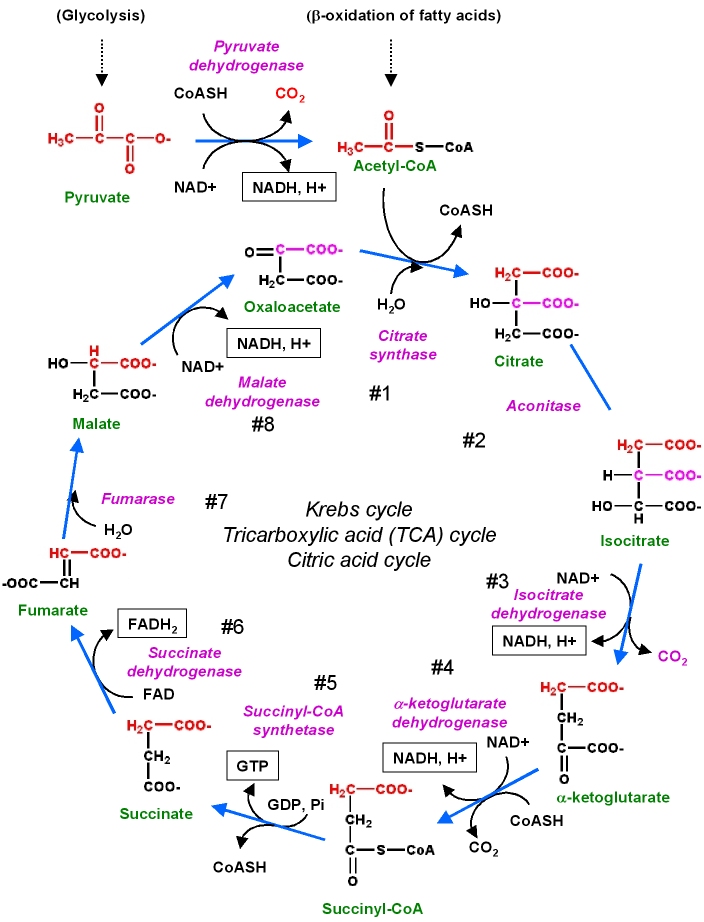
The citric acid cycle runs inside the mitochondrial matrix, and every turn of it takes one molecule of acetyl-CoA and produces a very specific set of outputs. People tend to memorize a list and move on, but if you're trying to actually understand metabolism — whether that's for a course, research, or clinical work — knowing exactly what comes out and why it matters is where things get useful. Per one acetyl-CoA entering the cycle, the direct products are: 3 NADH — These carry high-energy electrons to the electron transport chain. That's the main point of the cycle for most cells.
1 FADH2 — Also feeds electrons into the chain, but enters at Complex II, so it yields less ATP than NADH during oxidative phosphorylation. 1 GTP (or ATP) — Generated by substrate-level phosphorylation at the succinyl-CoA synthetase step. In many cell types this comes out as GTP, which is then converted to ATP by nucleoside diphosphate kinase. Some textbooks just write ATP directly; both are correct depending on the organism or tissue. 2 CO2 — These are the waste products from the two decarboxylation steps (isocitrate dehydrogenase and alpha-ketoglutarate dehydrogenase). They don't carry energy out of the cycle; they're just carbon leaving the system.
1 regeneration of oxaloacetate — Not a net product, but essential. The cycle has to close or it stops. If oxaloacetate gets pulled away for gluconeogenesis, the whole thing slows down. This is called anaplerosis when other pathways refill it. That's per acetyl-CoA. Since one glucose produces two pyruvates and therefore two acetyl-CoAs, you double those numbers for a full glucose oxidation through the cycle alone: 6 NADH, 2 FADH2, 2 GTP/ATP, 4 CO2. I ran into a real problem once when a student was calculating the total ATP yield from one glucose molecule and kept getting inconsistent numbers. The issue wasn't the math — it was that different textbooks use different P/O ratios. Some say each NADH gives 2.5 ATP and each FADH2 gives 1.5. Others still use the older values of 3 and 2. The discrepancy comes from how proton leakage and the cost of transporting ADP and Pi into the mitochondrion are counted. If you're doing yield calculations for a class, check which convention your professor uses. If you're doing it for research, report which P/O ratio you assumed and don't pretend the number is more precise than it is.
Get the Full Details
Here's something beginners often miss: the citric acid cycle is not just an energy-harvesting machine. It's a metabolic hub. Several intermediates are siphoned off for biosynthesis. Citrate leaves the mitochondrion for fatty acid synthesis. Alpha-ketoglutarate is a nitrogen sink for amino acid production via transamination. Succinyl-CoA feeds into heme synthesis. Oxaloacetate becomes phosphoenolpyruvate for gluconeogenesis. When a cell is growing and needs to build membranes and proteins, it pulls these intermediates out, and the cycle can't run at full speed unless those gaps are refilled. That's why anaplerotic reactions like pyruvate carboxylase converting pyruvate to oxaloacetate aren't optional side quests — they're necessary maintenance. Another thing that doesn't get enough emphasis: the cycle requires a minimum threshold of oxaloacetate to function. You can have plenty of acetyl-CoA and all the enzymes in the world, but if oxaloacetate is low, acetyl-CoA builds up and gets shunted toward ketone body production instead. This is exactly what happens during prolonged fasting or uncontrolled diabetes. The cycle doesn't break — it essentially goes idle because the entry point is starved. Ketogenesis isn't some separate alternate pathway; it's what happens when the citric acid cycle can't accept the acetyl-CoA coming at it. The cycle also doesn't operate in isolation from the rest of the cell's redox state. High NADH/NAD+ ratios inhibit three key enzymes: isocitrate dehydrogenase, alpha-ketoglutarate dehydrogenase, and malate dehydrogenase. So even if substrates are present, a backed-up electron transport chain — say from hypoxia or cyanide poisoning — will slow the cycle to a crawl simply because there's nowhere for those electrons to go. The cycle is Aerobically gated in a way that people don't always appreciate.
If you're studying this for an exam, focus on the enzyme steps that are truly regulatory: citrate synthase, isocitrate dehydrogenase, and alpha-ketoglutarate dehydrogenase. Those are the three committed control points. Succinate dehydrogenase matters too but mostly because it's embedded in the inner membrane and directly connected to the electron transport chain. The other steps are near-equilibrium reactions that just ride the concentration gradients. One more practical note: the NADH produced in the mitochondrial matrix can't cross the inner membrane. Cells use shuttle systems to get those electrons into the transport chain — the malate-aspartate shuttle in heart and liver tissue, the glycerol-3-phosphate shuttle in brain and skeletal muscle. These shuttles have different efficiencies, which is why the same amount of glucose can yield slightly different ATP totals depending on which tissue you're looking at. If someone tells you the number is exactly 30 or 32 ATP per glucose, they're simplifying. The real answer depends on the shuttle, the P/O ratio, and how leaky your membranes are. The citric acid cycle itself is elegant in its simplicity, but treating it as just a circular list of products does it a disservice. It's a dynamic interface between catabolism and anabolism, and it responds constantly to the cell's actual needs rather than some idealized textbook condition.