Understanding Active Transport in Cellular Biology
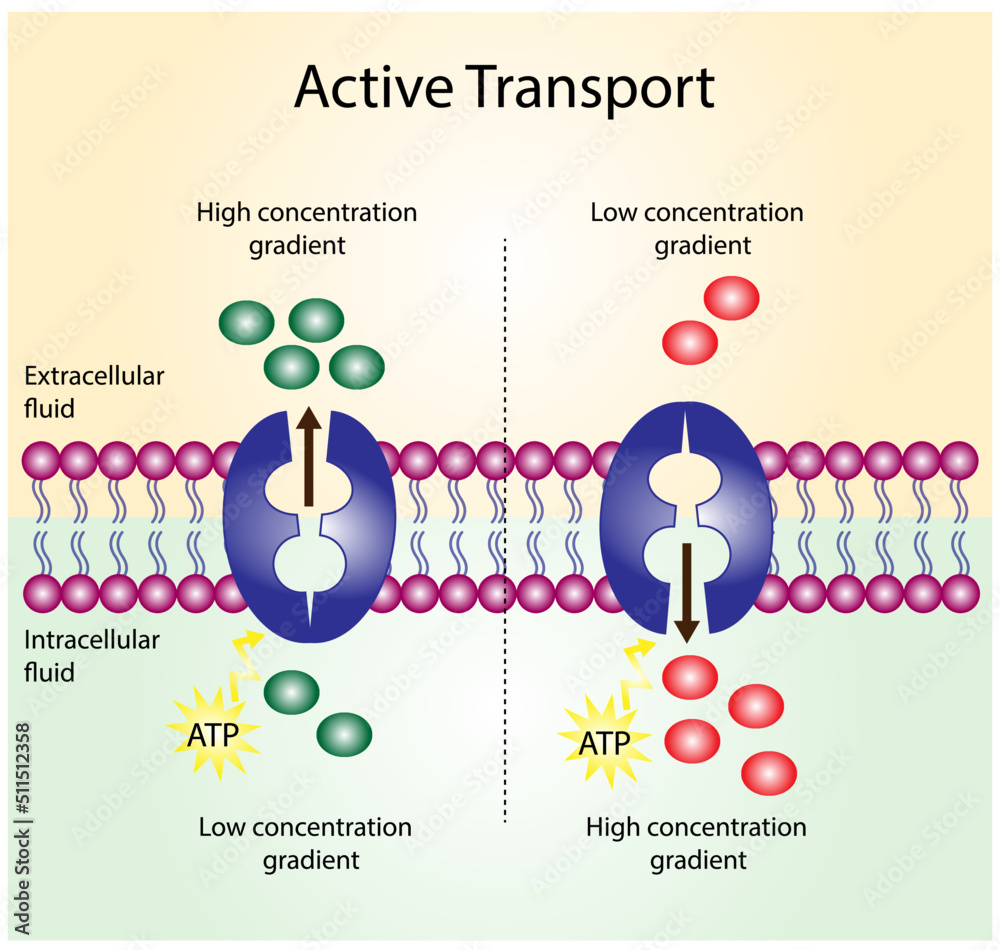
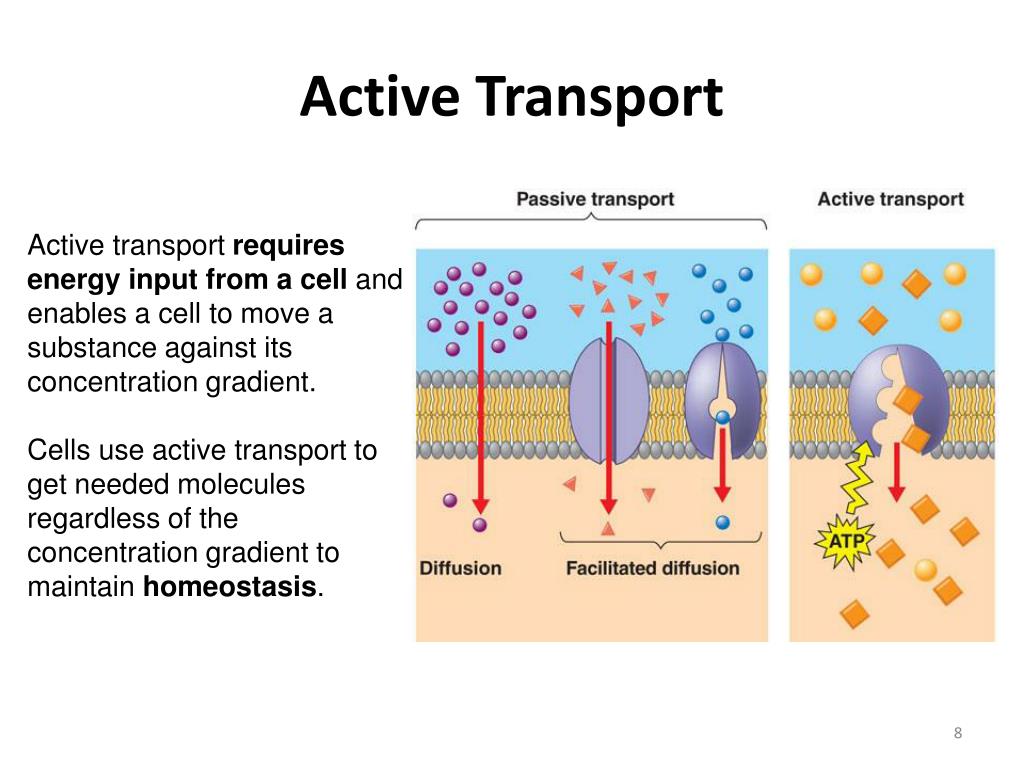
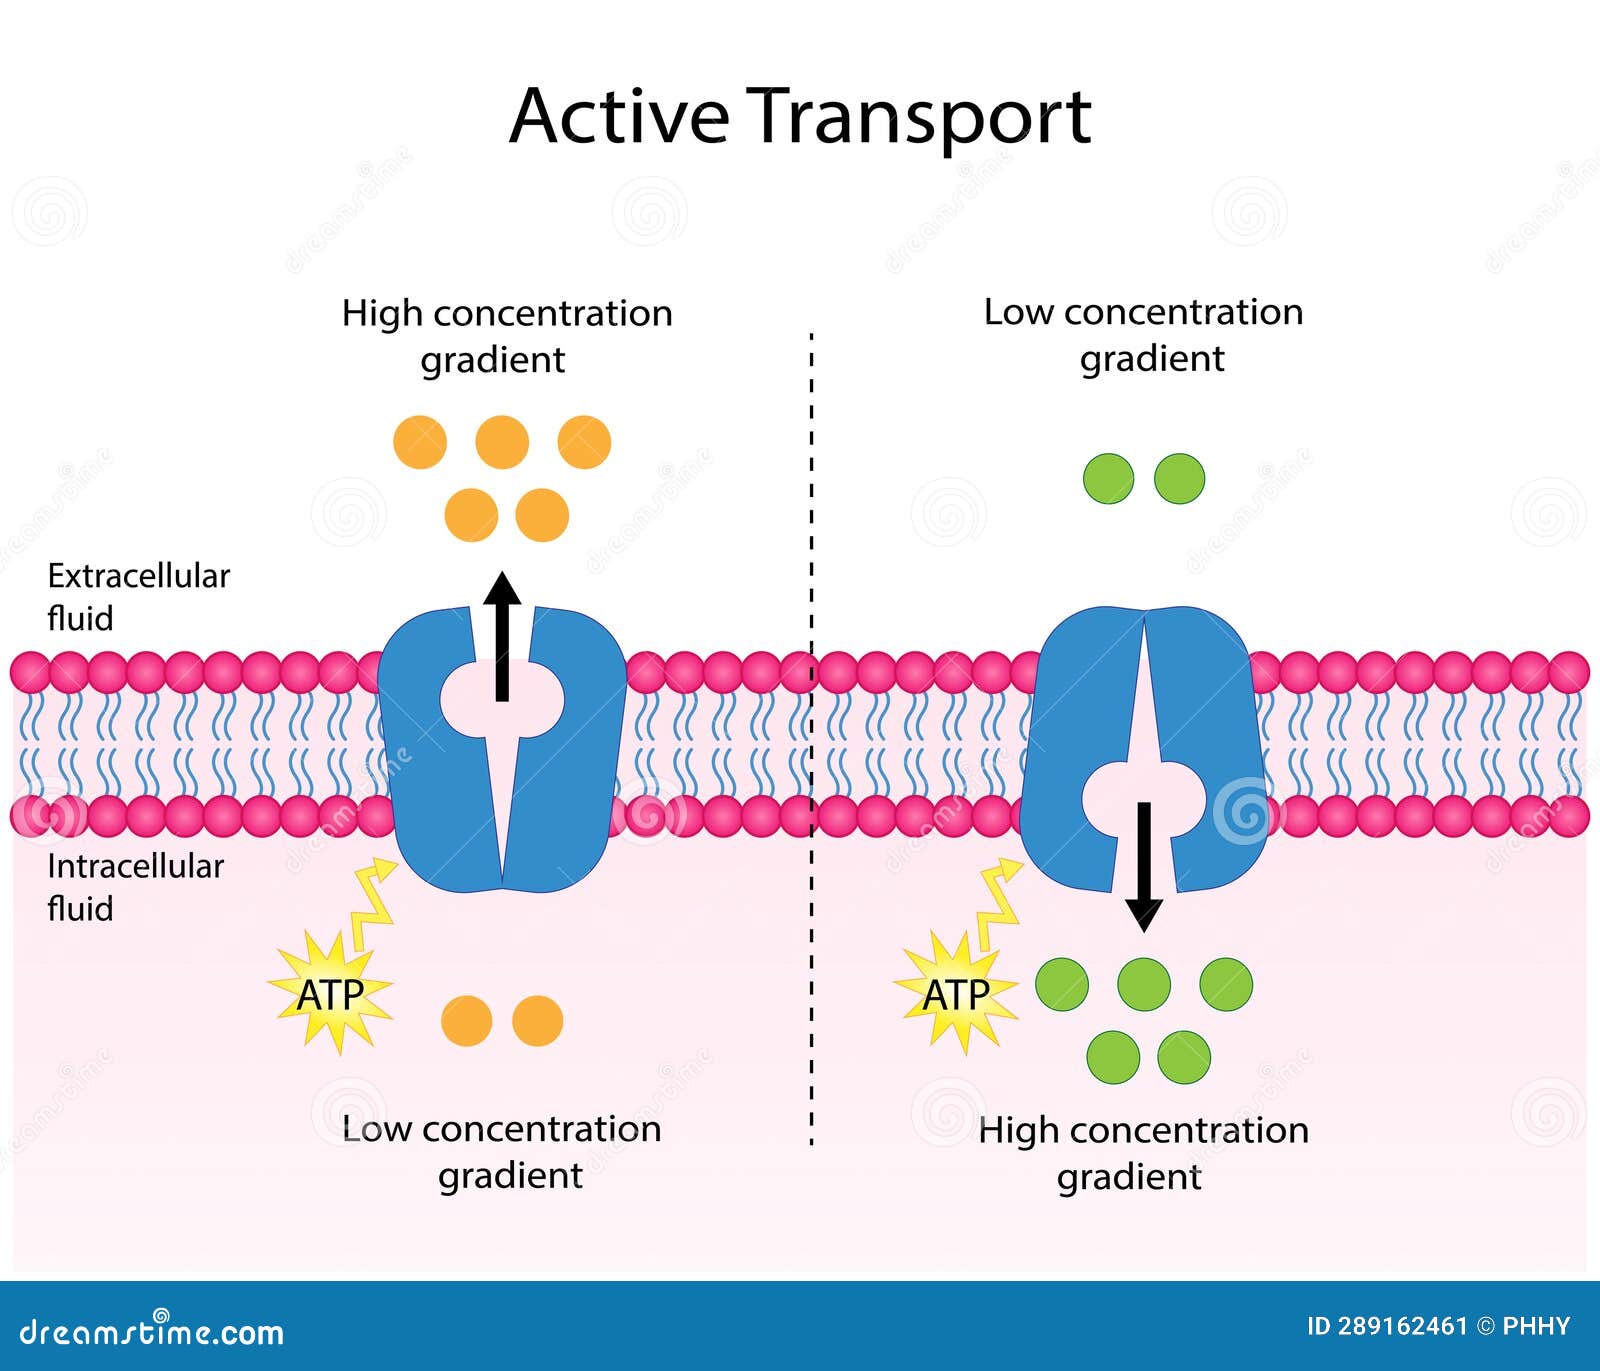
Active transport is one of those topics that gets glossed over in intro biology classes but actually comes up way more than you'd expect when you're dealing with real lab work or teaching advanced students. The short answer is yes, active transport requires energy. But the longer answer is where things get interesting, and where most people mess it up. At the cellular level, active transport moves molecules against their concentration gradient—from low concentration to high concentration. This doesn't happen spontaneously. You need input. In biological systems, that input usually comes from ATP hydrolysis, but it can also come from electrochemical gradients established by other active transport processes. The sodium-potassium pump is the classic example everyone learns about. It pumps three sodium ions out of the cell and two potassium ions in, using one ATP molecule per cycle. This creates and maintains the membrane potential that nerve cells depend on. If you block ATP production with something like cyanide, the pump stops within seconds and the cell loses its ability to fire action potentials. That's not theoretical— I've seen undergrad labs demonstrate this exact thing with isolated nerve tissue and a simple conductivity meter. The signal dies almost immediately once you add the metabolic inhibitor.
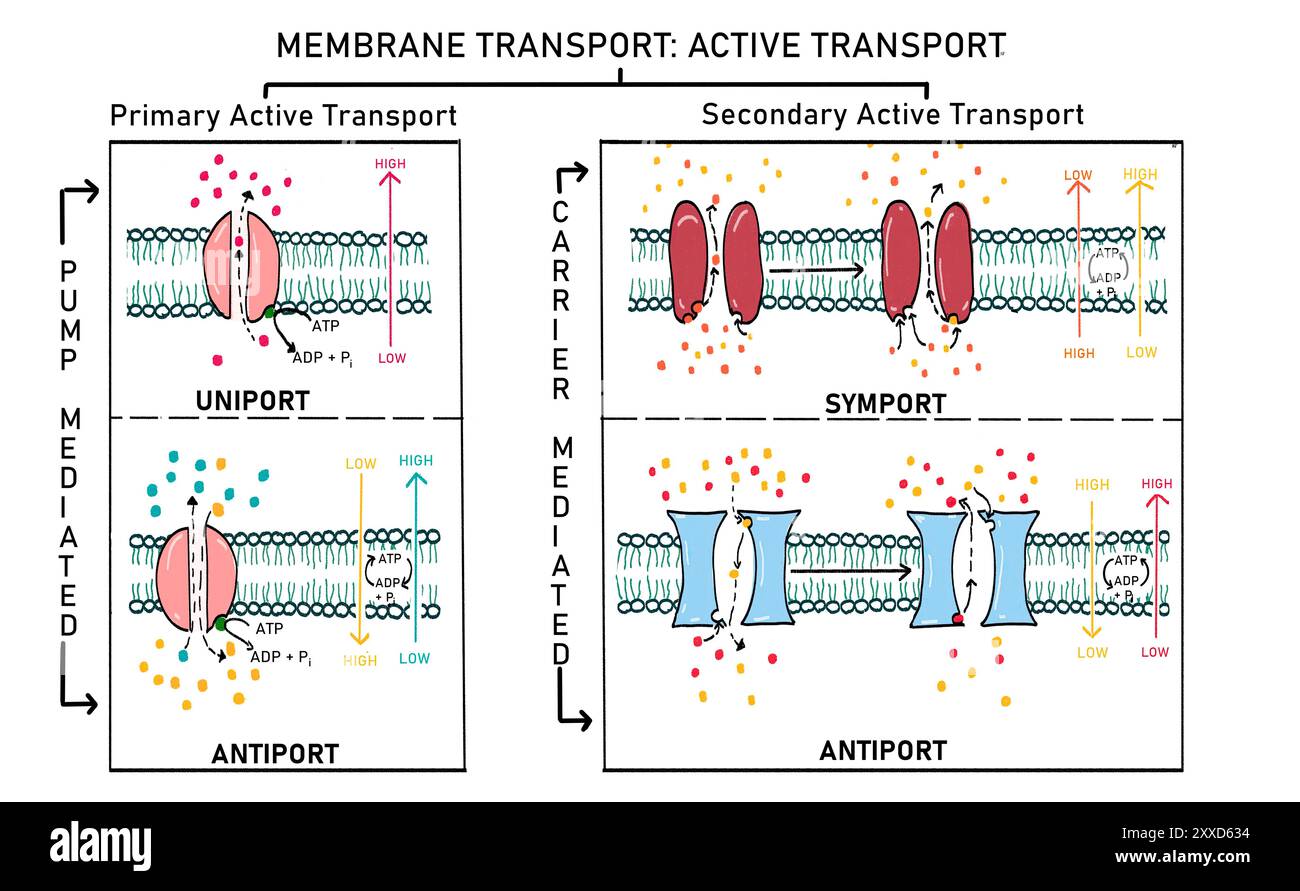
But here's what textbooks don't always make clear: not all active transport uses ATP directly. Secondary active transport, also called coupled transport, piggybacks on gradients that were established by primary active transport. The sodium-glucose cotransporter in your intestinal epithelium is a perfect example. It doesn't touch ATP itself. Instead, it uses the sodium gradient that the Na+/K+ pump created earlier. So technically, energy is still required—it's just indirect. This distinction matters more than you'd think when you're designing experiments or interpreting pharmacological data. I ran into this nuance directly when I was troubleshooting an unexpected result in a transport assay back when I was running a teaching lab. We were measuring glucose uptake in cultured epithelial cells, and the numbers didn't match published values at all. Turns out the cell line had downregulated its Na+/K+ ATPase expression after too many passages. The secondary active transport was starving because the primary pump that fed it had given out. We caught it because we also measured sodium gradients directly, which most protocols skip. If we'd only looked at glucose uptake without that context, we would have wasted weeks chasing a reagent problem that didn't exist.
When Active Transport Fails or Gets Overlooked
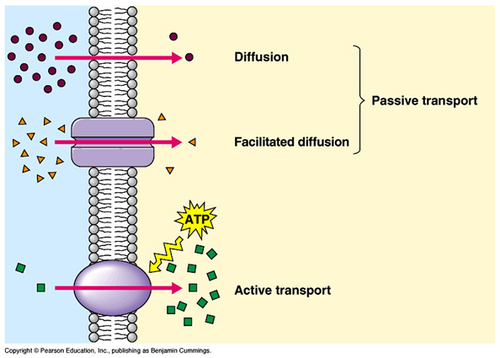
There are scenarios where the energy requirement becomes a critical bottleneck. Drug delivery is one area where this shows up repeatedly. Many pharmaceutical compounds rely on active transport mechanisms to cross cell membranes, and if a patient has compromised ATP production—say, from mitochondrial disease or certain toxins—the drugs won't reach effective intracellular concentrations. I've seen case reports where standard dosing produced therapeutic failure simply because the patient's cells couldn't power the transporters anymore. Another practical issue is that active transport has a maximum velocity. Unlike passive diffusion, which speeds up linearly with concentration gradient, active transport saturates. The proteins do the work, and there's a finite number of them in the membrane. Once you hit Vmax, adding more substrate does nothing. This is why competitive inhibitors can be so effective therapeutically—they're not blocking the energy source, they're blocking the carrier proteins themselves. The energy is still being spent, but nothing useful gets transported. Ion channels are often confused with active transport because they move ions across membranes, but they're fundamentally different. Channels are passive. They open and ions flow down their gradient. No ATP required. The confusion runs deep in introductory courses, and it causes problems when students try to reason through more complex physiology later on. A good rule of thumb: if it moves against a gradient, it costs energy. If it moves with one, it doesn't. But even that gets fuzzy with things like ion-coupled transporters that move one ion downhill to push another uphill, which blurs the line between passive and active in ways that tripped up half my students in a single semester.
Get the Full Details
Practical Considerations for Lab Work
If you're working with active transport in an experimental context, temperature control matters more than people realize. Most transport proteins have Q10 values in the 2-3 range, meaning their rate doubles or triples for every ten-degree increase. Running assays at room temperature instead of 37°C can make your transport rates look artificially low, and if you're comparing across papers, make sure the temperatures match. I've lost count of how many times someone asked me whether a discrepancy in their data was biological or just thermal. Membrane potential also plays a role that gets ignored too often. The electrochemical gradient isn't just about concentration—it's about charge too. For charged solutes, the membrane potential can either assist or oppose transport depending on the ion's sign and the inside-outside voltage. If you're studying cation transport and your cells are hyperpolarized, the electrical force is pulling those cations in, which means your apparent transport rate might reflect both chemical and electrical driving forces working together. Decoupling those requires voltage-clamp techniques that aren't always available in teaching or even mid-level research labs. The bottom line is that active transport absolutely requires energy, but the details of how that energy gets delivered and where the process breaks down are where real understanding lives. The ATP-dependent pumps get all the textbook space, but secondary transport, saturation kinetics, and the interplay between chemical and electrical gradients are what actually determine how these systems behave in living organisms.