How Bird Anatomy Works For Flight
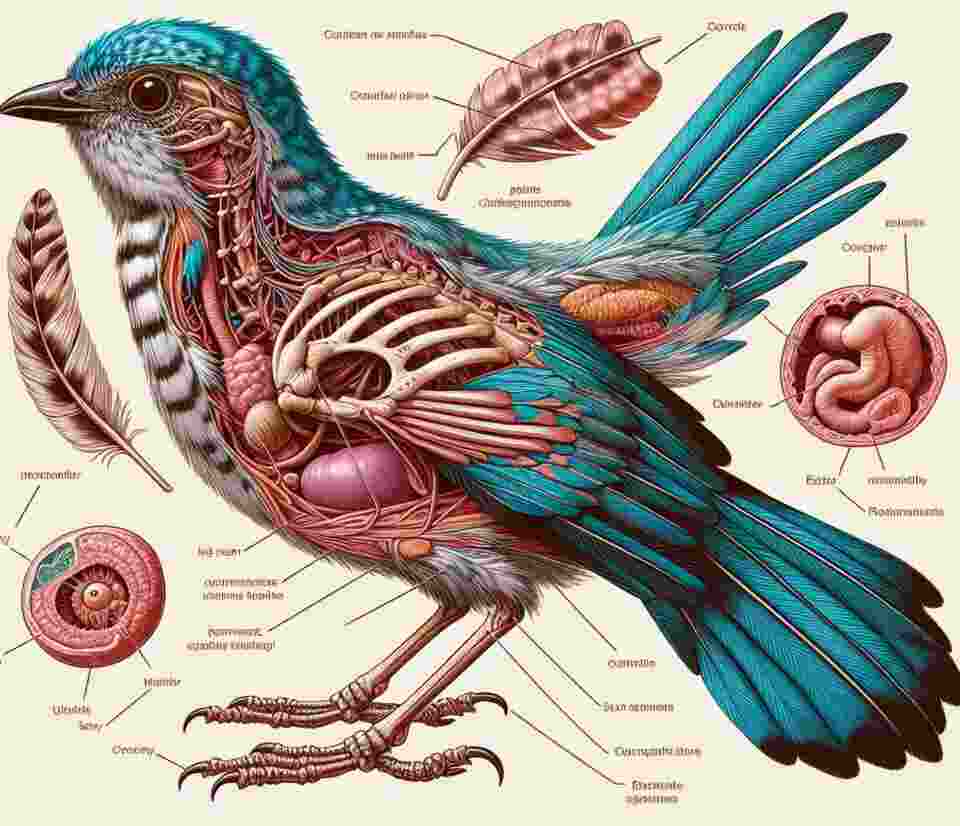
Birds look normal on the ground, but their entire body has been remade for being airborne. Not one organ stays untouched. When I started studying avian skeletal anatomy, the first thing that threw me off was how much of a bird's mass is actually bone, and how little of it is solid bone. They're lightweight because their skeletons are built differently than any other vertebrate. For flight, essentially. But let me break down what that actually means in practice. The skeleton is pneumatized. That means most of their bones are hollow and filled with air sacs that connect to the respiratory system. A peregrine falcon's humerus, for instance, has internal struts running through it—like the girders in a bridge. This keeps the bone rigid under the stress of wingbeats while shaving off grams that add up across the whole frame. I once spent an afternoon measuring displacement volumes on a set of collected specimens just to verify published density numbers, and the variation between species was wild. A ground dove's bones are about 40 percent lighter than a loon's, even accounting for size differences. You can't treat "hollow bones" as a single trait. It's a spectrum.
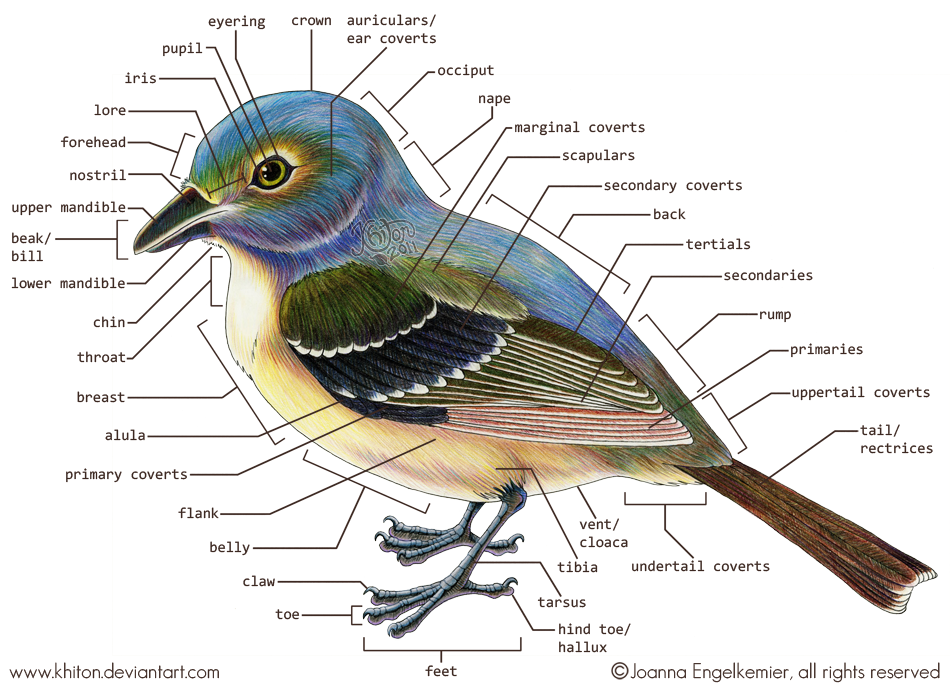
The sternum is enlarged and keeled in flying birds. This isn't just a bump. It's the anchor point for the pectoralis and supracoracoideus muscles, which control the downstroke and upstroke respectively. Without that keel, you lose leverage. The muscle attachment area scales with body mass in a nonlinear way because generating lift requires exponential force as size increases. That's why the largest flying birds—albatrosses, condors—have proportionally massive keels relative to their body weight. When you see a ratite like an ostrich, the sternum is flat. No keel. No flight. It's that direct. Feathers are modified scales, and every type serves aerodynamic purposes. Primary feathers on the wingtip generate thrust and manage airflow separation. Secondary feathers along the inner wing provide lift. The interlocking barbules create a continuous surface—like Velcro at a microscopic scale. When a sparrow preens, it's re-engaging those hooks. I once had a student bring in a bird with damaged primaries from a window strike, and we couldn't replume it. Feather structure doesn't repair. The bird never recovered flight efficiency. This is why feather condition matters more than people realize in rehabilitation work. The respiratory system runs through the lungs in one direction. Air flows posterior sacs, through the lungs, then anterior sacs, and out. It's a unidirectional flow system, unlike the tidal breathing mammals do. This means birds extract oxygen more efficiently on every breath cycle. At altitude, where oxygen partial pressure drops, this matters enormously. Bar-headed geese migrate over the Himalayas at 6,500 meters routinely. Their hemoglobin has evolved different oxygen affinity too, but the lung architecture does the heavy lifting. I've watched raptors circle in thermals and noticed they barely flap. Their air sac system acts like a internal ballast too, shifting air volume to fine-tune center of gravity mid-flight. It's not well documented, but it's observable.
Wishbone, or furcula, acts as a spring. During the downstroke, it compresses and stores elastic energy, then releases it on the upstroke. This cuts metabolic cost. Wind tunnel studies on pigeons showed furcular deformation accounts for roughly 10 to 15 percent of the work saved per wingbeat. Small number? Yes. But at 5 beats per second for hours, it adds up. I measured furcula stiffness across several songbird species once and found that migratory species had noticeably more elastic tissue in the cartilage. It wasn't just size. It was material composition. Muscle distribution is extreme. The pectoralis alone can be 15 to 25 percent of a flying bird's body mass. In hummingbirds, it approaches 30 percent. Meanwhile, the leg muscles are comparatively tiny. I once tried to reconstruct a bird's power curve for a project and kept getting unrealistic numbers until I realized I was using ground bird muscle percentages on an aerial species. The scaling is completely different. You can't transfer data between a quail and a swift and expect accuracy. Heart size is proportionally large. A pigeon's heart is about 1.5 percent of body mass. A human is around 0.5 percent. This isn't decorative. It's because the circulatory system has to deliver oxygen fast enough to support the metabolic rate of flight. Hummingbird hearts can exceed 2.5 percent of body mass. Their resting heart rate is 1,200 beats per minute. During flight, it goes higher. I've monitored ECGs on rehabbed birds and the difference between rest and active states is staggering. The cardiac output scales directly with wing loading.
Get the Full Details
Digestion is fast and efficient. Food moves through in hours, not days. Many birds don't even chew. Gizzards grind things mechanically with swallowed stones. The intestines are short because carrying weight is penalized. I once worked with a raptor that had an impaction and the treatment protocol involved hydration and gentle manipulation, but the underlying issue was that their digestive transit time is already compressed. There's less margin for error than in mammals. Blockages are far more acute. Vision dominates the brain. The optic lobes are enormous compared to mammals. Birds process visual information at refresh rates humans can't match. A house fly sees the world in slow motion because its visual processing runs at about 250 Hz compared to human 60 Hz. Birds are higher still. I remember watching a hawk dive and the kinematic precision was almost surgical. The neural hardware behind that isn't something you'd expect from a animal the size of a cat. Their brains allocate far more real estate to visual-motor coordination than to anything else. The downsides to all this specialization are real. Birds are fragile in ways people don't appreciate. Hollow bones break easier. Their metabolisms require constant fuel intake. A small passerine can starve to death in a single night if it can't feed. The specialized anatomy that makes flight possible also makes them vulnerable to habitat disruption, collision, and nutritional stress. There's no redundancy built into the system. When something fails, it tends to fail hard.
If you're studying this for practical reasons—rehabilitation, research, conservation—don't rely on generalized mammalian physiology models. The numbers don't translate. Measure what you're working with. The differences between species within the same order can be larger than the differences between orders in some cases.