Understanding Energy Flow in Ecosystems
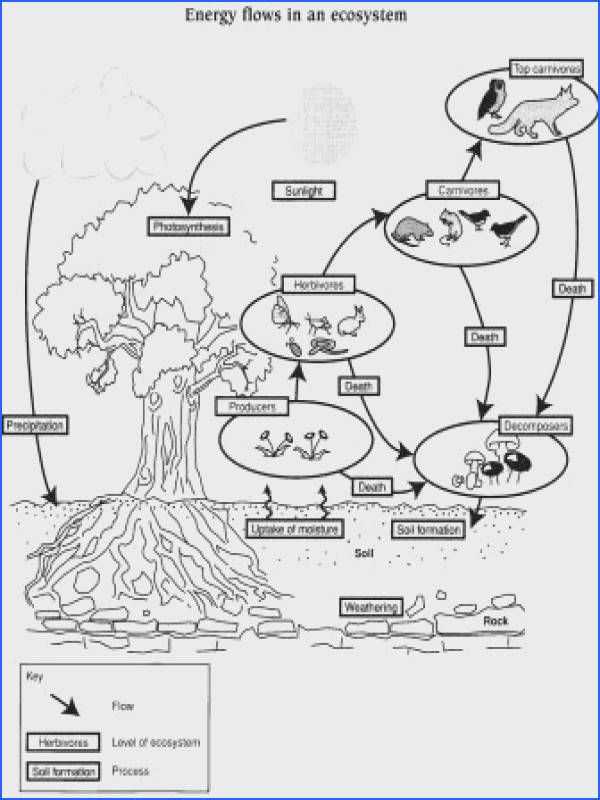
I spent a lot of time going through student papers on trophic dynamics, and the answers were almost always shallow. Students memorized the pyramid shape and stopped there. What actually matters is understanding how energy moves through a system, where it gets lost, and why the losses are non-negotiable. This guide covers the core concepts you need, not just the textbook definitions. Energy enters ecosystems as sunlight. Producers capture it through photosynthesis, converting roughly 1 to 2 percent of incoming solar radiation into chemical energy stored in biomass. That is the bottleneck most people gloss over. The rest of the solar energy is reflected, passes through the plant without being absorbed, or gets used in processes that do not store chemical energy at all. When a primary consumer eats a plant, it does not get all the energy the plant stored. A significant chunk is lost as heat during respiration, another portion goes into waste, and some energy remains in the plant material that the consumer could not digest. The standard figure you will see everywhere is the 10 percent rule. Only about 10 percent of the energy at one trophic level transfers to the next level. The remaining 90 percent is dissipated as metabolic heat or excreted.
Flow In Ecosystems Answer Key
Below is a compact set of the key facts you need. If you are looking at an answer key for a class assignment, these points cover the vast majority of what gets asked. Here is something that tends to trip people up on exams. The 10 percent rule is a rough average, not a fixed constant. In some aquatic systems, the transfer efficiency between phytoplankton and zooplankton can reach 20 percent because phytoplankton have high nutritional quality and are fully digestible. In contrast, energy transfer from grass to a grazing herbivore might be closer to 5 percent because cellulose is difficult to break down. The rule holds as a teaching tool. It fails when you apply it to specific calculations without checking the actual efficiency for that system. I ran into this exact problem when grading a set of calculations where a student applied 10 percent uniformly across every trophic step in a detrital food web. The numbers came out wrong because detritivores and decomposers operate under different efficiency constraints than the grazing chain. The correct approach is to treat detrital pathways separately and use actual measured efficiencies when data is available, rather than forcing the 10 percent assumption onto every step.
If you need to calculate energy available at a given trophic level, start with the gross primary production value and work downward. Subtract respiration to get net primary production. Then apply the transfer efficiency for each step. For a typical three-level system, you might calculate it like this: gross primary production of 10,000 kilocalories per square meter per year. Net primary production comes to about 5,000 after respiration losses. Primary consumers receive roughly 500. Secondary consumers receive about 50. The numbers get small fast, and that is the point. Another concept that does not get enough attention is the difference between standing crop and energy flow. Standing crop measures biomass at a single point in time. Energy flow measures the rate at which energy moves through the system. In a temperate forest, the standing crop of producers is large, but the turnover rate is slow. In a phytoplankton community, the standing crop is tiny, but the turnover rate is extremely fast. Both systems can support similar consumer populations despite having very different standing crops. Exam questions sometimes try to confuse these two measures, so keep them separate in your head. The Liebig factor and energy limitation are related but distinct ideas. Energy limits how much biomass a system can support at higher trophic levels. Nutrient availability limits primary production itself. In oceanic systems, nitrogen or iron often limits phytoplankton growth. In terrestrial systems, phosphorus can be the constraint. When you see a question about what controls ecosystem productivity, identify whether the context is about energy input or nutrient supply.
Get the Full Details

Human impacts on energy flow are usually framed in terms of habitat destruction, but the more direct effect is the simplification of food webs. Removing top predators causes trophic cascades. Remove the predator and the herbivore population increases, which increases grazing pressure on producers, which reduces plant biomass. This changes the energy distribution across the entire system. The direction of the cascade depends on whether the system is primarily driven by bottom-up resource control or top-down predator control, and that is another detail students tend to mix up. If you are using an answer key to check your work, look for these common errors. Confusing GPP with NPP is the most frequent. Students will often use gross production as the starting point for consumer energy calculations when they should be using net production. Another mistake is reversing the relationship between trophic level and biomass. Some students think more energy at the top means more biomass at the top, which contradicts the basic structure of energy pyramids. The pyramid shape exists specifically because energy decreases at each level. A practical tip that actually helps with these assignments. When you see a question asking about energy loss between trophic levels, think about the three fates of consumed energy. It is either assimilated, egested as waste, or respired as heat. Assimilated energy is split between growth and reproduction versus respiration. The portion that goes to growth is what becomes available to the next trophic level. If you track energy this way, most calculation problems become straightforward arithmetic instead of guesswork.
The deeper issue with how these topics are taught is that the numbers feel abstract. They are not. The reason food chains rarely exceed five trophic levels is not arbitrary. It is because the energy remaining at the fifth level is insufficient to maintain a viable breeding population. You will see this play out in real ecosystems. Apex predators are always rare relative to the organisms they depend on. That rarity is a direct consequence of energy loss at each transfer. Any answer key question about why there are fewer eagles than there are grasshoppers is really asking about the cumulative effect of thermodynamic inefficiency. For students who want to go beyond the standard curriculum, look into ecological efficiency models developed by Lindeman in 1942. His work established the foundation for modern energy flow analysis. More recent research uses stable isotope analysis to trace actual energy paths instead of relying on theoretical transfer rates. The isotope data sometimes shows transfer efficiencies that differ significantly from the 10 percent benchmark, which reinforces why you should not treat that number as a universal law. If you are compiling your own study materials or need a reference document for review, the essential structure is the same every time. Sunlight enters. Producers convert it. Consumers eat producers or other consumers. Decomposers process waste and dead matter. Heat leaves the system at every step. Energy does not recycle. Nutrients do. Keep those two tracks separate and you will rarely go wrong.