Mapping Tropical Rainforest Trophic Networks
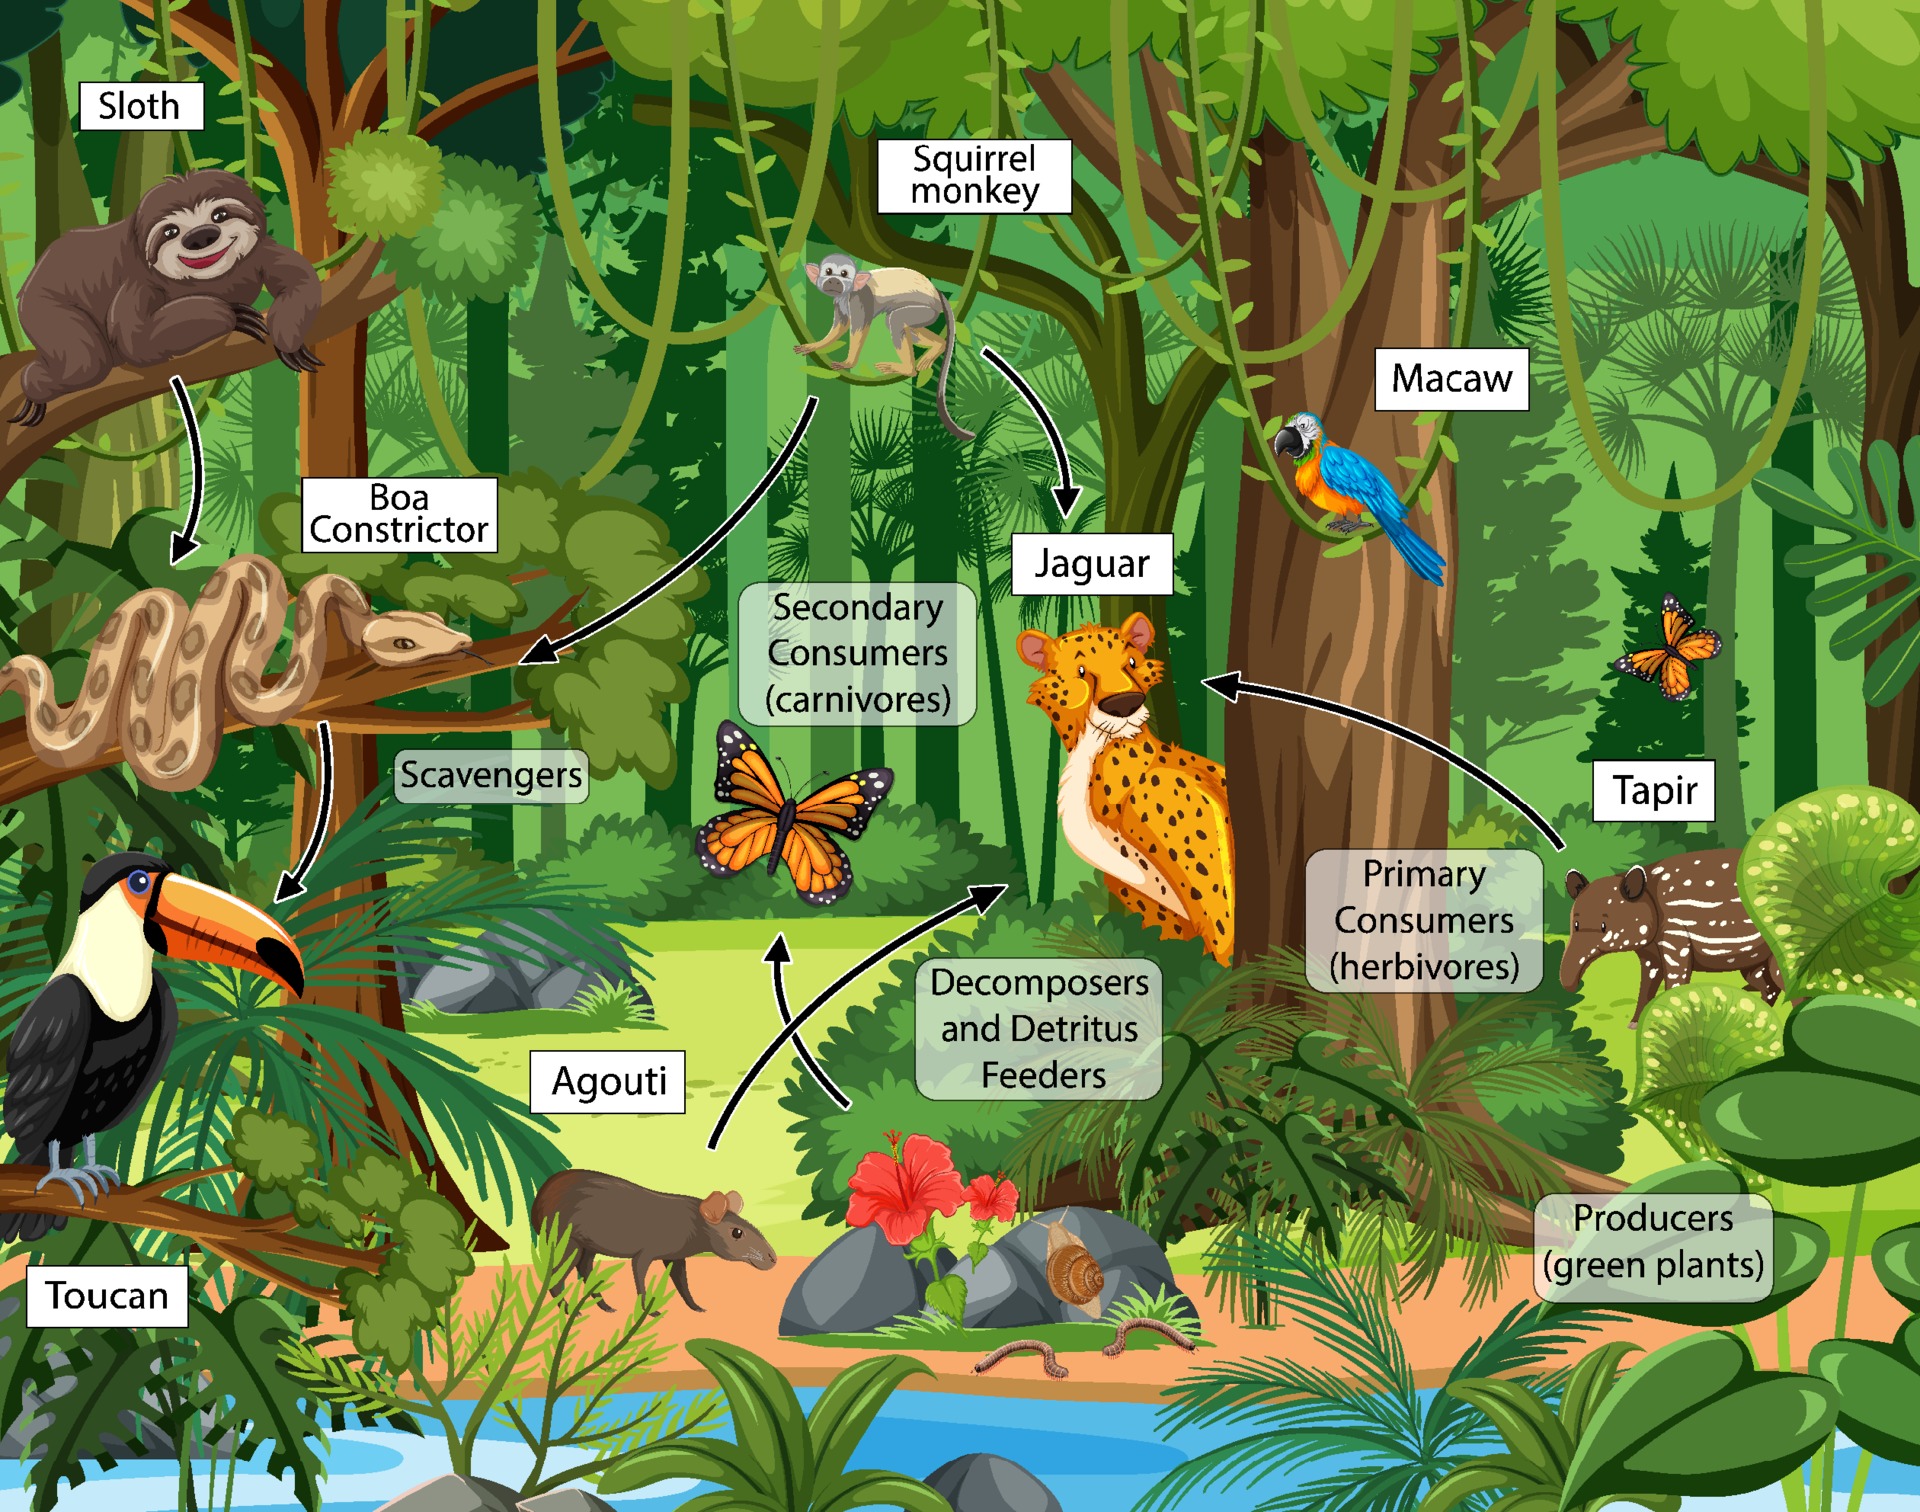
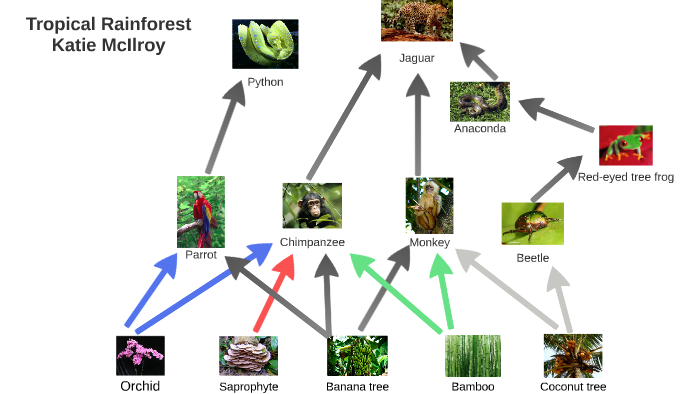
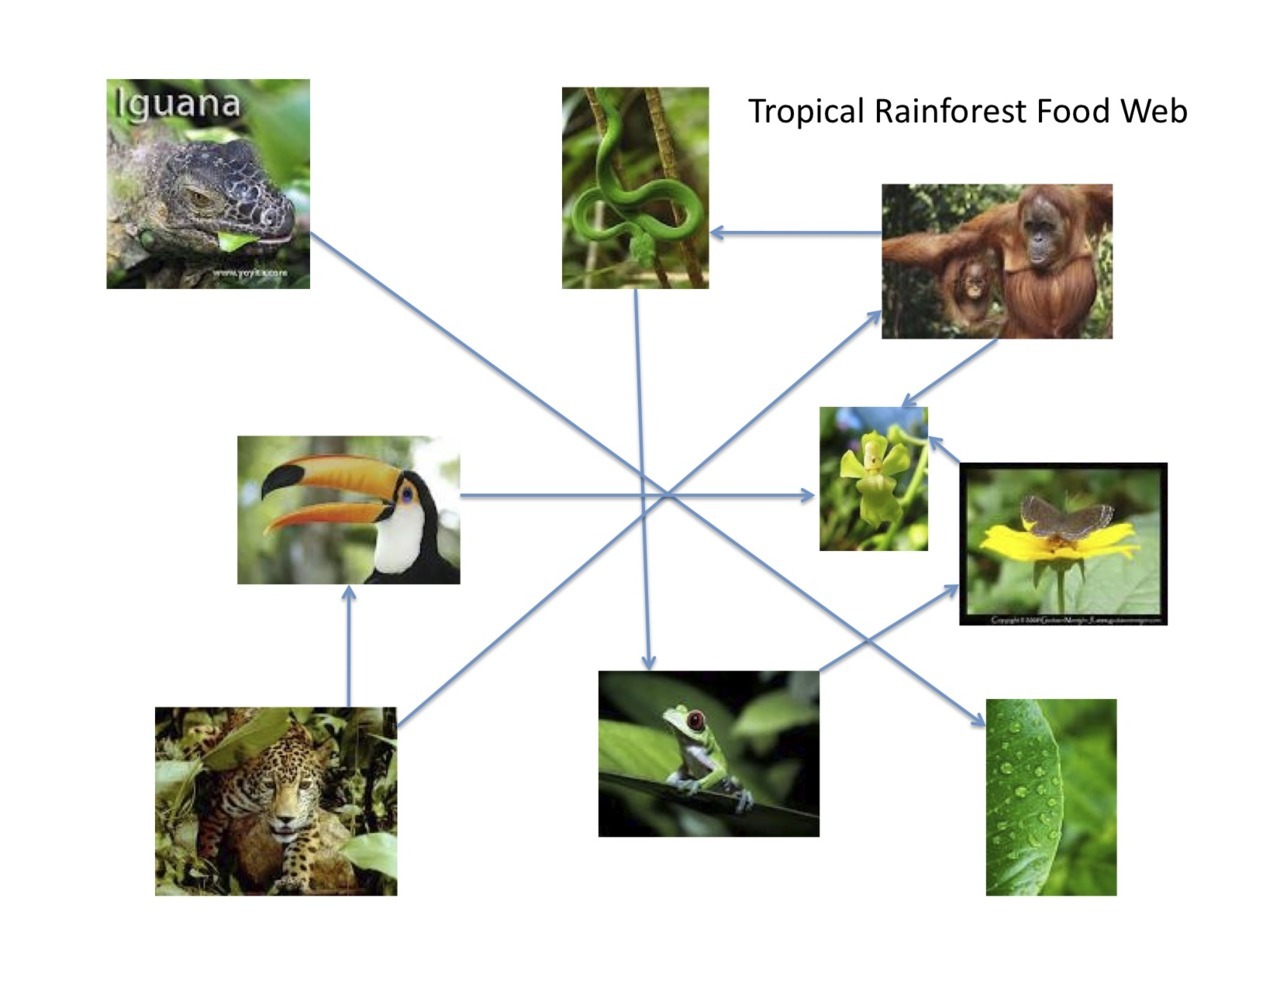
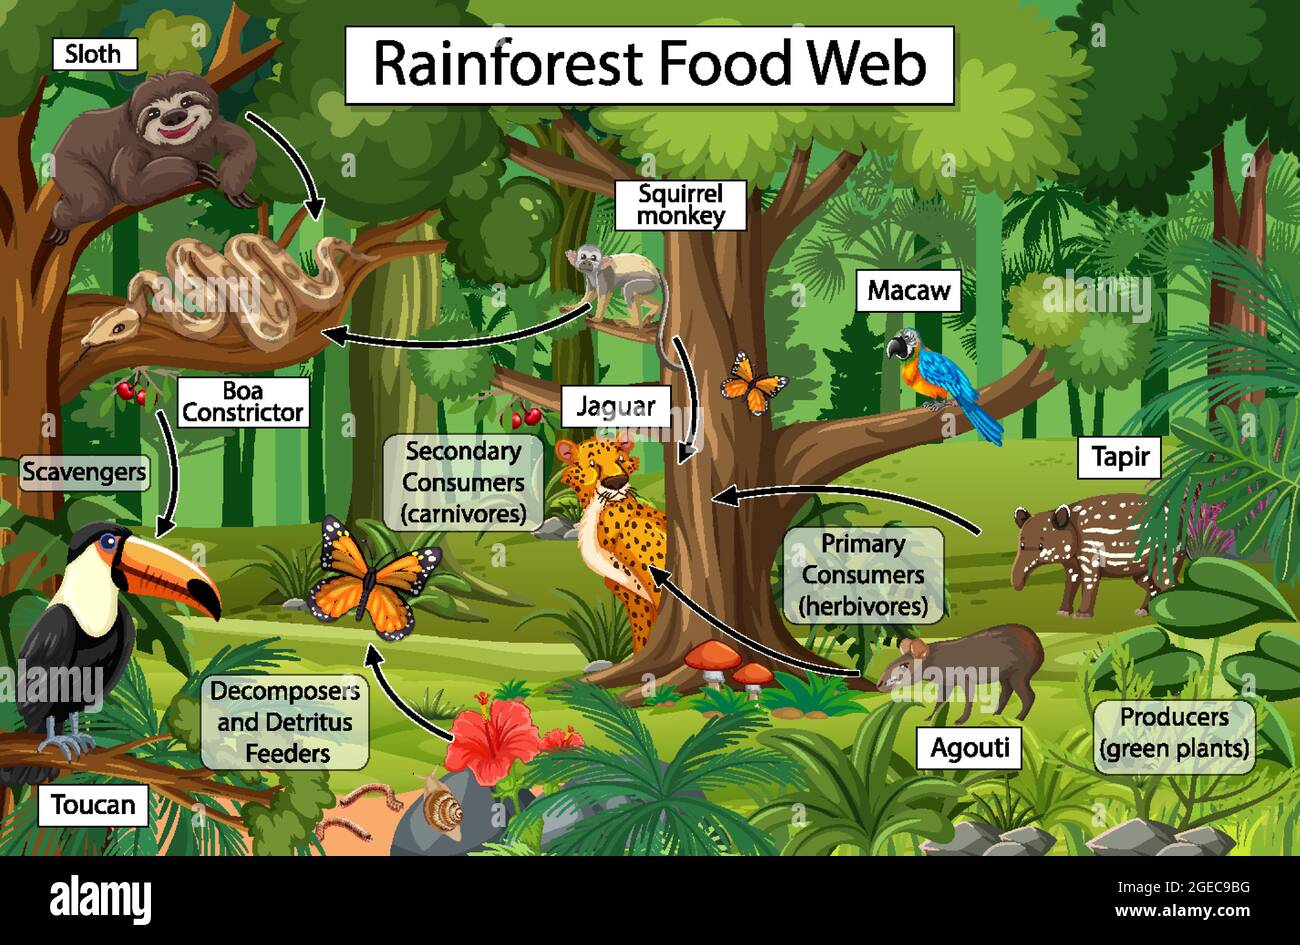
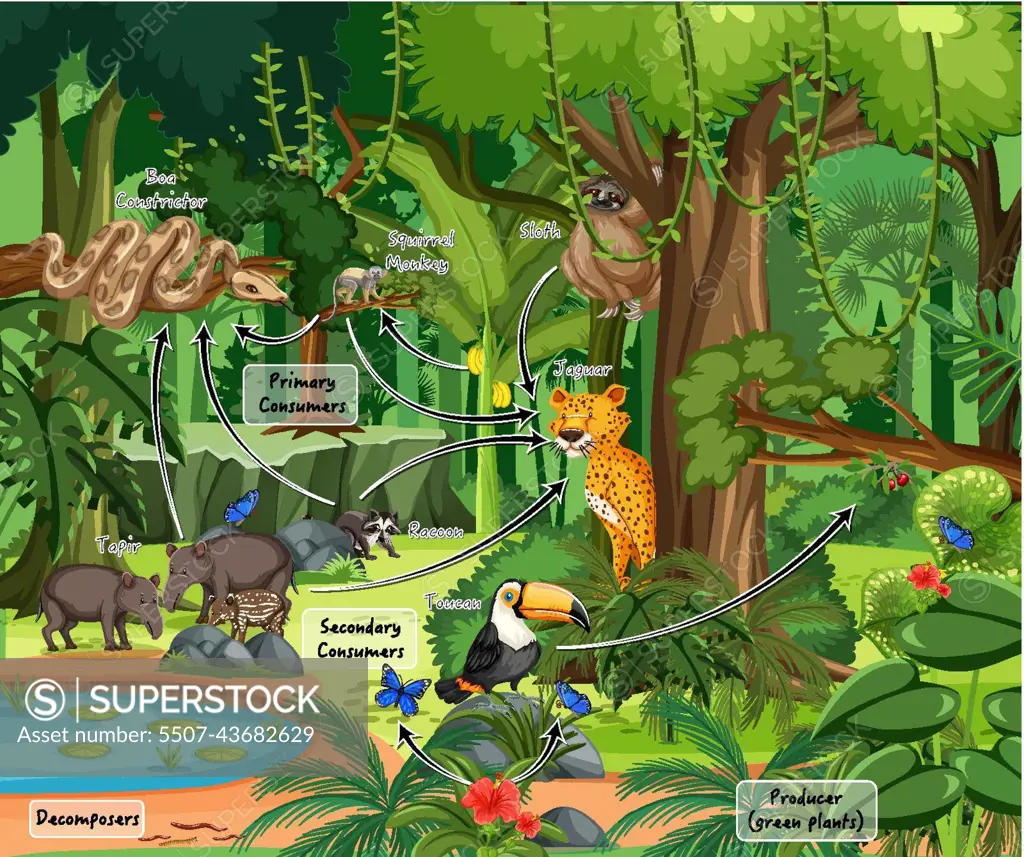
Most people think of a rainforest food web as a simple chain: leaf eats insect, bird eats insect, snake eats bird. It is more complicated than that, and not just because of variety. The actual connections shift with season, microhabitat, and the presence of keystone species that most field guides never mention. Start by picking a transect. I usually work with a 50-meter by 50-meter plot in the understory and mid-canopy layers. You map every species you can identify, then you spend time documenting who eats whom. That second part is where most people give up. You cannot just read a paper and copy someone else's connections. Every site has its own version of the web, even if the species look the same on paper. The practical approach is gut content analysis combined with direct observation over at least three months. I have spent a full wet season watching how frugivorous birds drop seeds and how those seeds get consumed by detritivores on the forest floor. The detritus layer alone accounts for roughly 40 to 60 percent of energy flow in these systems. That number changes by site, but it is always significant.
You also need to account for omnivory. A lot of beginner models treat organisms as either herbivore or carnivore, which breaks down fast in real rainforest data. The long-tailed macaque eats fruit, insects, and small vertebrates depending on what is available that month. If you force it into one trophic level, your model looks wrong almost immediately. When I was building a local food web for a conservation assessment in Borneo, I hit a specific problem with missing links around fig wasps. The literature listed figs as a primary producer and various hornbills as consumers, but the intermediate step was completely undocumented in our area. Without the wasp connection, the fig tree looked like an isolated node that pulled energy from nowhere. I solved it by collecting fallen figs and rearing the wasps in mesh cages for about six weeks. Once I identified the wasp species, I could link the pathway correctly. The hornbill actually depends on that wasp biomass indirectly, through the fruit production cycle. The web made sense again.
Energy Flow and Trophic Levels
Tropical rainforest ecosystems typically run through five to six trophic levels, though the efficiency between each level is about 10 percent, same as most terrestrial biomes. What makes the tropics different is the sheer number of parallel pathways. A single sheet beetle might be eaten by a jumping spider, a ground beetle, and a small frog, each of which feeds into a different predator cluster. This redundancy is what keeps the system stable when one prey population crashes. The canopy layer introduces a separate food web that overlaps with the understory one but operates on a different time scale. Epiphytes produce biomass that drops seasonally, and the flush of detritivores following a heavy leaf fall creates a pulse that cascades upward. I have seen bat populations spike two weeks after a major epiphyte bloom, simply because the insect prey base exploded. Any model that ignores the vertical stratification will miss those pulses entirely. A counter-intuitive point that people often miss is that the top predators in tropical rainforests are not always the largest animals. The harpy eagle is an apex predator, but in many plots the real top-down control comes from medium-sized carnivores like the ocelot or the clouded leopard. They regulate mesopredator populations that would otherwise decimate ground-nesting bird colonies. Remove the ocelot, and the rodent and small bird numbers shift in ways that ripple through seed predation and dispersal.
Get the Full Details
Common Pitfalls When Modeling These Systems
One mistake I see constantly is treating mutualisms as optional connections. Mycorrhizal fungi are not background decoration. They channel a large portion of carbon from trees into the soil food web, supporting nematodes, protozoa, and the decomposers that feed the next trophic level. Skip the fungi, and your web underestimates decomposition pathways by a wide margin. Another pitfall is assuming static connectivity. Tropical rainforest food webs respond quickly to drought. During El Niño years, fruiting frequency drops across multiple tree species, and frugivores switch to alternative food sources or migrate. The web does not break, but the dominant pathways change. If your model is built on data from a single wet season, it will look reasonable until the next dry period hits. I recommend running your web model through a sensitivity analysis before presenting it to anyone. Remove the most connected node and see what collapses. Then remove a low-connectance node and watch the difference. The nodes that cause disproportionate collapse are your keystone species, and those are the ones that matter for conservation decisions.
Data Collection Methods That Actually Work
Roadside surveys miss most of the web. The species closest to trails are the generalists, and they skew your connectivity data toward common interactions. I use camera traps paired with scat analysis for the mammal layer, fruit trap networks for the understory plant output, and light traps for nocturnal insect abundance. Covering all four layers takes roughly eight to ten weeks of field time per site, but it cuts the uncertainty in half compared to relying on existing literature alone. Stable isotope analysis is worth the cost if you can afford it. Carbon and nitrogen isotope ratios in tissue samples give you a direct read on trophic position without relying on observational guesses. I usually sample 20 to 30 individuals per major species group. The results confirm whether your assumed diet matches what the animals are actually metabolizing, and it flags opportunistic feeding events that observation alone would miss. The final web should include directional arrows with estimated biomass flow rates, not just presence or absence of connections. A link that shows "bird eats insect" tells you nothing about how much energy moves through that pathway. Adding rough biomass estimates, even if they are order-of-magnitude approximations, makes the model useful for comparison across sites.
When This Approach Falls Short
Food web modeling in tropical rainforests does not work well in areas with extreme logging history. Disturbed plots lose specialist species first, and the remaining web becomes dominated by generalist connections that look stable but are actually fragile. If you build a model from disturbed site data and apply it to an undisturbed reference site, the predictions will be off. The workaround is to sample both and build separate models, then overlay them to see where the structural differences lie. You also cannot resolve fungal and microbial pathways with standard field methods. If your question requires that level of detail, you need DNA metabarcoding of soil samples, which is a separate project with its own budget and timeline. Mixing that into a basic food web exercise usually just slows everything down without improving the visible pathways. I keep a running spreadsheet of all collected links with source citations, date of observation, and confidence rating. The spreadsheet gets messy fast, but it saves hours when you realize three weeks later that you double-counted a predator-prey pair or missed a seasonal switch in diet. The alternative is spending days reconciling inconsistent notes after the fact.