What Actually Holds a Lipid Together
Lipids are a messy category. They do not share one clean structural feature the way amino acids share a backbone. What they do share is that they are hydrophobic or amphipathic, meaning they do not dissolve well in water. This single property drives everything else about how they behave in formulation, in membranes, and in your body. I spent years working with lipid formulations for drug delivery, and the first thing you learn is that calling something a "lipid" is almost never enough information. You need to know the headgroup, the chain length, the saturation level, and the stereochemistry. Miss any of those and your results will drift.
General Structure Of Lipids
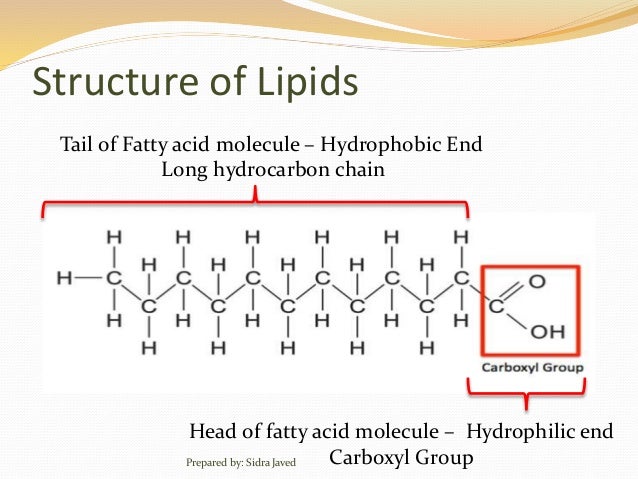
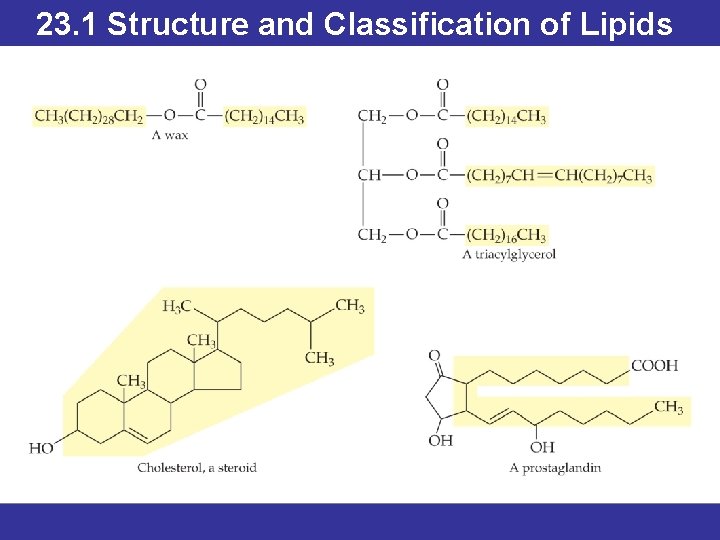
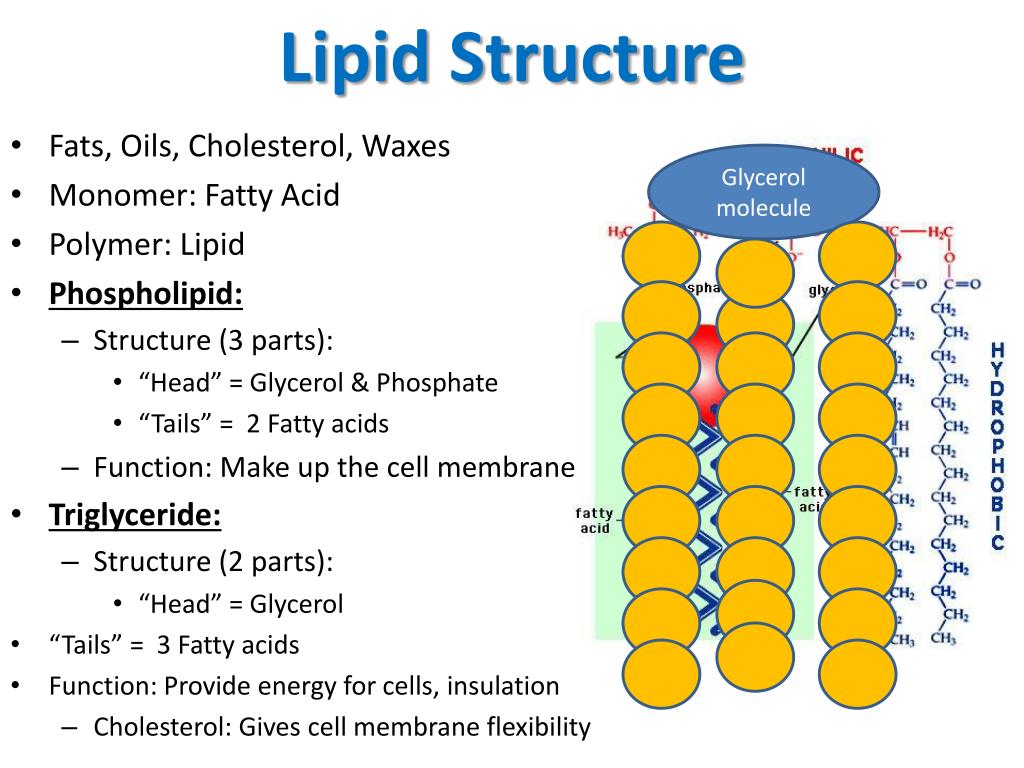
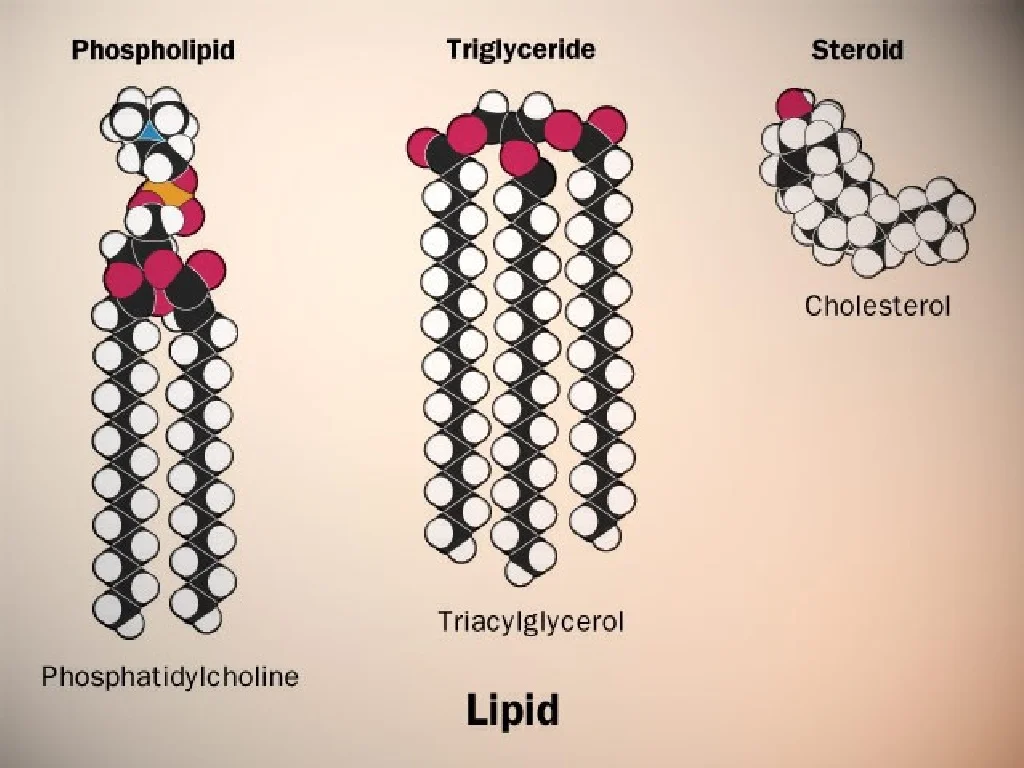
At the basic level, a lipid has a hydrophobic tail region and sometimes a hydrophilic head. The tail is usually made of hydrocarbon chains — either fatty acid chains or isoprenoid units. The head can be a phosphate group, a sugar, an alcohol, or nothing at all depending on the lipid class. The most common lipids you will encounter are triglycerides, phospholipids, sterols, and sphingolipids. Each has a different architecture, and that architecture determines packing, phase behavior, and stability. A phosphatidylcholine molecule packs very differently from a cholesterol molecule even though both are called lipids. They are not interchangeable in any practical sense. Triglycerides have three fatty acids esterified to a glycerol backbone. The fatty acids can vary in length from 4 to 24 carbons and in saturation from fully saturated to polyunsaturated with up to six double bonds. This variability matters enormously. A triglyceride with long saturated chains is solid at room temperature. One with short unsaturated chains is liquid. Same basic structure, completely different physical state.
Phospholipids add a phosphate-containing headgroup to two fatty acid chains on glycerol. The headgroup determines charge and hydration. Phosphatidylcholine is zwitterionic and neutral at physiological pH. Phosphatidylserine carries a net negative charge. Phosphatidic acid is strongly acidic. These charge differences affect everything from micelle formation to protein binding to formulation shelf life.
Get the Full Details
How Lipid Structure Dictates Behavior
The hydrocarbon chains are not just passive bulk. Their length and saturation control the phase transition temperature, which is the temperature at which the lipid moves from a gel-like ordered state to a fluid disordered state. For a typical phospholipid with two 16-carbon saturated chains, that transition is around 41 degrees Celsius. Change one double bond and you drop it by roughly 20 to 30 degrees. Change the chain length by two carbons and you shift it by about 5 to 10 degrees. This is not abstract. When I was optimizing lipid nanoparticle formulations, I had a batch where the ionizable lipid had an extra double bond that I had not specified correctly in the procurement document. The particle size distribution widened from 80 nanometers to over 200 nanometers, and the encapsulation efficiency dropped by nearly half. The structural difference was one double bond. The practical consequence was a completely failed formulation run. Chain packing is governed by van der Waals interactions between the hydrocarbon tails. Longer chains pack more tightly. Saturated chains pack more tightly than unsaturated ones because double bonds introduce kinks that prevent close approach. Cis double bonds are worse for packing than trans double bonds. Natural lipids almost exclusively have cis configuration, which is why vegetable oils are liquid and animal fats are solid at the same temperature.
The headgroup region controls hydration and interfacial properties. Phosphatidylcholine has a large hydrated head that promotes curvature and prevents tight packing. This is why it is commonly used in liposome formulations where you want stable vesicles rather than flat bilayers. Headgroup size relative to tail cross-section determines the critical packing parameter, which predicts whether the lipid will form micelles, bilayers, or inverted structures.
Common Structural Variations You Will Encounter
Sphingolipids use sphingoid base instead of glycerol. Ceramide is the simplest sphingolipid with a fatty amide-linked to a sphingoid base. Add a phosphorylcholine and you get sphingomyelin, which behaves similarly to phosphatidylcholine but has different metabolic pathways. Add sugar groups and you get glycolipids like cerebrosides and gangliosides. These are abundant in neural tissue and play roles in cell recognition that phosphoglycerides do not. Sterols are structurally unrelated to the other classes. Cholesterol has four fused rings and a single hydroxyl group. The ring system is rigid and planar, which means it inserts between phospholipid chains and modulates membrane fluidity in both directions. At high temperatures it restricts motion. At low temperatures it prevents tight packing. This bidirectional effect is why cholesterol is present in nearly all animal cell membranes. Wax esters are simple esters of long-chain fatty alcohols and long-chain fatty acids. They have no headgroup and are extremely hydrophobic. Beeswax, lanolin, and jet oil are common examples. In formulation contexts they are useful as barriers and emollients but generally not as carriers because they do not form organized structures in water.
Polyketides and terpenes are biosynthetic lipid classes that do not follow the fatty acid ester pattern. They are important in medicinal chemistry but less relevant for structural biology or formulation work. If you are working with membranes or drug delivery, you will encounter them rarely.
Structural Determinants of Stability and Degradation
Unsaturated lipids oxidize. This is not a minor issue. Double bonds are sites of radical attack, and lipid peroxidation propagates through adjacent molecules in a chain reaction. The rate depends on the number of double bonds, their proximity to the ester linkage, and the presence of transition metal ions. Linolenic acid with three double bonds oxidizes roughly eight times faster than oleic acid with one double bond. I learned this the hard way with a phospholipid formulation that looked stable for two weeks and then degraded rapidly. The peroxide value spiked from under 5 to over 50 in three days. The root cause was a trace amount of copper in the water phase, not the oxygen content of the headspace. Adding a chelator solved it. The structural lesson was that unsaturation level alone does not predict oxidation susceptibility if you ignore metal contamination. Hydrolysis is the other major degradation pathway. Ester bonds in triglycerides and phospholipids can hydrolyze, especially at extreme pH or elevated temperature. The rate is catalyzed by bases and by certain enzymes like phospholipases and lipases. In formulation work, you generally avoid pH below 4 or above 9 unless you have specific reason to do so. Even then, shelf life drops dramatically.
Isomerization of double bonds is a slower but real concern. Trans isomers can form during processing or storage, particularly under heat and light. These isomers have different packing properties and different biological effects. The structural change is minimal, but the functional consequences are measurable in both membrane properties and health outcomes.

When Structural Knowledge Fails You
No amount of structural analysis will predict everything. Lipid behavior in complex environments depends on impurities, processing history, and interactions with other components. A pure phosphatidylcholine sample behaves differently than a commercial preparation with 98 percent purity, because the 2 percent impurities can include lysolipids, free fatty acids, and oxidation products that act as surfactants and destabilize the system. Mixed lipid systems are even harder. Phase separation occurs when lipid compositions are incompatible, creating domains with different properties. This happens in cell membranes naturally as lipid rafts, and it happens in formulations unintentionally as precipitates or cloudiness. Identifying which lipid pairs are compatible requires experimental data, not just structural reasoning. Even advanced techniques have limits. Mass spectrometry can tell you the molecular species present. NMR can reveal ordering and dynamics. X-ray diffraction can measure lattice parameters. But none of these will tell you how your formulation will behave after six months of storage under fluctuating conditions. You still need to run stability studies.
If you are designing lipid-based systems, start with the structure, understand the constraints it imposes, and then validate experimentally. The structure tells you what is possible. It does not tell you what will work in practice without testing.