What actually controls whether a culture grows or stays dark
I spent three weeks troubleshooting a stubborn contamination in my lab's anaerobic chamber. Every plate looked identical, every incubator read the same temperature, and still one rack of cultures would grow fluffy white colonies while the adjacent rack stayed crystal clear. The problem wasn't technique. It was oxygen leakage at a rubber seal that had hardened enough to let trace amounts of air seep in without anyone noticing. That experience taught me something I didn't fully grasp from textbooks: microbial growth factors don't just turn on and off. They exist on gradients, and small deviations from set points can mean the difference between a thriving culture and nothing at all. When you're trying to Identify Factors That Affect Microbe Growth, you're really looking at a matrix of physical and chemical parameters that either permit or prevent cellular replication. The fundamental question isn't whether a microbe can grow at all. It's whether the environment meets its specific requirements for metabolism, division, and survival.
Temperature and how it shapes microbial communities
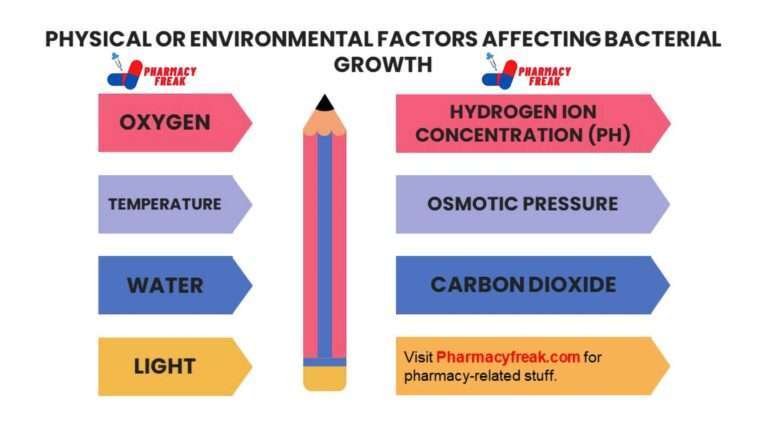
Temperature affects enzyme activity, membrane fluidity, and RNA stability. Each microorganism has a cardinal temperature range with three key points: minimum, optimum, and maximum. Below the minimum, membranes become so rigid that transport proteins stop working. Above the maximum, proteins denature and the cell collapses. Between those extremes lies the range where growth rate climbs toward its peak. Psychrophiles grow best at 15 degrees Celsius or lower and are common in deep ocean environments and permafrost. Mesophiles, which include most human pathogens and the organisms I work with daily, thrive between 20 and 45 degrees Celsius. Thermophiles and hyperthermophiles occupy hot springs and hydrothermal vents, with some hyperthermophiles growing at temperatures above 80 degrees Celsius. The practical implication here is straightforward: if you're culturing clinical isolates, 37 degrees Celsius is the standard because it matches human body temperature. But if you're investigating environmental samples, you need to match the source habitat's temperature regime or you'll miss most of what's there. I once ran a comparative study where I incubated soil samples at 25, 37, and 55 degrees Celsius. At 37 degrees, the colony count was roughly ten times higher than at 25 degrees, but at 55 degrees the organisms were entirely different. The mesophilic population crashed while thermophilic Bacillus species took over. This isn't abstract. It's why compost piles generate their own heat and shift microbial composition as they mature.
pH and the hydrogen ion concentration problem
Every culture medium has a pH, and every microbe has a pH range where it can maintain internal homeostasis. Acidophiles grow at pH values below 5. Alkaliphiles prefer pH above 9. Most bacteria sit comfortably between 6.5 and 7.5, which is why standard laboratory media are buffered around neutral pH. Fungi generally tolerate more acidic conditions, which is why adding acid to a medium can selectively suppress bacterial growth while letting molds and yeasts flourish. The mechanism is subtle but important. Intracellular pH must stay within narrow limits for enzymatic function. When external pH shifts, the cell expends ATP pumping protons in or out to compensate. Eventually the energy cost becomes unsustainable and growth stops. Some organisms produce acid as a metabolic byproduct, which further lowers the surrounding pH and creates a feedback loop that can inhibit competitors. This is lactic acid bacteria in action, and it's also why pickling works as a preservation method. One thing beginners consistently miss is that pH measurements are temperature-dependent. A buffer at 25 degrees Celsius will read differently at 37 degrees Celsius. If you calibrate your pH meter at room temperature and then measure a medium that's been warmed for incubation, your reading could be off by a meaningful amount. I always measure pH after the medium has reached its final working temperature, or I apply a temperature correction factor. It's a small step that prevents a lot of confusion.
Get the Full Details
Oxygen requirements and the Redox potential factor
Oxygen is toxic to many organisms because it forms reactive oxygen species that damage DNA, proteins, and lipids. Aerobes have the enzymatic machinery, superoxide dismutase and catalase, to neutralize these compounds. Anaerobes lack these enzymes and are killed by even brief oxygen exposure. Facultative anaerobes can switch between aerobic respiration and fermentation or anaerobic respiration depending on what's available. Microaerophiles need oxygen but only at reduced partial pressures. Capnophiles require elevated carbon dioxide concentrations. The Redox potential, measured in millivolts, is the actual parameter that determines whether an environment supports aerobic or anaerobic life. A positive Eh favors oxidation reactions. Negative Eh favors reduction. Some organisms grow at any Redox potential. Others are restricted to a narrow window. In practice, this means you can't judge anaerobic conditions by smell or appearance alone. You need indicators like resazurin or an actual Redox probe. I've seen labs attempt anaerobic cultures using just gas packs without verification, and roughly one in five runs had compromised conditions due to seal failures or indicator exhaustion. Here's a practical point that doesn't get enough attention: inoculation technique matters for oxygen-sensitive organisms. Stabbing a deep tube rather than spreading on the surface reduces oxygen exposure. Working quickly and keeping tubes capped between uses cuts exposure time. For organisms that are borderline sensitive, adding reducing agents like cysteine or sodium sulfite to the medium can lower the Redox potential chemically and give you a wider margin of error.
Osmotic pressure and water activity
Water activity, written as Aw, describes the availability of water in a system. Pure water has an Aw of 1.0. Most bacteria require Aw above 0.91. Yeasts can grow down to about 0.88. Xerophilic molds can go lower, around 0.65. When solutes like salt or sugar are added to a medium, Aw drops. Water moves out of cells by osmosis, causing plasmolysis in bacteria with cell walls and complete desiccation in those without. Halophiles have adapted by accumulating compatible solutes internally or by having cell wall and membrane compositions that resist dehydration. I've encountered a case where a research group was trying to culture a novel organism from a salt flat and couldn't get it to grow on any standard medium. The breakthrough came when someone finally tried adding sodium chloride to match the environmental concentration, around 15 percent. The organism wouldn't grow below that threshold. This is why environmental context matters. Sampling site conditions should inform your medium formulation before you start diluting and plating. Mannitol salt agar is a classic example of using osmotic pressure for selection. The 7.5 percent NaCl concentration inhibits most staphylococci bacteria while allowing Staphylococcus species to grow. The mannitol component then distinguishes pathogenic S. aureus, which ferments the sugar and produces acid, from other staphylococci that grow but don't change the pH indicator. It's a two-factor selection system working in tandem.
Nutrient availability and growth media composition
Microbes need carbon, nitrogen, sulfur, phosphorus, trace metals, and sometimes specific growth factors like vitamins. The carbon source fuels both energy production and biosynthesis. The nitrogen source feeds amino acid and nucleotide synthesis. Without any one of these, growth stops regardless of how abundant the others are. This is Liebig's law of the minimum applied to microbiology. Benchmark media like nutrient broth support a wide range of non-fastidious organisms. Selective media suppress unwanted flora. Differential media reveal metabolic capabilities through visible changes. The choice depends entirely on what you're trying to isolate or quantify. If you're doing environmental sampling, complex media like tryptic soy agar will recover more organisms than defined synthetic media because you don't know in advance what growth factors the inhabitants might need. But if you're quantifying a specific organism or studying metabolic pathways, defined media eliminate variables and let you control exactly what's available. A common mistake is assuming that more nutrients always means faster growth. At high concentrations, nutrients can become inhibitory. Excess salts create osmotic stress. Some carbon sources at high levels can cause catabolite repression, where the preferred sugar is consumed first and other metabolic pathways are suppressed until it's exhausted. This is the diauxic growth phenomenon that Monod described, and it's visible as two distinct growth phases on a turbidity curve when glucose and lactose are both present.
Moisture and the role of water in microbial life
Water is the solvent in which all cellular chemistry occurs. Without adequate moisture, metabolic reactions slow dramatically or stop entirely. Desiccation-resistant organisms like bacterial spores and fungal conidia can survive for years in dry conditions but won't grow until water is available. This is why food preservation through drying works and why sterilization protocols that rely on dry heat require higher temperatures and longer exposure times than moist heat methods like autoclaving. In laboratory settings, humidity control around incubators and storage areas affects medium quality. Agar plates stored in dry conditions lose moisture through the lid, and the resulting shrinkage concentrates the medium components and lowers Aw. This subtly changes growth characteristics and can inhibit sensitive organisms. I store plates inverted in sealed bags with a moisture-retention barrier, and I check for condensation on the lid surface as a quick quality indicator. Plates that are too dry show a shiny, cracked agar surface. Plates that are too wet show heavy condensation, which can cause colonies to merge and spread.
Radiation and other physical stressors
Ultraviolet light damages DNA by forming pyrimidine dimers. Ionizing radiation like X-rays and gamma rays causes strand breaks and generates reactive radicals. Both can kill microbes or induce mutations. The response varies widely. Deinococcus radiodurans tolerates doses that would shatter a human genome. Standard E. coli dies at fractions of those levels. UV germicidal lamps are effective for surface decontamination but don't penetrate well, so shadowed areas remain untreated. This is a limitation worth remembering when validating disinfection protocols. Filter sterilization at 0.22 micrometers removes bacteria and most fungi but not viruses or mollicutes like Mycoplasma, which are smaller than the pore size. If you're working with cell cultures, Mycoplasma contamination is a silent killer that doesn't affect turbidity but depletes nutrients and alters cell behavior. Detection requires PCR or specific staining, not routine plating on bacteriological media.
Practical identification framework
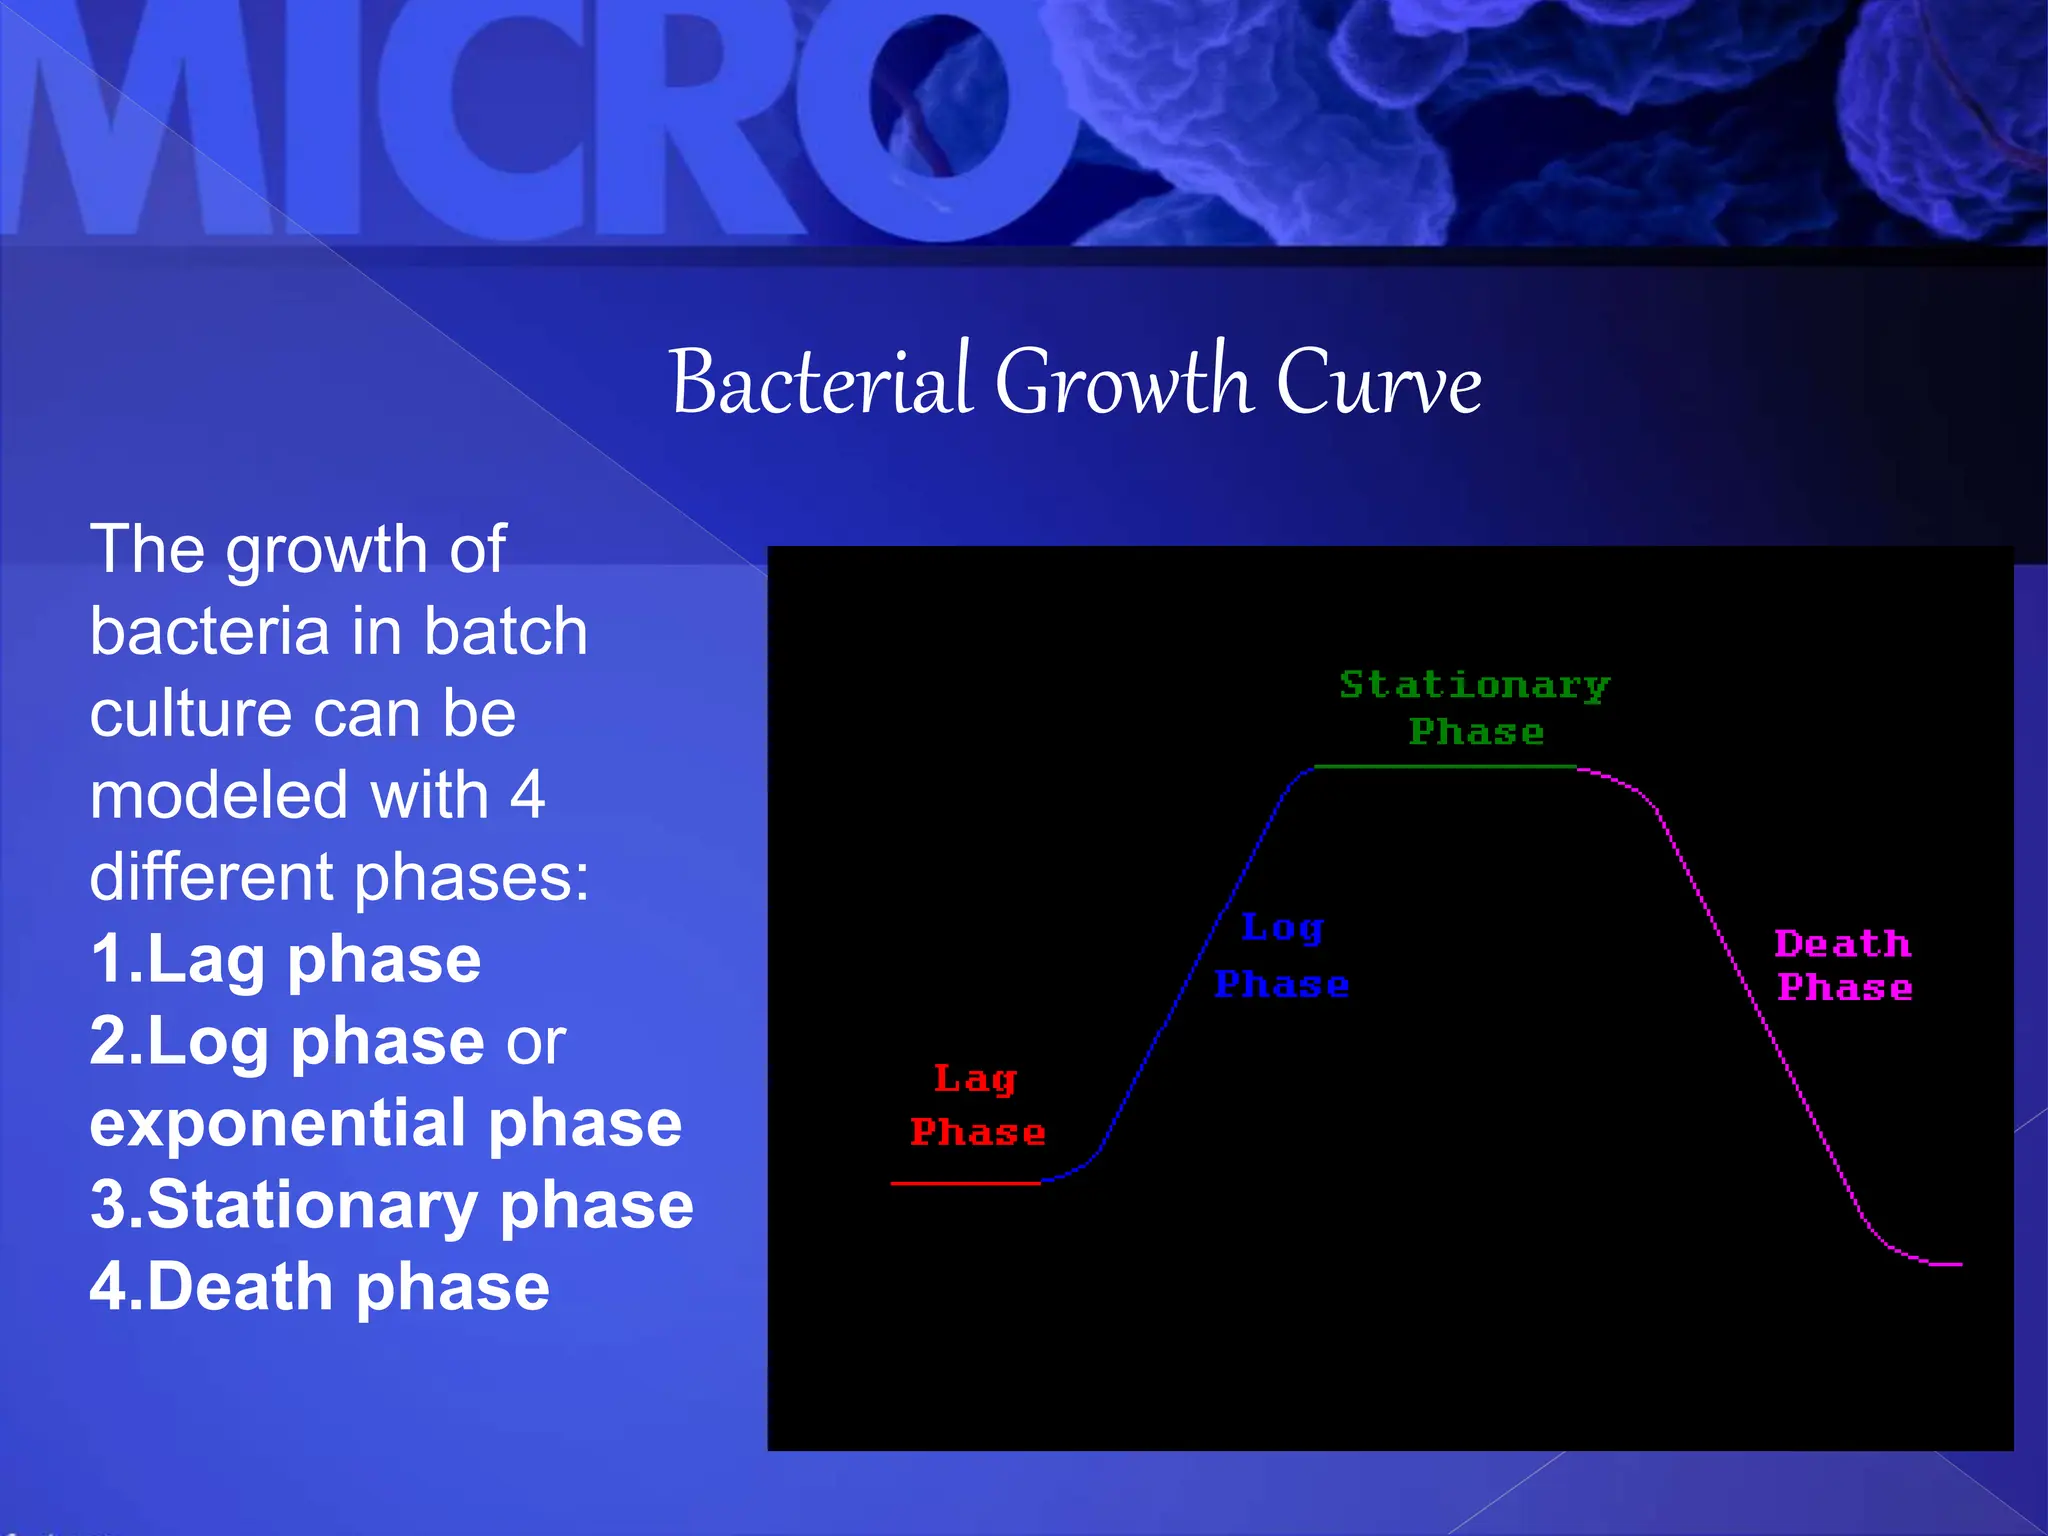
When you're systematically working through the process of identifying factors that affect microbe growth, the most reliable approach is to vary one parameter at a time while holding everything else constant. Change temperature and pH simultaneously and you won't know which variable caused the observed effect. Serial dilution of a single factor across a gradient of conditions reveals the actual tolerance range rather than a binary grow-or-don't-grow result. Growth curves are the standard tool for quantifying the effect of any factor. Lag phase duration, exponential growth rate, and carrying capacity each respond differently to environmental changes. A suboptimal temperature might lengthen the lag phase without affecting the maximum growth rate. A inhibitory pH might reduce the carrying capacity while leaving the exponential rate relatively intact. These distinctions matter when you're optimizing conditions for industrial fermentation or diagnosing a problematic culture. For rapid screening of multiple factors, microdilution plates with checkerboard or fractional factorial designs let you test numerous condition combinations in a single experiment. You can map out a growth landscape across temperature, pH, salt concentration, and nutrient level in a format that uses minimal media and incubation time. The data output requires statistical analysis but pays for itself quickly when you're characterizing an unfamiliar organism or optimizing a production strain.

Common pitfalls when assessing growth conditions
The first pitfall is assuming that growth on a standard medium tells you everything about an organism's ecology. Most environmental bacteria don't grow on routine laboratory media. The great plate count anomaly, the observation that direct microscopic counts far exceed colony counts on agar, is well documented. Your isolation conditions select for a small fraction of the community. If you want to understand the full growth factor profile of an environmental sample, you need environmental simulation techniques like diffusion chambers or iChip devices that let organisms grow in their native substrate while still being isolated on solid media. The second pitfall is ignoring inoculum size. A heavy inoculum can overwhelm weak selective pressures. A light inoculum might fail to establish even in permissive conditions due to stochastic effects or quorum sensing delays. Consistent inoculation density, typically standardized to a 0.5 McFarland turbidity equivalent, is essential for reproducible results. I use a spectrophotometer at 600 nanometers to verify density rather than relying on visual matching, which is subjective and varies with instrument path length. The third pitfall is conflating growth with survival. An organism might remain viable without dividing under conditions that suppress growth. Viability stains like Live/Dead kits or plate counts after extended incubation can reveal this distinction. Stress responses, general stress sigmas, and stationary phase adaptation can allow persistence long after active growth has ceased. If your experiment measures growth rate but your question is about survival, you need to adjust your readout accordingly.
Identifying factors that affect microbe growth is ultimately about understanding the intersection between organismal physiology and environmental chemistry. The parameters are well catalogued. The complexity comes from their interactions and from the fact that every organism has a unique fingerprint across those parameters. The most useful skill isn't memorizing cardinal values. It's designing experiments that reveal what matters for your specific question, recognizing when your method is missing something, and knowing which conditions to adjust when growth doesn't behave as expected.