What Independent Assortment Definition Biology Actually Means in the Lab
You open a textbook and it says independent assortment happens during meiosis when chromosomes line up randomly. That's technically true and completely useless if you've ever tried to apply it to a real genetics problem. The independent assortment definition biology teachers usually give you is a starting point, not the full story. Here's how it actually plays out when you're working with organisms, calculating ratios, or trying to figure out why your testcross results don't match the expected 9:3:3:1 ratio. I spent three semesters struggling with dihybrid crosses before I stopped treating Mendel's laws like gospel and started treating them like approximations. The core idea is straightforward enough: alleles for different traits segregate independently of one another during gamete formation. But "straightforward" in textbooks and "straightforward" in practice are two different things. The reason is that real genes don't always behave like the idealized examples in chapter four of any intro biology book.
Independent Assortment Definition Biology — The Real Version
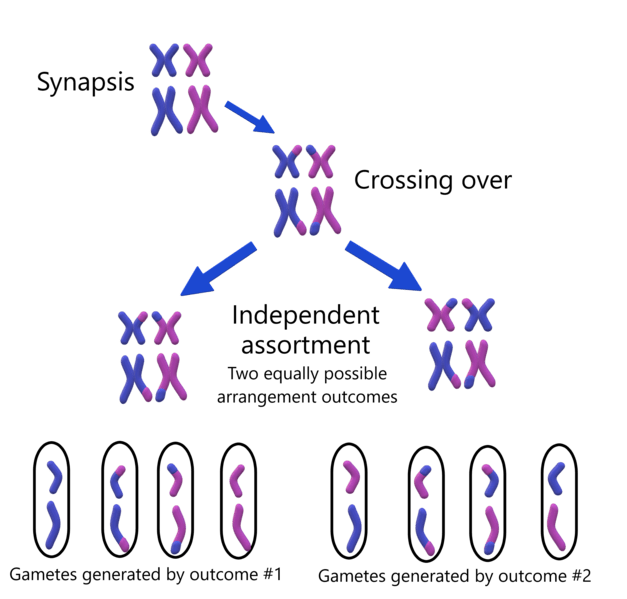
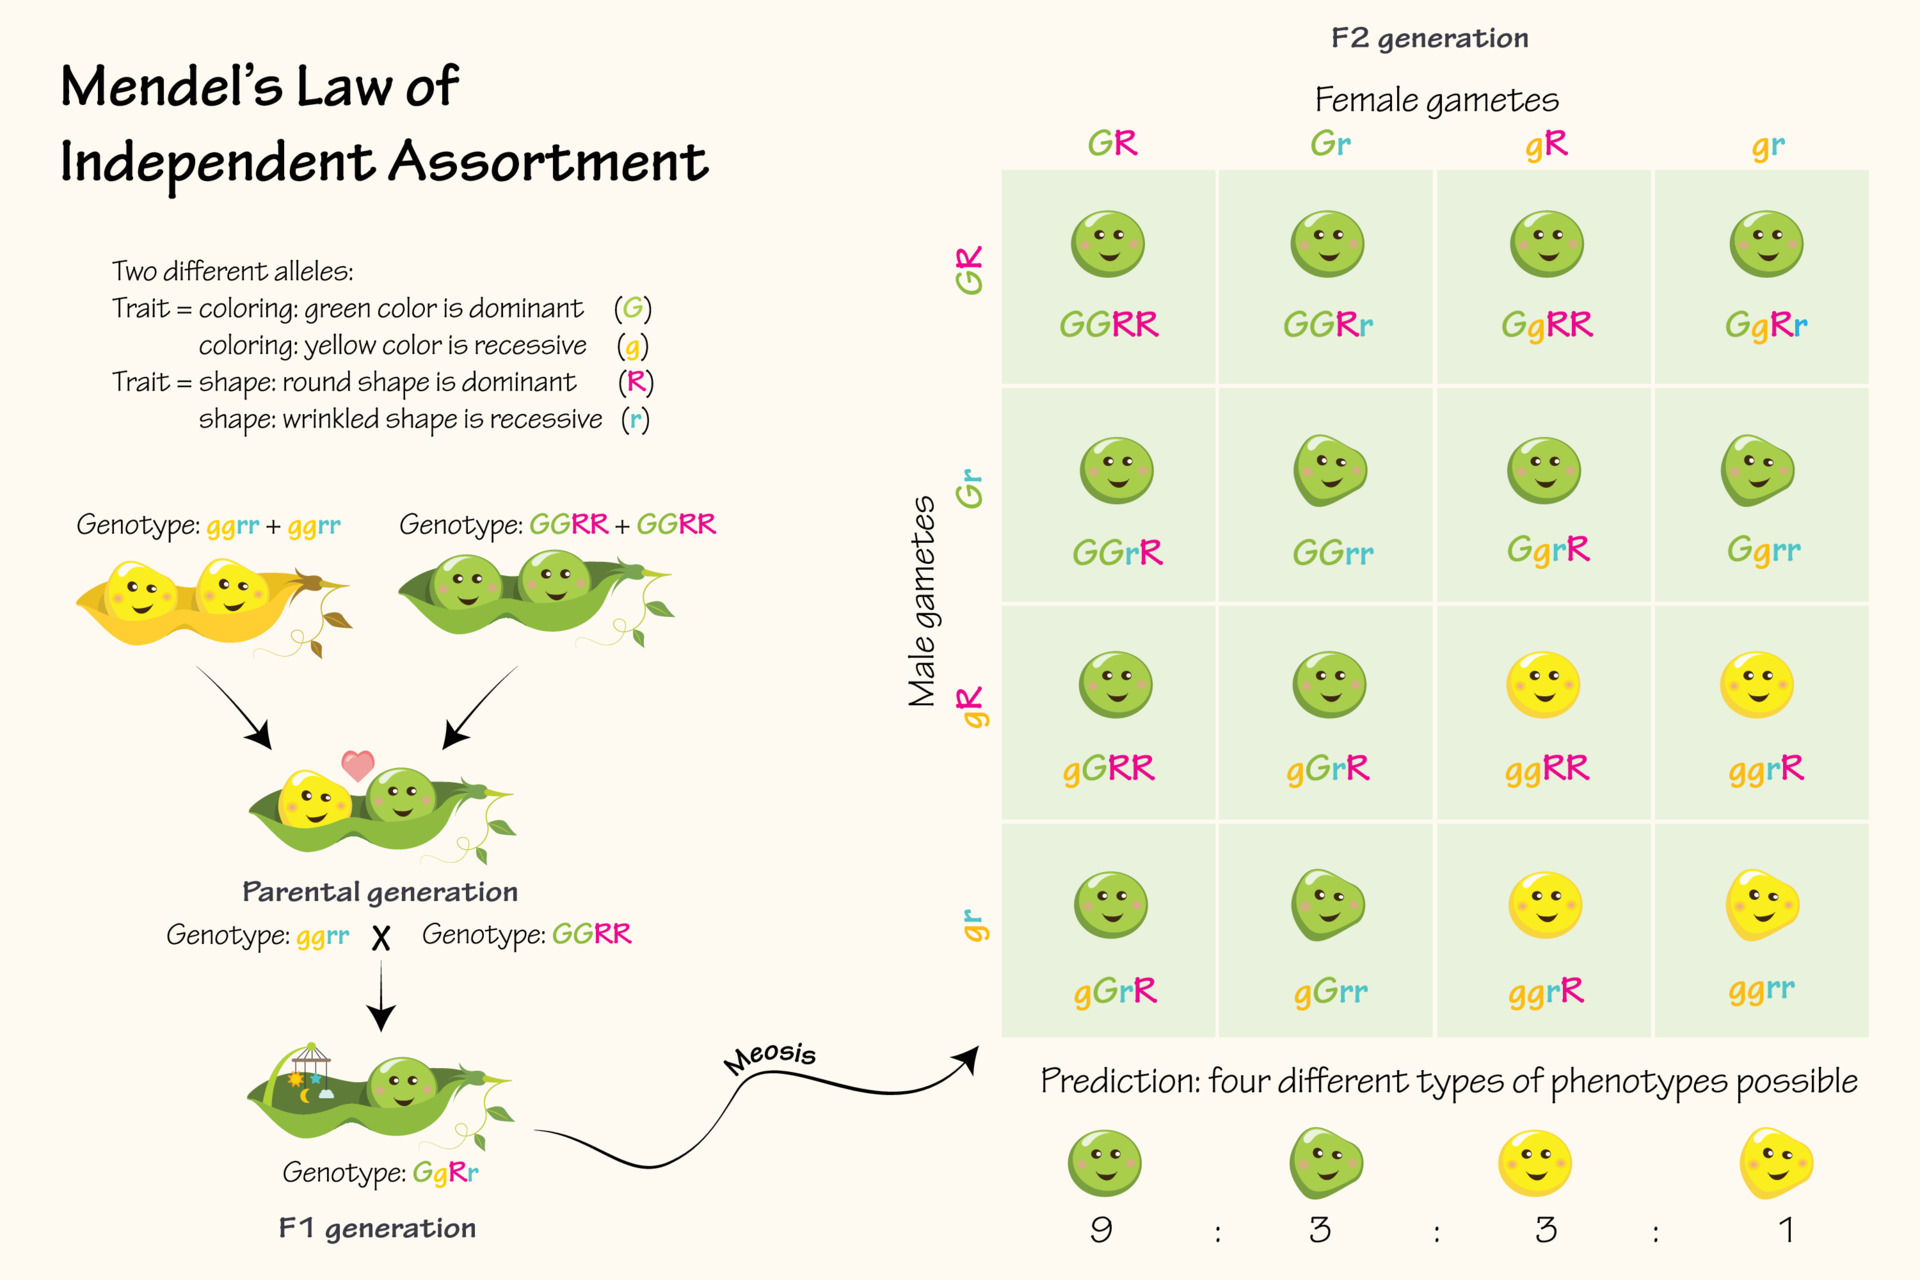
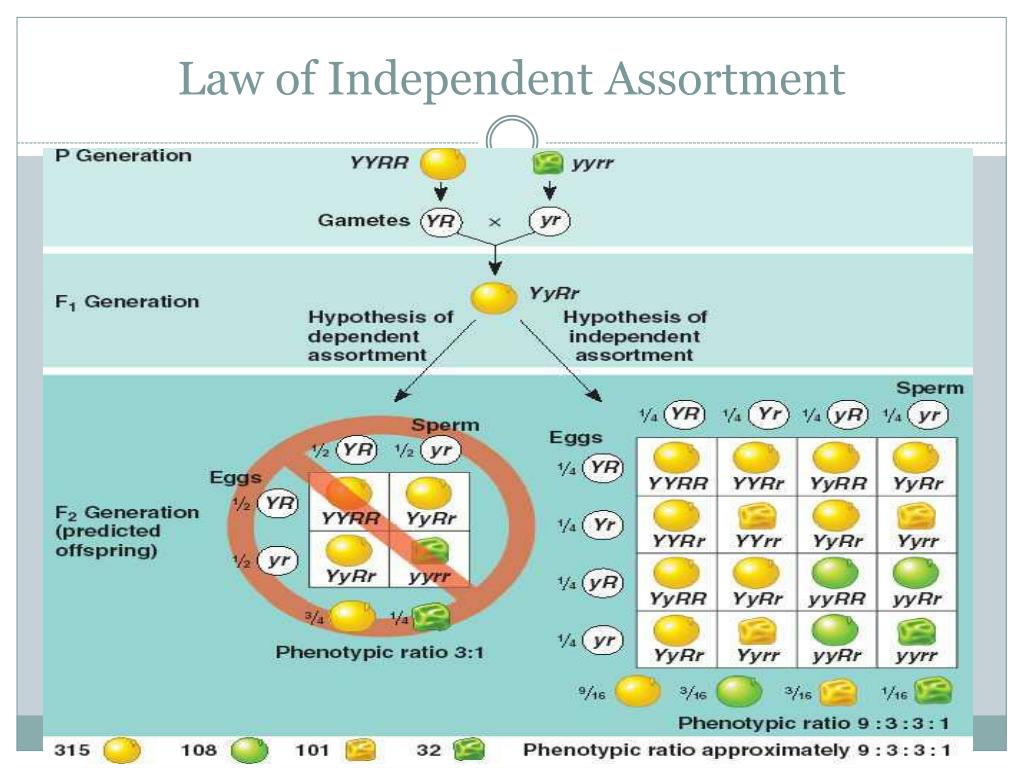
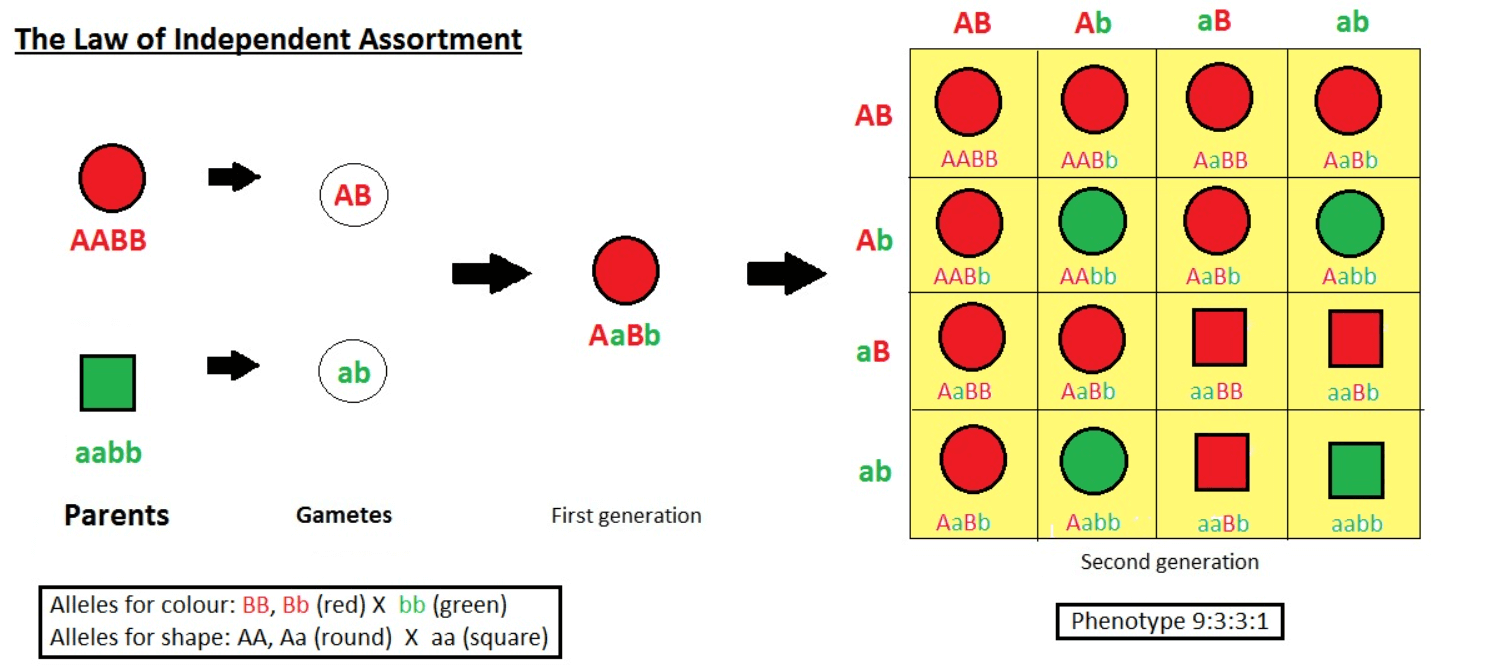
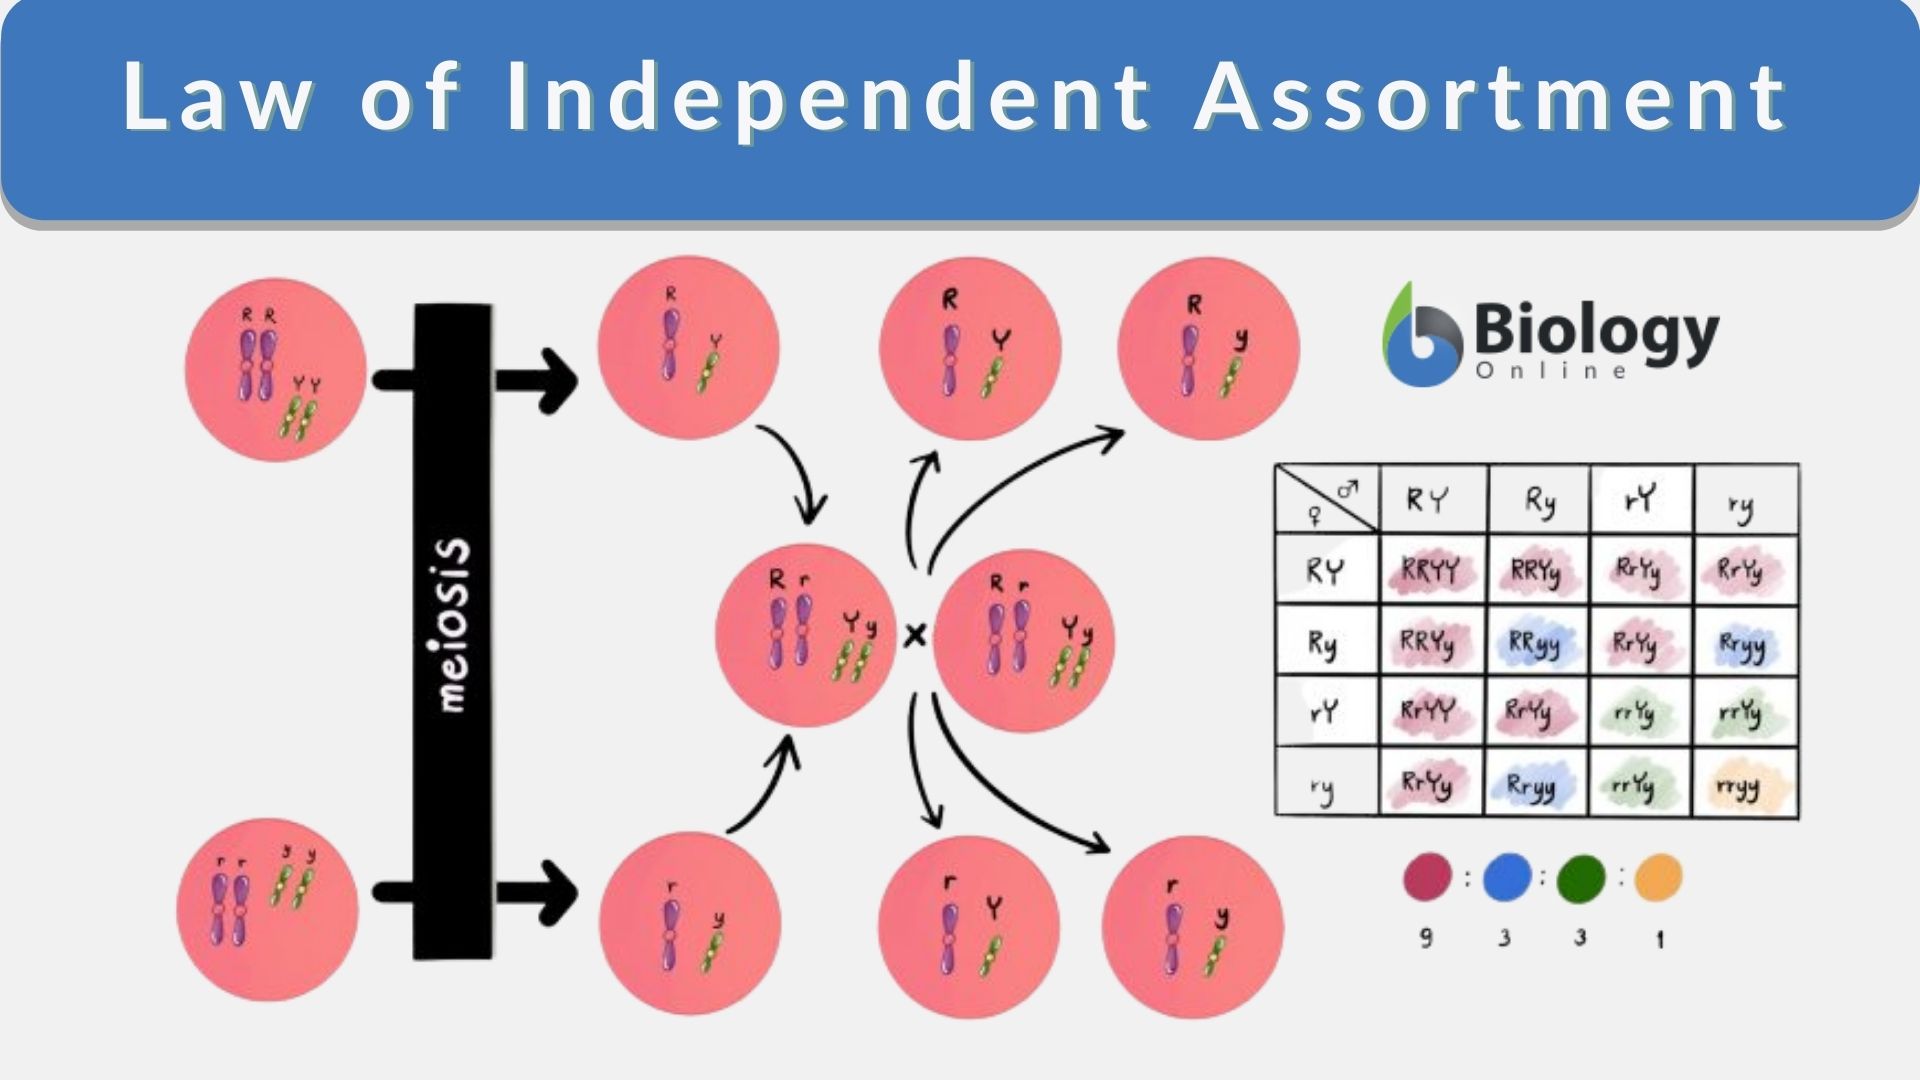
Independent assortment states that the inheritance of one trait does not influence the inheritance of another trait, provided the genes are located on different chromosomes or are far enough apart on the same chromosome to behave as if they're unlinked. During metaphase I of meiosis, homologous chromosome pairs orient randomly at the cell equator. Each pair's orientation is independent of every other pair. This randomness is what generates new allele combinations in the gametes. For a organism that is heterozygous at two loci, this produces four equally probable gamete types instead of just two parental types. The practical consequence is that when you cross two dihybrids, you expect a 9:3:3:1 phenotypic ratio in the F2 generation under complete dominance at both loci. That ratio assumes three things: the genes are on different chromosomes, there is no epistasis interacting with them, and the sample size is large enough that random sampling error doesn't distort the numbers. Miss any one of those and your data will look nothing like the textbook diagram. I learned this the hard way when I was grading undergraduate lab reports on pea plant crosses. Students would set up a dihybrid cross between plants heterozygous for seed color and seed shape, grow out the F2 generation, and get ratios like 7:5:4:2 instead of 9:3:3:1. They'd immediately declare the experiment a failure and move on. The actual problem was that they were using a species where those two genes happened to be linked on the same chromosome with roughly 15 map units between them. The independent assortment definition still applied conceptually, but the physical linkage meant the expected ratio was completely wrong. I had them run a testcross instead of an F1 self-cross and calculate recombination frequency from the progeny distribution. That single change turned a "failed experiment" into a legitimate mapping exercise and taught them more than any correct textbook example ever could.
Here's another thing most courses skip over: independent assortment only creates new combinations of existing alleles. It does not create new alleles. Mutation does that. Recombination within a gene does that. What independent assortment does is reshuffle the deck so that the alleles you already have end up in new combinations across different gametes. This distinction matters when you're thinking about sources of genetic variation in a population. Sexual reproduction generates diversity through independent assortment, crossing over, and random fertilization. All three mechanisms contribute, but they operate at completely different levels. Independent assortment acts at the chromosome level during meiosis I. Crossing over acts at the chromatin level during prophase I. Random fertilization acts after meiosis is complete when sperm and egg fuse. The chromosome number of an organism directly determines how many different gamete types independent assortment can produce. An organism with n=3 can theoretically produce 2^3 or 8 distinct gamete types from independent assortment alone. An organism with n=23, like a human, can produce 2^23 or about 8.4 million different chromosomal combinations in gametes without even counting crossing over. That's a lower bound because crossing over adds another layer of variation on top of whatever independent assortment contributes. Most students understand the math but don't connect it to the actual biological mechanism until they see a karyotype and trace which chromosomes go to which pole during anaphase I. There are hard limits to when independent assortment breaks down. Genes on the same chromosome that are close together will not assort independently regardless of how many offspring you score. Genes on sex chromosomes follow different inheritance patterns altogether. Mitochondrial and chloroplast genes are inherited through cytoplasmic pathways that bypass meiotic assortment entirely. Polygenic traits controlled by multiple genes don't produce clean phenotypic ratios because environmental factors and gene-gene interactions blur the categories you're trying to count. And in organisms with complex chromosomal arrangements like inversions or translocations, the physical behavior of chromosomes during meiosis can suppress or distort the expected assortment patterns.
Get the Full Details

If you're working with model organisms in a teaching lab, the safest approach is to pick genes that are known to be on different chromosomes or sufficiently apart on the same chromosome. Drosophila melanogaster has four chromosome pairs and many well-mapped markers. Pisum sativum, the garden pea Mendel used, has seven chromosome pairs and his seven studied traits happened to fall on different chromosomes or be far enough apart that they behaved independently. Arabidopsis thaliana has five chromosomes and a fully sequenced genome, making it easier to verify gene positions before you set up a cross. If you pick random genes without checking their map positions first, you're gambling with your experimental results. The chi-square test is the standard tool for determining whether your observed ratios deviate significantly from the expected 9:3:3:1 pattern. But remember that chi-square only tells you whether the deviation is statistically significant. It doesn't tell you why. A significant result could mean linkage, it could mean epistasis, it could mean reduced viability of certain genotypes, or it could mean you didn't count your offspring carefully enough. I once saw a student spend two weeks trying to figure out why her chi-square kept rejecting the independent assortment hypothesis before realizing she had misclassified the phenotype of every brown-seeded plant as green because she was colorblind and hadn't accounted for it. The genes were assorting perfectly independently the entire time. When genes are linked, the independent assortment definition biology framework still applies conceptually but the numerical predictions change. You calculate recombination frequency from testcross data and convert it to map units. One percent recombination equals one map unit. Genes more than 50 map units apart essentially behave as if they're unlinked because the recombination frequency maxes out at 50 percent, which is indistinguishable from independent assortment statistically. This is why linkage maps can be unreliable for genes that are far apart on the same chromosome. The observed recombination frequency underestimates the actual physical distance because double crossovers go undetected in a simple two-point cross. You need a three-point cross to catch those events and get an accurate map distance.
For anyone actually doing this work rather than just memorizing it for an exam, the most useful skill is learning to recognize when independent assortment is a reasonable assumption and when it isn't. Look at your data first. If the ratio is close to 9:3:3:1, you can proceed with that assumption. If it's clearly distorted, figure out whether the distortion matches a known pattern like epistasis or linkage before you declare the genes linked. Sometimes the answer is simpler than you think. I've had colleagues dismiss independent assortment entirely because their preliminary data looked messy, only to later discover that contamination in the growth chamber had skewed their counts. A clean re-do with proper controls restored the expected ratio. The bottom line is that independent assortment is a foundational principle that describes what happens when genes are unlinked, but it is not a universal law that applies to every gene pair in every organism. It works when the conditions are right and fails predictably when they aren't. Understanding both the mechanism and its limitations is what separates someone who can pass a genetics midterm from someone who can design a valid experiment.