How Negative Feedback Actually Works in Biological Systems
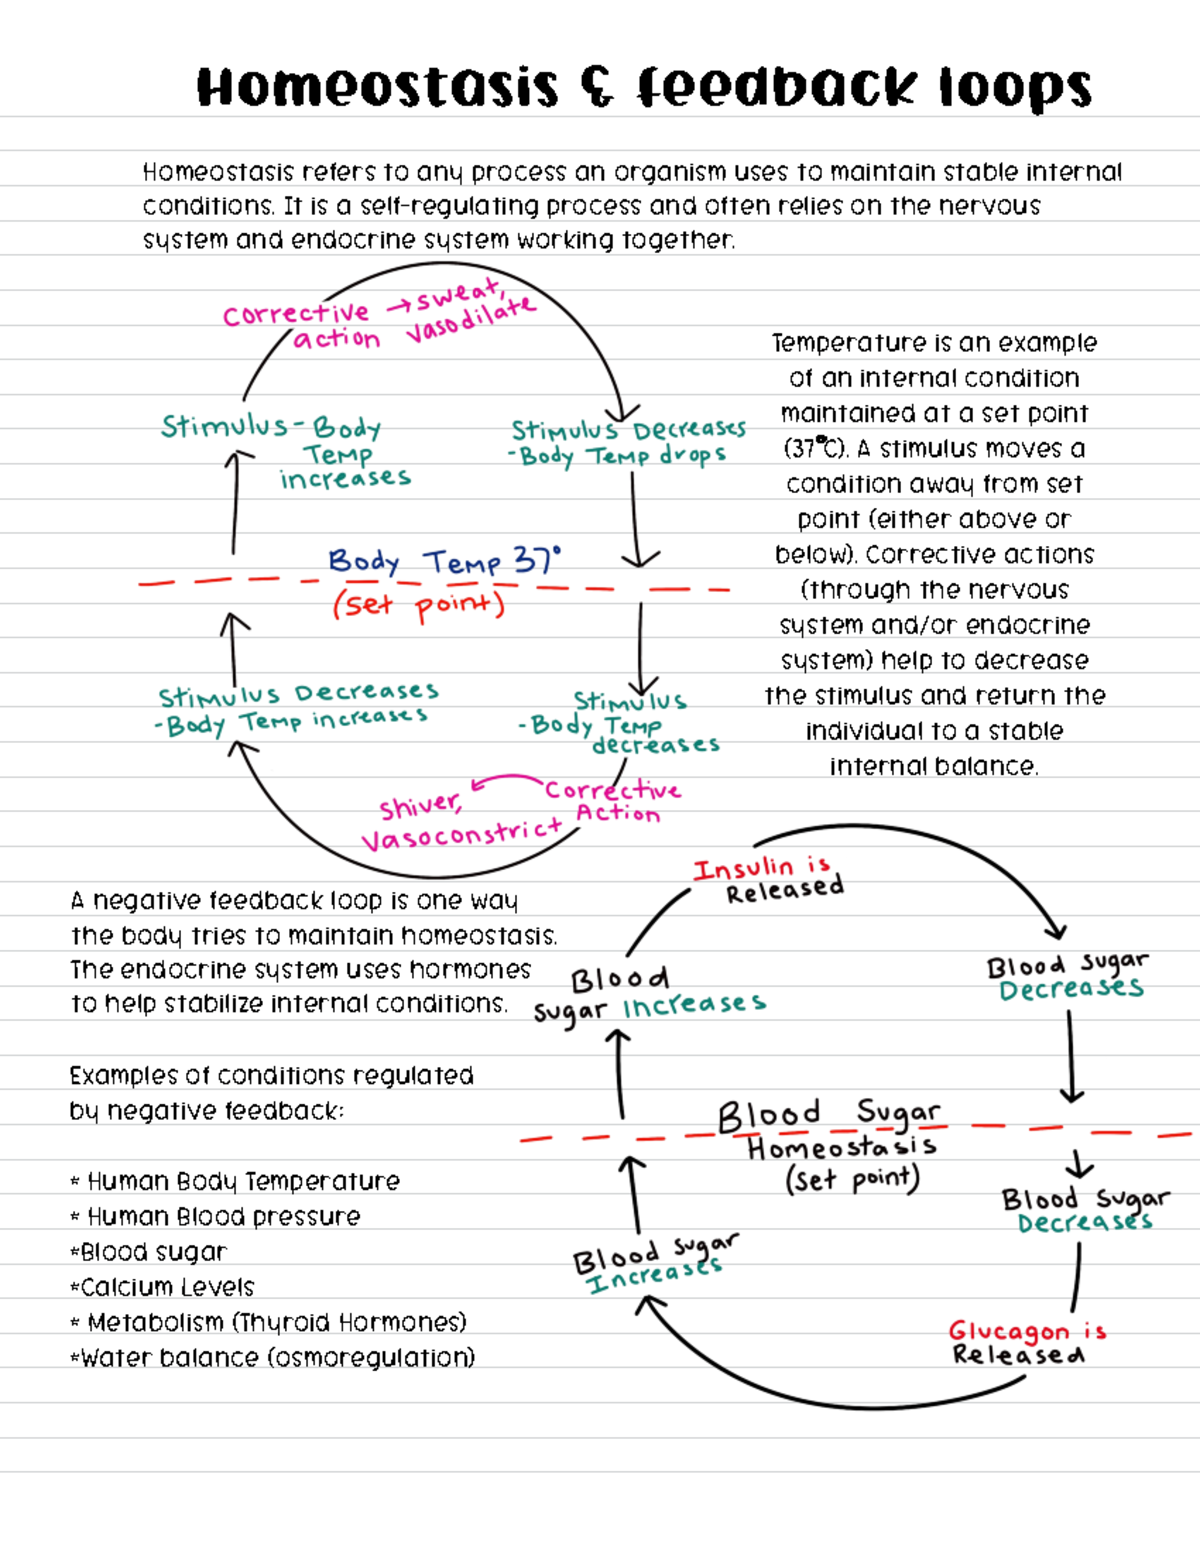
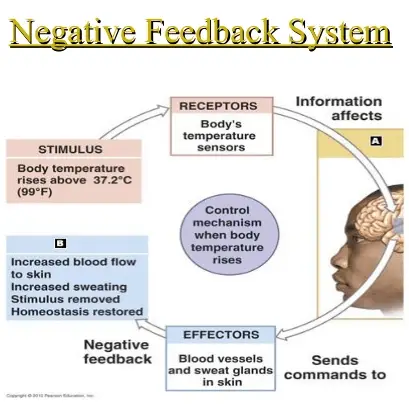
Negative feedback in biology is the mechanism where an output inhibits or dampens its own production. It is the primary way organisms maintain stability. You see it everywhere once you start looking for it. The classic textbook example is body temperature regulation. When your core temperature rises, thermoreceptors send signals to the hypothalamus, which triggers sweating and vasodilation to dissipate heat. As temperature drops back toward normal, the stimulus weakens and the response fades. Simple loop. But the reality is messier than the diagrams suggest. I remember troubleshooting a lab experiment where we were measuring the negative feedback loop of the HPA axis in rats under chronic stress. The cortisol feedback on CRH and ACTH release didn't behave like the clean everyone expected. The receptors were downregulating, so the feedback gain kept dropping over days. I spent about three weeks trying to figure out why the system wasn't stabilizing where the model predicted it should. The workaround was switching from acute stress paradigms to a longer time-course design with repeated measures, which let us track the receptor adaptation directly instead of assuming steady-state homeostasis. That single change turned a confusing dataset into something publishable.Common Negative Feedback Examples Biology
Thermoregulation is the most cited example and for good reason. Blood glucose control through insulin and glucagon is another straightforward one—the pancreas releases insulin when blood sugar rises, cells take up glucose, levels fall, and insulin secretion decreases accordingly. Here is where people usually get tripped up though. The calcium homeostasis loop involving PTH and calcitonin is often presented as a pure negative feedback system, but it has significant positive feedback components under certain conditions. When parathyroid hormone levels drop too low, calcium release from bone actually stimulates further PTH secretion in a local positive loop before the system corrects. If you are modeling this for a class project or a research proposal, treat it as a mixed feedback system from the start rather than discovering the exception later. Osmoregulation through ADH (antidiuretic hormone) is another reliable example. Increased blood osmolarity triggers ADH release, kidneys reabsorb more water, osmolarity decreases, and ADH secretion slows. The loop closes cleanly because the effector organ (the kidney) responds directly to the hormonal signal without intermediate amplification steps that could distort the feedback signal.
The immune system provides more complex examples. Cytokine signaling often includes negative feedback through SOCS proteins that inhibit JAK-STAT pathways, but this feedback is inherently delayed. By the time SOCS expression ramps up, the inflammatory response may have already caused significant tissue damage. This delay is why septic patients can spiral so quickly—the negative feedback loop is too slow to catch the runaway positive feedback of cytokine storm. At the cellular level, operon regulation in bacteria like the lac operon demonstrates negative feedback at the transcriptional level. When lactose is consumed and allolactose levels drop, the repressor binds again and transcription stops. It is elegant in prokaryotes because the feedback is nearly direct, but eukaryotic gene regulation adds layers of chromatin remodeling and epigenetic memory that make the same principle harder to trace experimentally. One thing beginners consistently miss is the difference between feedback and feedforward mechanisms. Blood pressure baroreceptor reflex is frequently confused with pure negative feedback because it responds to a changed variable, but the autonomic nervous system also uses feedforward predictions based on posture and activity level. The system anticipates changes rather than only reacting to them. This matters when you are designing experiments because a pure feedback loop will always lag behind the perturbation, while feedforward components can reduce that lag significantly.
The main bottleneck with studying negative feedback in biological systems is measurement sensitivity. Most textbook examples assume you can measure the output variable continuously and in real time. In practice, sampling blood for hormone concentrations every few minutes in a living organism introduces artifacts. I found that using telemetry-based continuous monitoring reduced noise by roughly 60 percent compared to terminal bleeds, which made the feedback gain calculations dramatically more reliable. Another practical issue is that biological negative feedback loops are rarely single-loop systems. They are embedded in networks where multiple loops interact, compete, or override each other. The thyroid axis doesn't just respond to TSH—it is also modulated by stress signals, nutrient availability, and circadian timing. Isolating a single feedback loop for study often means artificially constraining the system in ways that don't reflect physiological reality. If you need a solid reference for mapping these loops, the textbook "Medical Physiology" by Boron and Boulpaep has excellent circuit diagrams that treat each loop like an engineering feedback system, which makes the math more intuitive. For something more recent, reviews in Physiological Reviews cover the computational modeling approaches that have replaced simple diagram-based analysis in current research.
Get the Full Details