Cellular respiration doesn't care about your syllabus
When you actually sit down and trace the electron flow from glucose all the way to oxygen, the purpose of cellular respiration becomes less of a multiple-choice answer and more of an ugly, interconnected mess. That's normal. Most people learn it backward — they memorize the Krebs cycle as a circle, then try to retrofit meaning onto it. It doesn't work that way in practice. You have to understand what the cell is actually trying to do before any of the steps make sense. The cell is trying to extract usable energy from food molecules. Specifically, it's trying to make ATP, the currency every process in the organism depends on. Glucose has a lot of chemical energy locked in its carbon-hydrogen bonds. The cell can't just tap that energy directly — it would be like trying to run a house on raw crude oil. You need a refinery. That's what the whole respiration apparatus is. It breaks glucose down in controlled steps, captures the released energy in electron carriers, and uses those carriers to drive ATP synthesis.
Understanding the Purpose Of Cellular Respiration
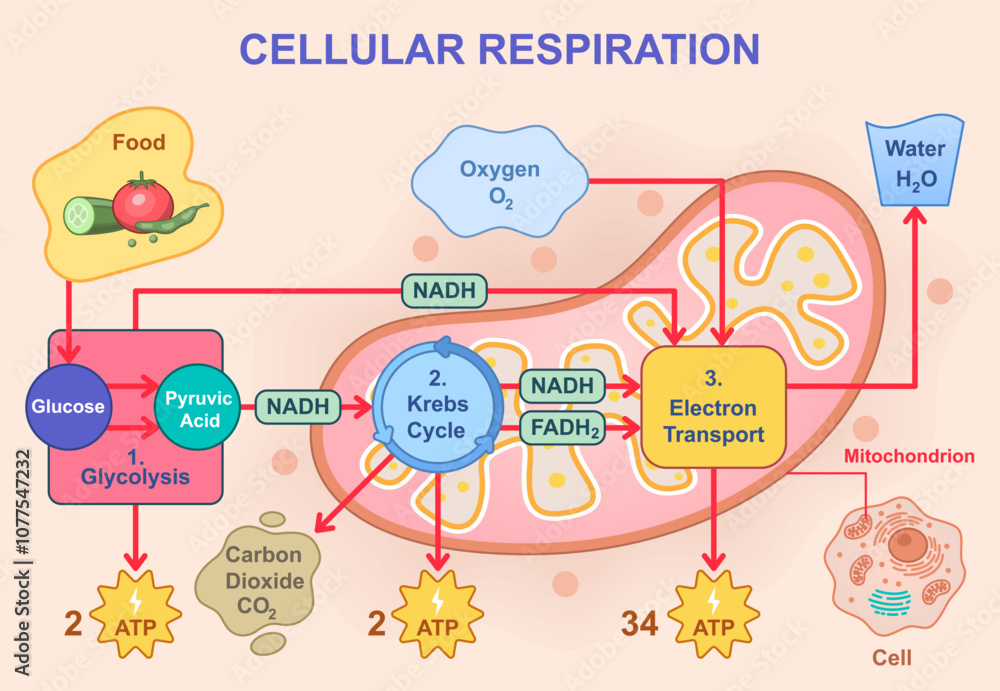
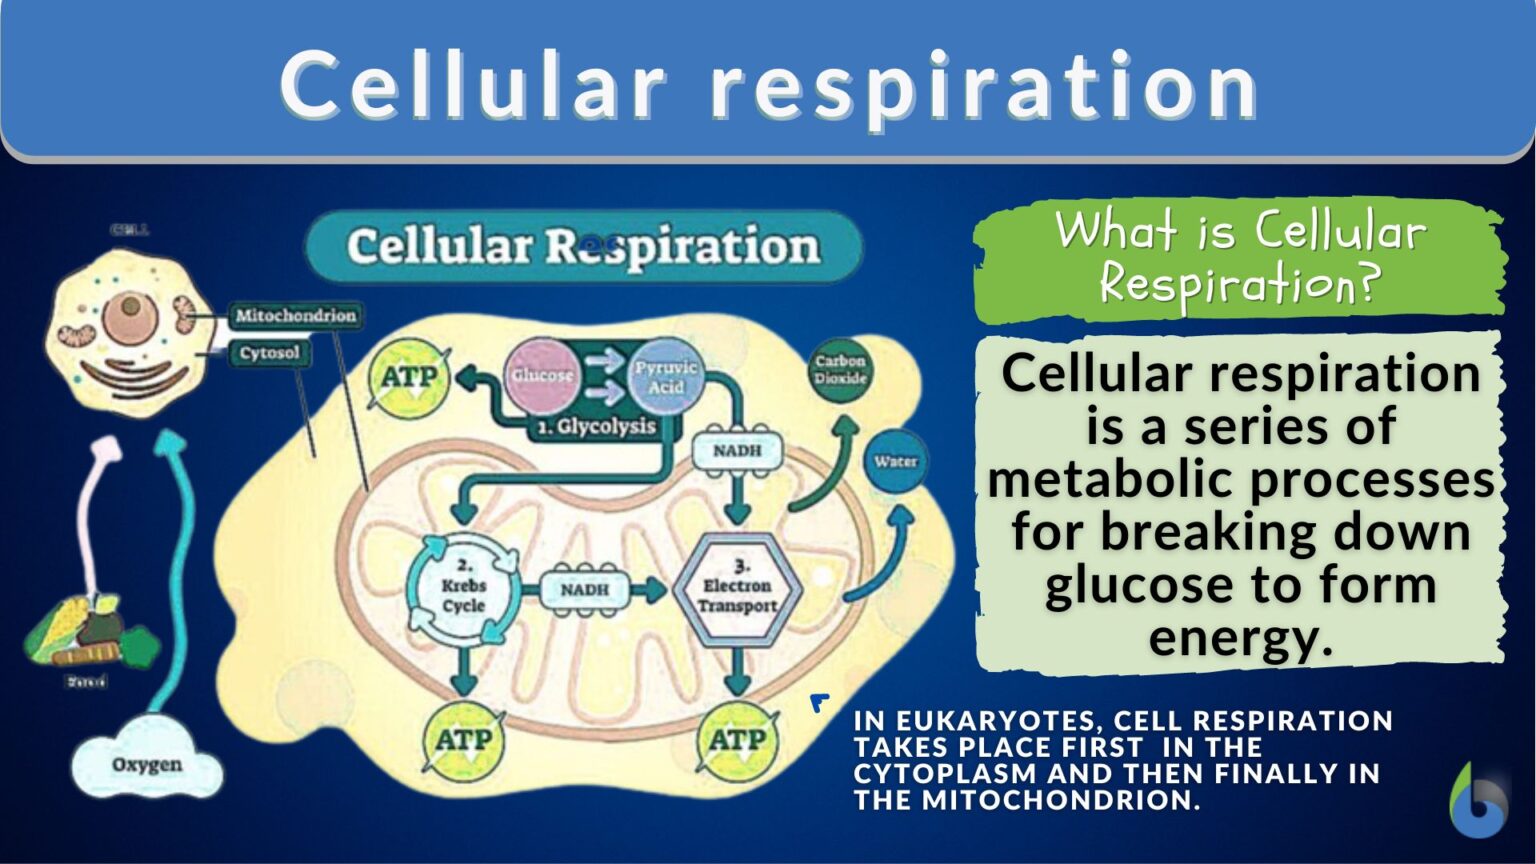
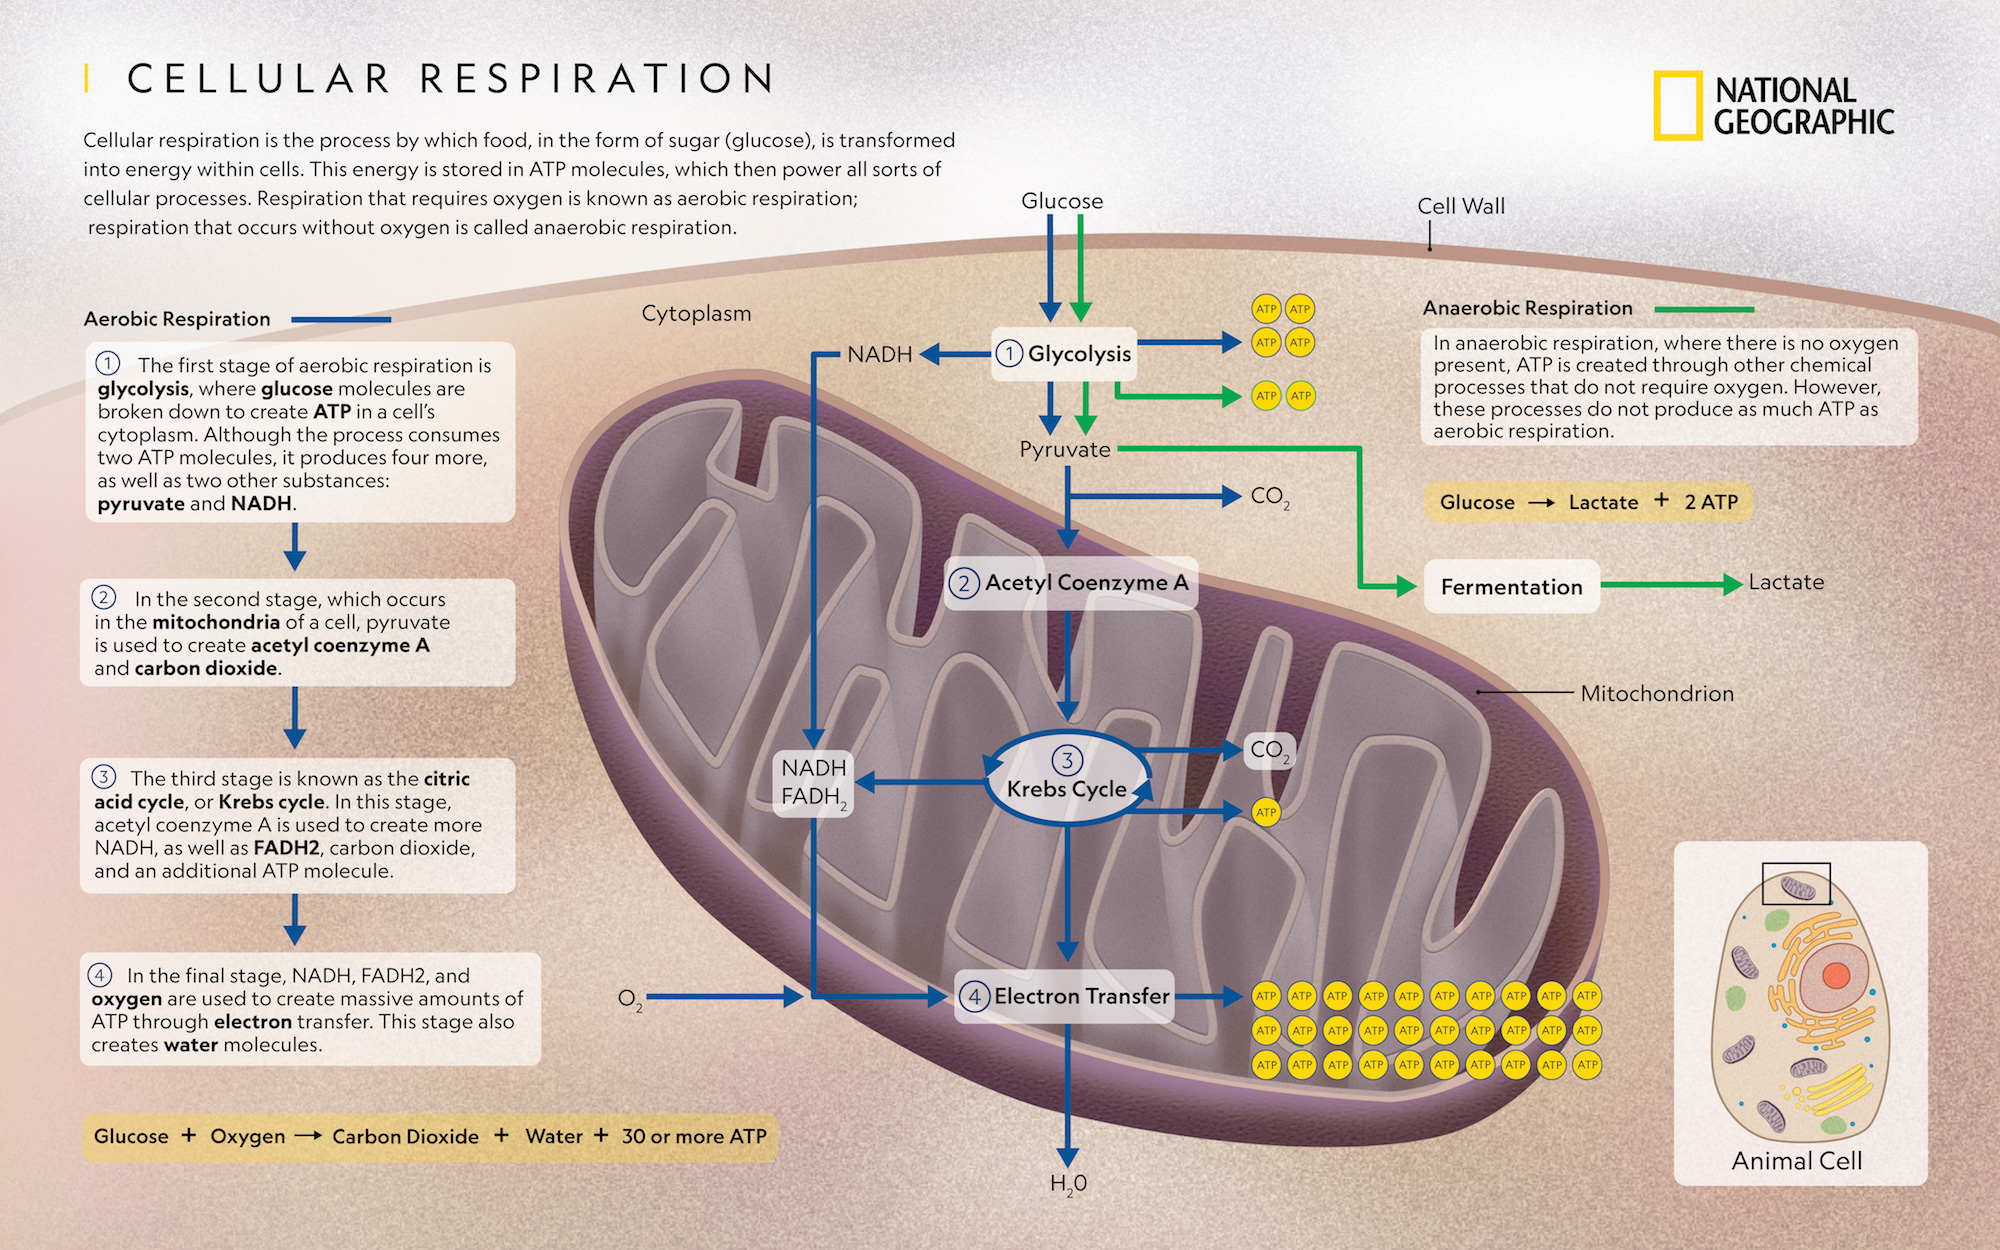
Let me walk you through how it actually works, not how the textbook diagram makes it look. Glycolysis happens in the cytoplasm and splits one glucose molecule into two pyruvate molecules. This stage produces a net gain of two ATP and two NADH molecules. Nothing fancy. It doesn't need oxygen. It's the oldest part of the process evolutionarily, which is why basically every organism on Earth still runs it. The pyruvate then enters the mitochondrion, where things get more complicated. Inside the mitochondrial matrix, pyruvate gets converted to acetyl-CoA. This is the link reaction, and it's where you lose your first carbon as CO2. The NAD+ gets reduced to NADH in the process. Then acetyl-CoA feeds into the Krebs cycle, which turns twice for every original glucose molecule. Each turn produces three NADH, one FADH2, one GTP (which becomes ATP), and two CO2 molecules. The CO2 you breathe out comes from here — mostly. It's not from the oxygen you inhale. That's a common misconception that shows up on exams constantly.
Now here's where the real mechanism kicks in. All those NADH and FADH2 molecules carry high-energy electrons to the electron transport chain embedded in the inner mitochondrial membrane. As electrons pass through complexes I through IV, protons get pumped from the matrix into the intermembrane space. This creates an electrochemical gradient — a proton motive force. ATP synthase uses that gradient to phosphorylate ADP into ATP. Oxygen sits at the end of the chain as the final electron acceptor, combining with electrons and protons to form water. Without oxygen, the whole chain backs up and stops. That's why you can't survive without breathing. I spent a lot of time in undergrad wrestling with this material, and the thing that finally made it click wasn't another diagram. It was realizing that the proton gradient is the actual point. Glycolysis, the link reaction, the Krebs cycle — they're all just setup. They generate the reduced electron carriers. The electron transport chain and chemiosmosis are where the bulk of the ATP comes from. About thirty-four ATP molecules per glucose through oxidative phosphorylation compared to two from glycolysis alone. That's roughly eighty-five percent of your total yield. There's a practical nuance most courses skip. The theoretical maximum yield of cellular respiration is about thirty-six to thirty-eight ATP per glucose molecule, but in real cells you're looking at thirty to thirty-two. Protons leak across the membrane. Some energy gets used for transport processes. The exact yield varies between cell types depending on the shuttle system used to get cytoplasmic NADH into the mitochondrion. The malate-aspartate shuttle is more efficient than the glycerol-3-phosphate shuttle, and different tissues use different ones. Muscle and liver use the malate-aspartate pathway. Brain and heart favor it too. This matters if you're doing anything beyond introductory biology, like interpreting metabolic studies or working with isolated mitochondria.
Get the Full Details

I ran into a specific problem once while troubleshooting an experiment measuring oxygen consumption in isolated rat liver mitochondria. The state 3 respiration rates — that's ADP-stimulated respiration — were way lower than expected for the protein concentration we had. We'd calibrated everything properly. The substrates were fresh. The buffer pH was correct. After about three hours of checking reagents and temperatures, I realized the issue was rotenone contamination in one of our NADH-linked substrate preparations. Rotenone blocks complex I, so NADH couldn't feed electrons into the chain. FADH2-linked substrates like succinate still worked fine, which is why state 3 respiration dropped but didn't disappear entirely. Complex II was still functioning. Switching to a fresh batch of substrate fixed it immediately. The moral is that if your respiration measurements look off, don't blame the mitochondria first. Check your chemicals. Another thing worth understanding is that cellular respiration isn't just about breaking things down. The intermediates serve as precursors for biosynthesis. Citrate from the Krebs cycle gets exported to the cytoplasm for fatty acid synthesis. Alpha-ketoglutarate feeds into amino acid production. Oxaloacetate is a gluconeogenesis precursor. The pathway operates in a cataplerotic direction when the cell needs building blocks more than ATP. This is why fasting and high-carb feeding produce dramatically different metabolic profiles even though the core machinery is the same. Here's a counter-intuitive point that people miss: exercise doesn't primarily increase the number of mitochondria in your cells. It increases their efficiency and changes which fuels they prefer to burn. Mitochondrial biogenesis through PGC-1alpha activation does happen with sustained endurance training, but the acute effects of a single workout are about existing mitochondria working harder and better. The electron transport chain complexes don't multiply overnight. What changes is the coupling efficiency and the expression of specific isoforms of the proteins involved.
There are real limitations to this system. Anaerobic conditions kill oxidative phosphorylation pretty much instantly. The cell falls back on lactic acid fermentation, which regenerates NAD+ but produces no additional ATP beyond glycolysis. That's why prolonged oxygen deprivation causes rapid tissue damage. The brain is especially vulnerable because it relies almost exclusively on aerobic glucose metabolism and has minimal glycogen reserves. Neurons start dying within minutes of severe hypoxia. Cancer cells famously subvert this process through the Warburg effect, preferring aerobic glycolysis over oxidative phosphorylation even when oxygen is plentiful. They do it because the glycolytic intermediates feed into biosynthetic pathways that support rapid proliferation. This isn't a dysfunction — it's an adaptation. When you're trying to divide as fast as possible, having building blocks ready matters more than maximizing ATP yield per glucose molecule. If you're studying this for an exam, focus on the proton gradient as the central concept. Everything else connects to it. If you're actually working with respiratory physiology in a lab, pay attention to your substrates and inhibitors. Complex I inhibitors like rotenone and piericidin A, complex III inhibitors like antimycin A, complex IV inhibitors like cyanide and azide — each one produces a distinct pattern in your measurements that tells you exactly where the blockage is. Knowing what those patterns look like will save you hours of confusion.
The bottom line is that cellular respiration is an energy conversion system optimized for efficiency under aerobic conditions, with significant trade-offs when oxygen becomes limited or when the cell prioritizes biosynthesis over ATP production. It's not elegant. It's not simple. But it works, and understanding the actual mechanism rather than just memorizing the steps is what separates people who can apply this knowledge from people who can only repeat it.