Chloroplasts Are Workhorses, Not Magic
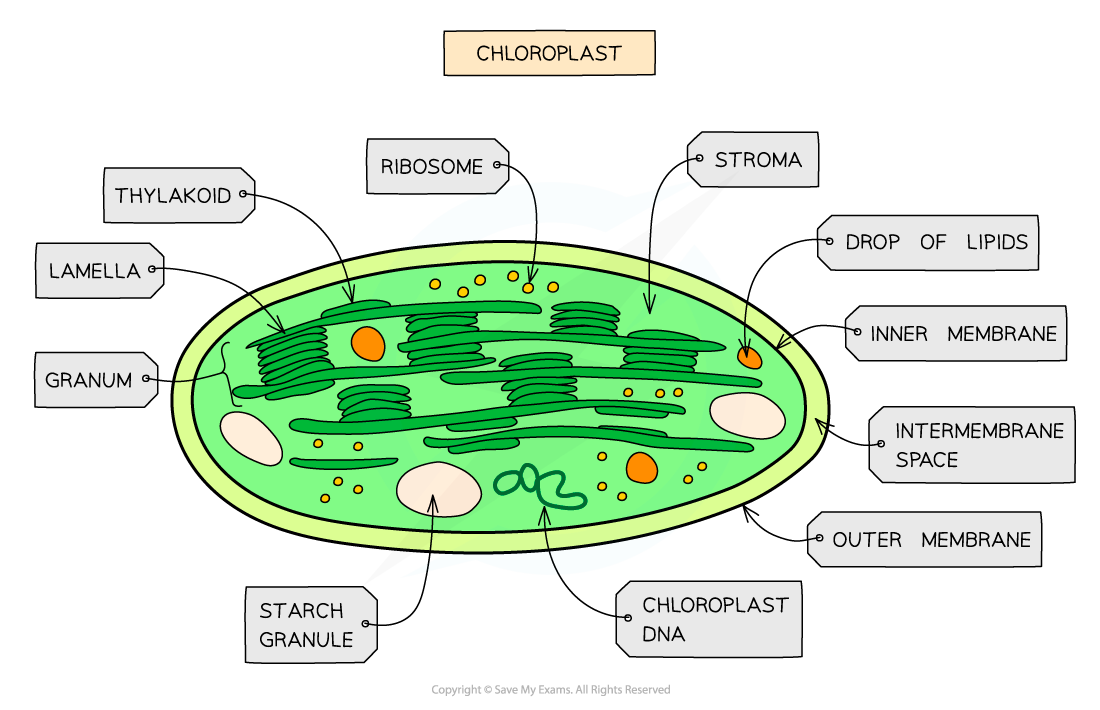
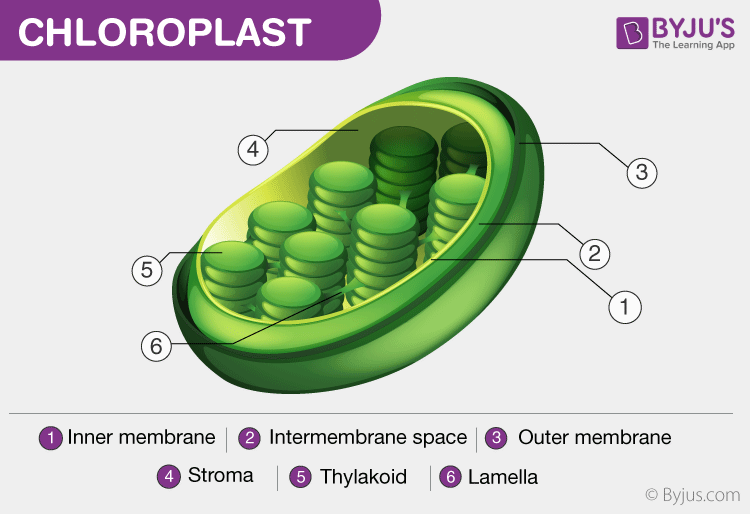
A chloroplast is a double-membrane organelle found in plant and algal cells. Its main job is photosynthesis, which breaks down into two linked stages: the light reactions in the thylakoid membranes and the Calvin cycle in the stroma. The light reactions capture photon energy to split water, pump protons across the thylakoid membrane, and generate ATP plus NADPH. Those two molecules then power the stroma enzymes to fix CO into triose phosphates, which eventually become sucrose or starch depending on what the cell needs at that moment. Most people stop at "makes sugar," but chloroplasts run half the metabolic pathways in a plant cell. They synthesize amino acids like glutamate and aspartate from Calvin cycle intermediates. They produce the isoprenoid precursors via the MEP pathway, which feeds terpenoid and plastochromanol biosynthesis. They house fatty acid elongation enzymes in the stroma. They handle nitrate reduction partially through nitrite reductase. They signal back to the nucleus under stress via retrograde signaling, which is why a chloroplast dysfunction phenotype often looks like a whole-plant problem even when only one organelle is affected. I spent a couple of years running chloroplast isolation protocols for enzyme assays, and the first thing that trips people up is getting clean stroma without thylakoid contamination. If your preparation has intact thylakoids, your Calvin cycle rates will be completely off because everything gets coupled to electron flow. The trick is a gentle homogenization in ice-cold isolation buffer — 0.33 M sorbitol, 50 mM HEPES at pH 7.5, 1 mM EDTA, 2 mM MgCl, and 0.1% BSA — followed by a single low-speed spin at 2,000 × g for 5 minutes to pellet debris, then a second spin at 10,000 × g for 10 minutes to recover the chloroplasts. Never use a higher g-force or you start breaking them open before you want them to. The BSA is not optional, by the way. It binds phenolic compounds released during homogenization that would otherwise inhibit Rubisco irreversibly.
The thylakoid proton gradient is where things get interesting. The pH across the thylakoid membrane can reach 3 full pH units during active illumination, which means roughly a thousand-fold difference in proton concentration between the lumen and stroma. That gradient drives ATP synthase, but it also regulates non-photochemical quenching through the xanthophyll cycle. When the lumen drops below pH 6.2, violaxanthin converts to zeaxanthin and the excess excitation energy dissipates as heat. This is a protective mechanism, not a flaw. Plants that can't switch this on — like certain npq1 mutants in Arabidopsis — photobleach within hours under full sunlight. Here's the part textbooks gloss over: Rubisco isn't just a carboxylase. It's also an oxygenase, and the oxygenation reaction produces phosphoglycolate, which triggers photorespiration. Photorespiration recovers about 75 percent of the carbon from glycolate, but it costs the plant roughly 25 percent of the fixed carbon and additional ATP in the process. C and CAM plants evolved spatial or temporal separation of initial CO fixation from the Calvin cycle precisely to suppress this wasteful pathway. C plants concentrate CO around Rubisco in bundle sheath cells, while CAM plants fix it at night when stomata are open and decarboxylate it during the day. Neither strategy is free — C plants spend extra ATP on the CO pump, and CAM plants have slower growth rates because they can only take in CO at night. One practical limitation nobody warns about: chloroplast genomes don't recombine freely with nuclear DNA the way you'd expect from simple Mendelian genetics. Most chloroplast genes are now in the nucleus — probably after millions of years of endosymbiotic gene transfer. In angiosperms, chloroplasts are usually inherited maternally, which means transgene containment strategies based on chloroplast transformation are one of the few ways to achieve biological containment for genetically modified crops. Pollen-borne transgenes won't spread through the chloroplast route. That said, chloroplast transformation efficiency varies enormously between species. Tobacco and lettuce take to it easily. Most crops still resist it, and getting stable homologous recombination into the chloroplast genome requires a lot of optimization.
If you're trying to measure actual photosynthetic rates rather than just guessing from leaf color, a gas exchange system that tracks O evolution and CO uptake simultaneously is the standard approach. Pulse-amplitude modulation fluorometry gives you the effective quantum yield of PSII in real time, which is useful for diagnosing photoinhibition before visible damage appears. The downside is that both methods require steady-state conditions and careful temperature control. Leaf temperature alone can shift the Rubisco specificity factor enough to change the carboxylation-to-oxygenation ratio noticeably. Chloroplasts also accumulate starch transiently during the day and degrade it at night to sustain growth when light isn't available. The starch turnover rate matters — mutants that can't degrade starch properly grow stunted even though their photosynthetic capacity is normal. The circadian clock pre-adjusts starch degradation enzymes before dusk so the reserve lasts exactly through the night. If the timing is off, the plant either runs out of carbon before dawn or wastes potential biomass storing excess starch. For anyone setting up chloroplast experiments and wondering why their yields are lower than expected, the biggest factor is usually leaf age and growth conditions. Mature, fully expanded leaves give the best preparations. Younger leaves have proportionally fewer chloroplasts and more amyloplasts cluttering the isolation. Plants grown under low light produce larger chloroplasts with more grana stacks but lower Rubisco content per unit volume. High light does the opposite. Adjust your buffer volumes and spin times accordingly — a preparation optimized for shade-adapted leaves will shear sun-adapted ones.
Get the Full Details