Coenzymes Explained Like You're Actually Sitting Across From Me At A Bench
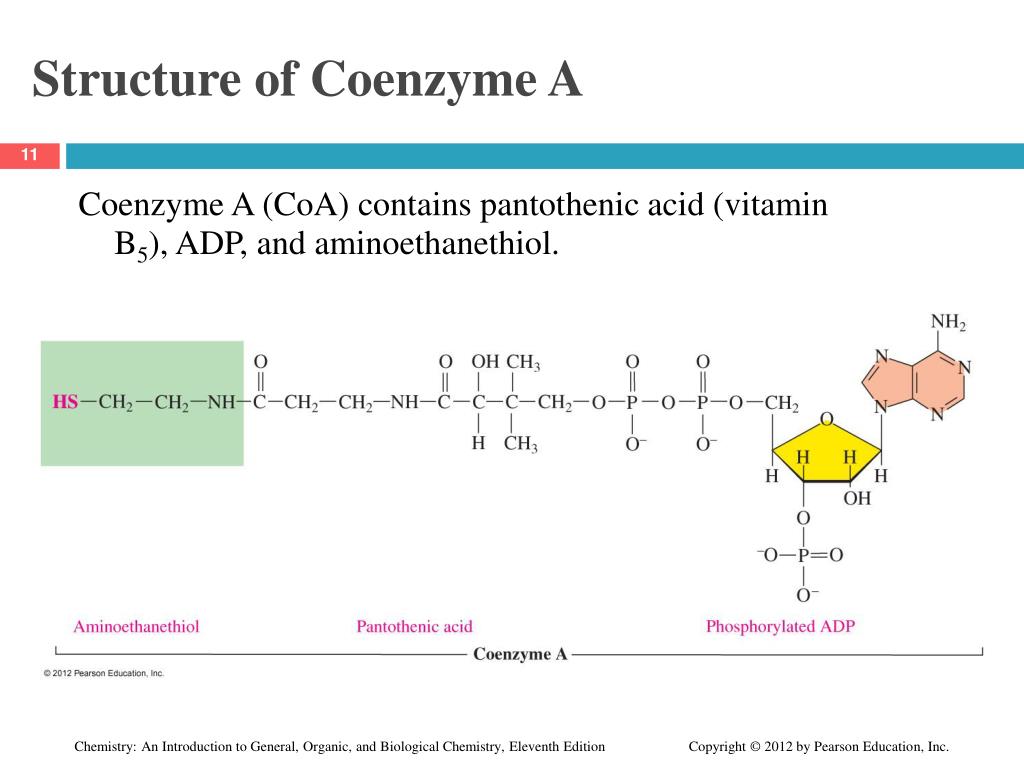
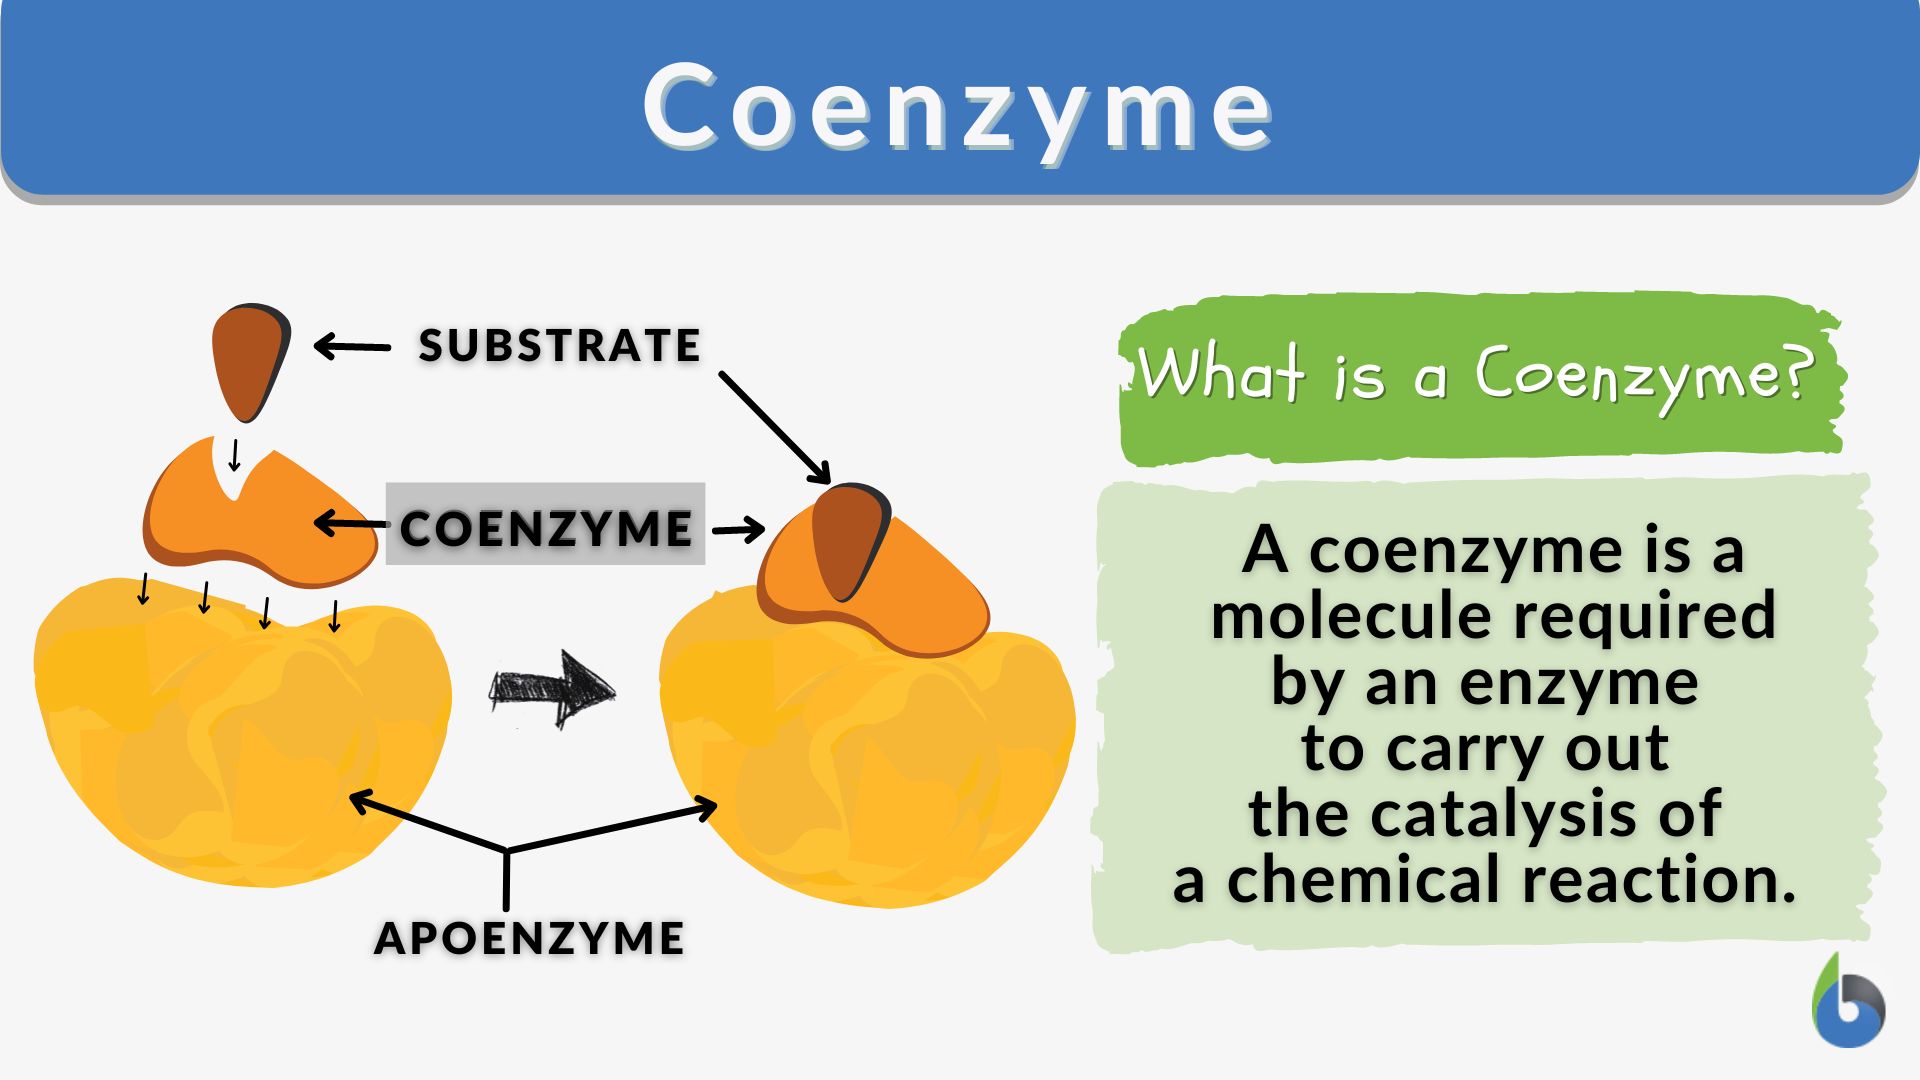
You grab a vial of cofactor from the shelf, add it to your reaction mix, and then watch the spectrophotometer flatline for forty-five minutes while your sample degrades. This is where the rubber meets the road with coenzymes. They are not magic. They do not perform miracles on their own. They are small organic molecules that shunt electrons, atoms, or functional groups between enzymes during catalysis, and they get consumed in the process. That last part is what trips most people up. You can think of them as the refillable fuel cartridges for enzymes, which is why cells constantly recycle them through companion pathways. In practical terms, What Is A Coenzyme becomes obvious once you stop treating it like a vocabulary word and start thinking about it as a consumable reagent that needs its own supply chain. I ran into a specific problem last year that cost me about three days of work before I figured out what was going on. I was running a lactate dehydrogenase assay using NAD+ as the coenzyme, and the reaction kinetics looked weird at concentrations below fifty micromolar substrate. The velocity dropped faster than the Michaelis-Menten curve predicted, even though everything else was right. Turns out the NAD+ stock had partially degraded from repeated freeze-thaw cycling, and the free nicotinamide ring was oxidizing into an inactive form that still absorbed at 260 nanometers but catalyzed nothing. The absorbance readout fooled me into thinking I still had plenty of active coenzyme. I had to run an HPLC check on the stock, separate the intact NAD+ from the degraded fragments, and recalculate the actual active concentration before the data made any sense. That is the kind of thing nobody tells you in undergrad biochem. The common pitfall is assuming that nominal concentration equals functional concentration. Coenzymes degrade. NAD+ loses activity on exposure to light and repeated temperature cycling. FAD can photobleach in the cuvette. Thiamine pyrophosphate hydrolyzes at neutral pH over time. If you are doing quantitative enzyme kinetics and your Km or Vmax values shift between prep batches, check the coenzyme first before you blame the enzyme.
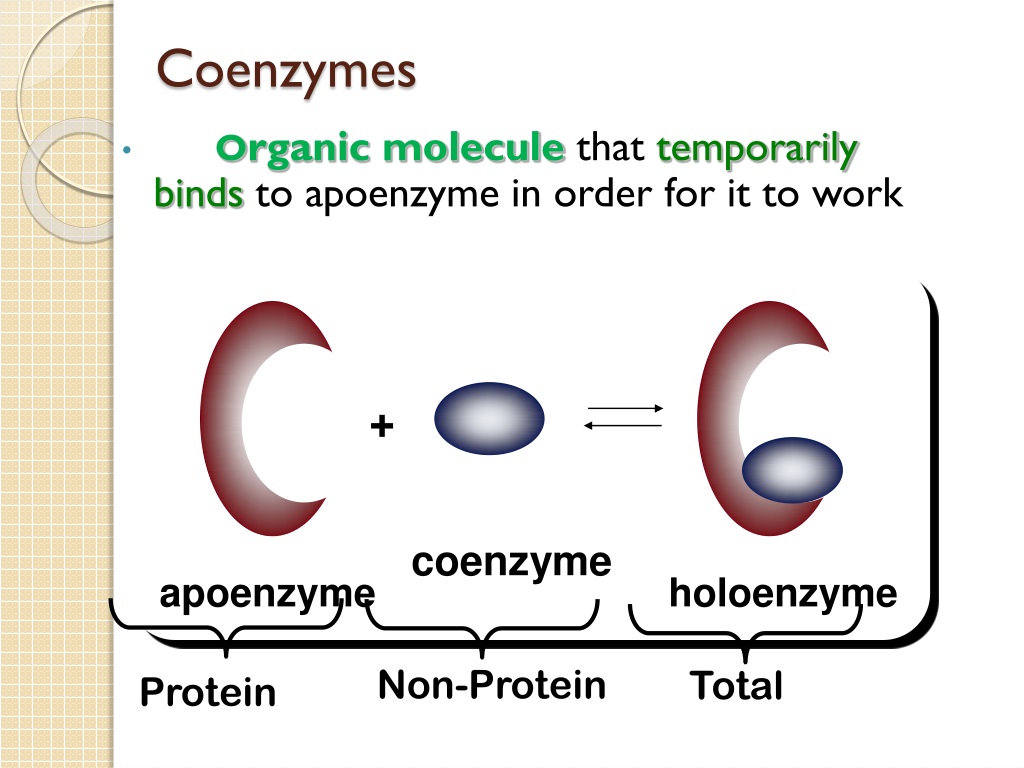
Another counter-intuitive point: coenzymes are not always required. Some enzymes function perfectly well without any organic cofactor. Carbonic anhydrase works fine with just a zinc ion and water. The distinction matters because when someone says a reaction needs a cofactor, you need to know whether they mean a metal ion, a prosthetic group, or a true coenzyme that dissociates after each catalytic cycle. Prosthetic groups like heme in cytochrome c stay bound. True coenzymes like NADH come and go. This distinction changes how you handle purification, storage, and assay design. From a practical standpoint, here is how I approach coenzyme-dependent work now. I aliquot everything on first arrival. I store NAD+ and NADP+ at minus eighty degrees, never touch them after thawing. I make working solutions fresh weekly in dark tubes because UV light degrades the nicotinamide ring. I verify activity with a standard assay before committing a full experimental run. For FAD-dependent enzymes, I protect from light more aggressively and use anaerobic conditions when possible because the reduced flavin form oxidizes rapidly in air. The turnover number for most coenzymes is high, but the specific activity drops noticeably after two weeks in solution even at four degrees Celsius, so I do not trust stocks older than that for precise work. The downside of relying on exogenous coenzymes in vitro is that they introduce a second variable into every experiment. You are no longer measuring just enzyme activity. You are measuring enzyme activity conditional on coenzyme integrity, concentration, and regeneration capacity. In cell-free systems this is manageable. In vivo it is a whole different problem because the cell has to balance coenzyme pools across multiple pathways simultaneously. The NAD+/NADH ratio, for instance, is not just a label for redox state. It is a regulatory signal that shifts with metabolic flux, and perturbations in coenzyme availability can change gene expression independently of any enzymatic defect you are trying to study. I learned that the hard way when my apparent enzyme inhibition turned out to be coenzyme depletion from an unexpected side reaction in the buffer.
If you need a cheaper alternative to purchasing pure coenzymes for large-scale work, some labs regenerate them in situ. Glucose dehydrogenase can recycle NADH continuously from glucose. Pyruvate dehydrogenase couples NAD+ reduction to pyruvate conversion. These systems cut coenzyme costs by roughly ninety percent and keep concentrations stable over hours rather than minutes, but they add complexity and potential interference from the recycling enzymes themselves. Worth it for preparative work, less worth it if you are doing mechanistic studies where extra proteins muddy the interpretation.
Get the Full Details