Oxygen in the Lab versus Oxygen in the Body
You run a respiration assay and the numbers look wrong. The probe reads 8 mg/L dissolved oxygen, but the culture is clearly starving. This happens more often than you would expect, and it has nothing to do with your math. It is about understanding what O2 actually does at the molecular level, and where the easy explanations fall apart. I spent three years troubleshooting exactly this problem in a plant physiology lab before I stopped blaming the electrode and started looking at the media composition. At its core, O2 is a terminal electron acceptor in aerobic respiration. Electrons travel through the electron transport chain embedded in the inner mitochondrial membrane, and molecular oxygen sits at the end of that line, accepting electrons and protons to form water. That reaction drives proton pumping, which builds the electrochemical gradient that ATP synthase uses to make adenosine triphosphate. Without that final acceptor, the chain backs up, proton pumping stops, and ATP production drops to near zero within seconds. The chemistry is straightforward. The standard reduction potential for the O2/H2O couple is +0.82 volts, which makes it one of the most powerful biological oxidants available under physiological conditions. That high potential is exactly why your cells bother with it instead of using something simpler like sulfate or carbonate. The tradeoff is that the same reactivity that makes O2 useful also makes it dangerous.
Reactive Oxygen Species Are Not an Accident
Electron leakage from complexes I and III generates superoxide radicals even under normal aerobic conditions. Superoxide dismutase converts it to hydrogen peroxide, catalase and glutathione peroxidase then reduce that to water. The system works most of the time, but it is not perfect. When the proton motive force gets too high, or when NADH accumulates faster than the TCA cycle can process it, electron leakage spikes and ROS production follows. This is why you see oxidative damage in cultures that are overgrown or starved of nutrients, even though they have plenty of oxygen. A counterintuitive point that many textbooks skip is that higher oxygen tension does not always mean higher respiration rates. In mammalian cell culture, for example, pushing dissolved oxygen above 60 mmHg often suppresses proliferation because the resulting oxidative stress triggers cell cycle arrest. The cells are not dying from hypoxia; they are slowing down because the redox balance is off. I ran into this when I switched from 21 percent atmospheric oxygen to a 30 percent headspace setup expecting faster growth, and instead got slower, more senescent populations. Dialing the oxygen back to 5 percent actually improved the data.
Molecular Transport Mechanisms Vary by Organism
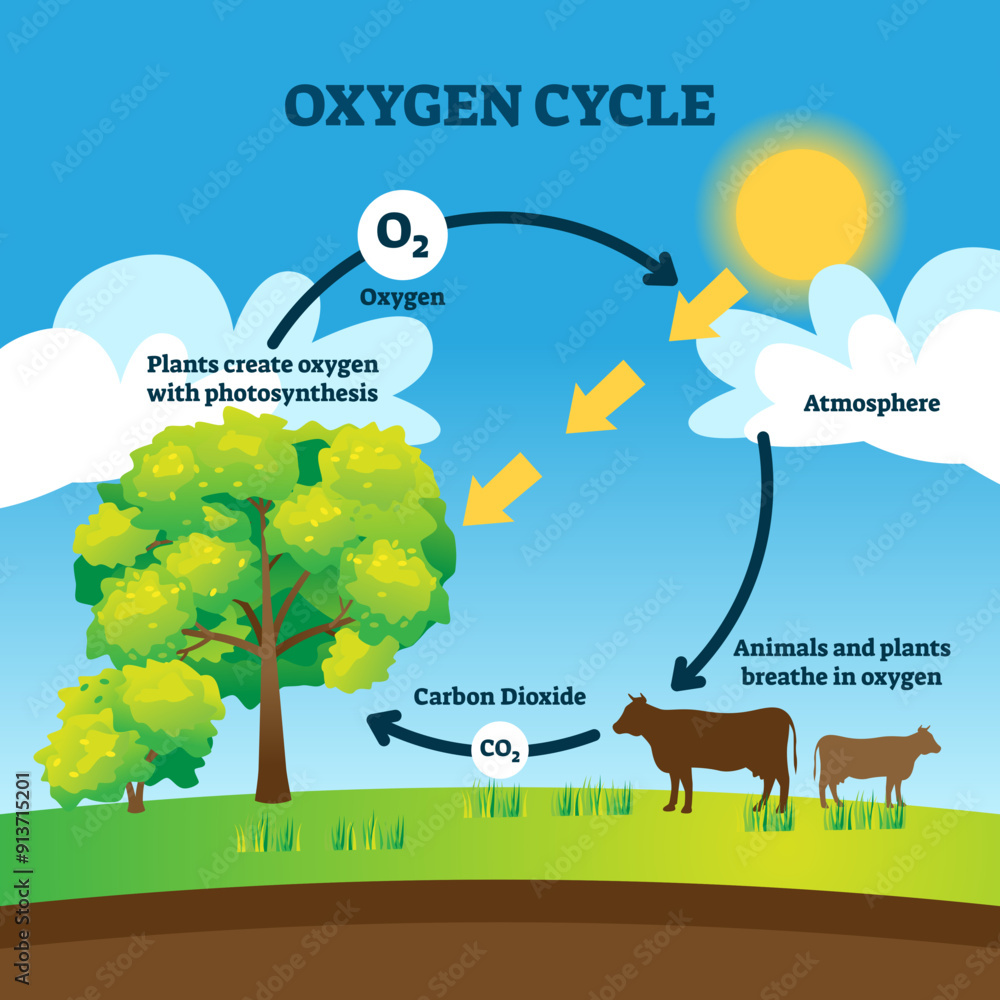
Diffusion alone handles oxygen transport in small organisms and thin tissues because the distance is short enough that Fick's law keeps up with metabolic demand. A single-celled organism does not need hemoglobin. A flatworm does not need lungs. The diffusion limit works until you exceed a certain thickness, and then you need a circulatory system or respiratory pigment to move O2 faster than diffusion allows. Hemoglobin and hemocyanin solve this by binding O2 cooperatively, which gives you the sigmoidal saturation curve that lets the molecule load efficiently in the lungs or gills and unload efficiently in the tissues. The P50 value, the partial pressure at which the protein is 50 percent saturated, shifts depending on pH, temperature, and allosteric effectors like CO2 and 2,3-BPG in vertebrates. That Bohr effect is not a minor detail. It means that metabolically active tissues, which produce acid and heat, actually get more oxygen released from hemoglobin right where it is needed most. In plants, the picture is different because photosynthesis and respiration happen in the same organs. Chloroplasts produce O2 during the light-dependent reactions by splitting water at photosystem II. Mitochondria consume it during photorespiration and dark respiration. The net gas exchange depends on light intensity, temperature, and CO2 concentration. At low light, plants are net consumers of oxygen. At high light, they become net producers. The compensation point where photosynthetic O2 evolution exactly balances respiratory O2 consumption is usually around 200 to 500 ppm CO2 depending on the species.
Get the Full Details

Altitude and Adaptation
At 3000 meters the atmospheric partial pressure of oxygen drops to about 150 mmHg compared with 160 mmHg at sea level. The difference sounds small, but it matters for VO2 max and aerobic performance. The immediate response is hyperventilation driven by peripheral chemoreceptors in the carotid bodies. Over days and weeks, erythropoietin increases red blood cell production, and mitochondrial density can shift in skeletal muscle. These are standard adaptations, but they have limits. High-altitude pulmonary edema and high-altitude cerebral edema occur when the normal compensatory responses overshoot. The exact mechanisms involve hypoxic vasoconstriction, increased capillary pressure, and endothelial leakage, but the practical takeaway is that supplemental oxygen or graded ascent works better than pushing through symptoms. I had a colleague who ignored mild headache and insomnia during a field season at 4200 meters, assuming it was normal acclimatization. He ended up with HAPE and needed evacuation. The headache is your body telling you something is wrong, not a rite of passage.
Measuring Oxygen Correctly
Winkler titration remains the reference method for dissolved oxygen, even though it is slow and requires careful handling of manganese sulfate and alkaline iodide. Clark-type electrodes are faster but drift over time and need regular calibration. Optical sensors using ruthenium or palladium porphyrin fluorophores are more stable and do not consume oxygen during measurement, which makes them better for microaerobic experiments. If you are working with low oxygen tensions, electrode consumption can artificially lower the reading in a closed chamber. The common pitfall is ignoring temperature compensation. Oxygen solubility changes by roughly 2 percent per degree Celsius. A reading taken at 25 degrees Celsius without correction will be systematically wrong if you compare it to a value measured at 20 degrees. Always record temperature and apply the solubility correction, or use a sensor with built-in compensation. Another frequent error is stirring too vigorously during membrane permeability experiments. Agitation can create local hypoxic zones around the sample surface, which distorts the apparent permeability coefficient. Gentle swirling is usually sufficient, and you should verify that your stirring speed does not affect the measured rate constant.
When Oxygen Limits Biotechnology Processes
Bioreactor scale-up is almost always an oxygen transfer problem. The volumetric mass transfer coefficient, kLa, determines how much oxygen you can deliver to the culture per unit time. As volume increases, the surface-area-to-volume ratio decreases, and sparging becomes less efficient. You compensate by increasing agitation speed, enriching the headspace with oxygen, or using pure oxygen instead of air. Each option has costs and risks. Higher agitation creates shear stress that can damage animal cells. Pure oxygen increases the risk of fire and explosion in sealed systems. Enriched air is the safest compromise for most bacterial fermentations. I once watched a $12,000 fermentation run fail because someone forgot to check the oxygen sparge line for condensation buildup. The line looked fine visually, but liquid had pooled in the tubing and blocked gas flow entirely. The biomass yield was half of what the model predicted, and the only clue was the dissolved oxygen trace holding steady at near-zero after two hours. Installing a pressure gauge on the sparge line and checking it every hour prevented this from happening again.
Oxygen in Anaerobic Environments
Anaerobic organisms lack the enzymes to detoxify reactive oxygen species, which is why trace oxygen is lethal to many strict anaerobes. Clostridium species, for example, carry only minimal superoxide dismutase and catalase activity. Even micromolar oxygen levels generate enough superoxide to damage iron-sulfur clusters in key metabolic enzymes. This is why anaerobic work requires rigorous deoxygenation of media and strictly inert atmospheres. Facultative anaerobes like Escherichia coli switch between respiration and fermentation depending on oxygen availability. Under aerobic conditions, they perform complete oxidation of glucose through the TCA cycle and electron transport chain. Under anaerobic conditions, they ferment pyruvate to mixed acids. The switch is regulated by the Fnr and ArcAB systems, which sense oxygen through iron-sulfur cluster chemistry. This regulatory logic is elegant, but it means that anaerobic cultures of E. coli produce very different metabolite profiles than aerobic ones, and you cannot simply subtract the difference.
Photosynthetic Oxygen Evolution
The oxygen-evolving complex in photosystem II is a manganese-calcium cluster that extracts electrons from water through a four-step S-state cycle. Each photon absorbed advances the cycle by one state, and after four photons, molecular oxygen is released and four protons are deposited into the thylakoid lumen. The OEC is one of the most challenging enzymatic systems to study structurally because it is sensitive to X-ray damage and requires cryo-preservation for high-resolution diffraction. Halogen substitution at the OEC is a real phenomenon in some marine algae and cyanobacteria, where chloride and bromide ions participate directly in the catalytic mechanism. Removing chloride from the buffer inhibits oxygen evolution within minutes. If you are doing in vitro PSII experiments and the activity drops unexpectedly, check the chloride concentration in your extraction buffer before assuming the sample is degraded.
Practical Takeaways
Oxygen is not just a background condition in biology. It is a reactant, a regulatory signal, a source of damage, and a limiting factor in culture systems. The relationships are nonlinear and context-dependent. A protocol that works at 21 percent oxygen may fail at 5 percent, not because the cells are hypoxic, but because the oxidative signaling environment changed enough to alter gene expression. If your experimental results do not match the literature, checking the oxygen conditions first is usually worth more than re-running the entire assay on a hunch. The tools available for measuring and controlling oxygen have improved significantly in the last decade, but they still require careful calibration and an understanding of what the readings actually represent. Dissolved oxygen in milligrams per liter is not the same as percent saturation. Percent saturation depends on temperature and salinity. Partial pressure in millimeters of mercury is the physiologically relevant quantity for gas exchange calculations. Converting between these units is straightforward, but the conversions are often skipped in methods sections, which makes reproducibility harder than it needs to be.