The Pressure Inside a Plant Cell
Water potential is one of those concepts that sounds simple until you try to use it in the lab. The textbook definition says it is the potential energy of water per unit volume relative to pure water, measured in megapascals. That is accurate. It is also not enough. I spent three years working with plant physiology and measuring water relations in seedlings. The first time I tried to calculate osmotic potential from a pressure probe, my numbers were completely wrong. Not slightly off. Wrong. The problem was not the math. It was the assumption that a leaf cell is in equilibrium at the moment you puncture it. It is not. The cell leaks, pressure drops, and the reading you record is a fraction of what the water was actually doing before the probe touched it.
What Is Water Potential In Biology
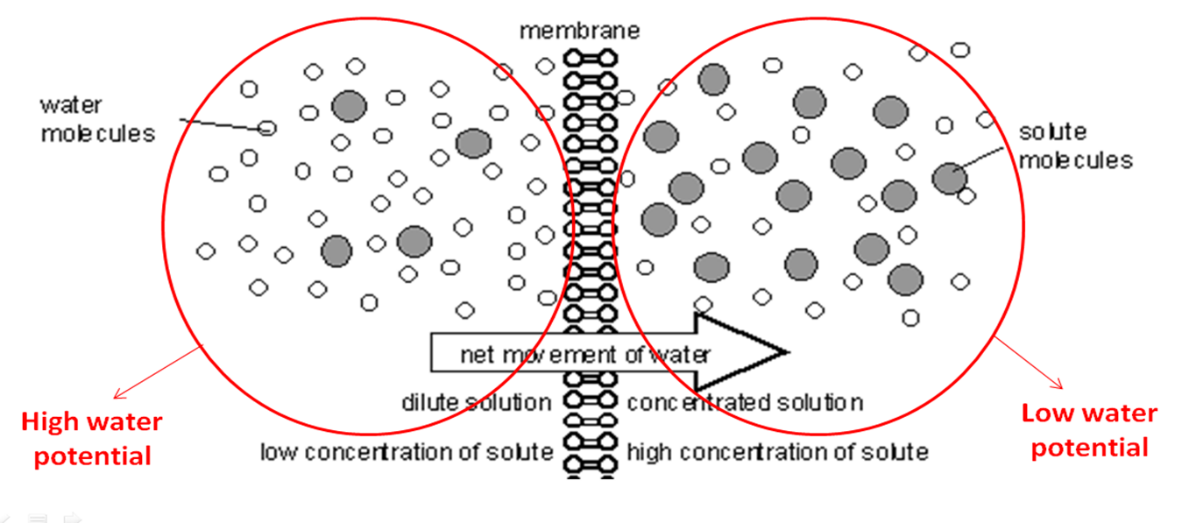
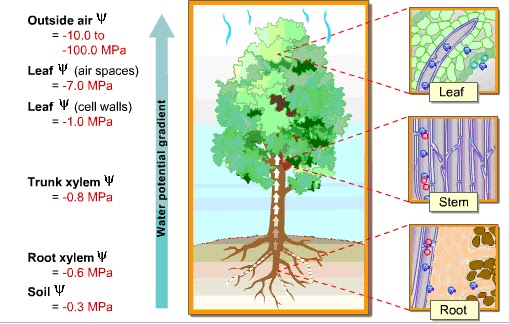
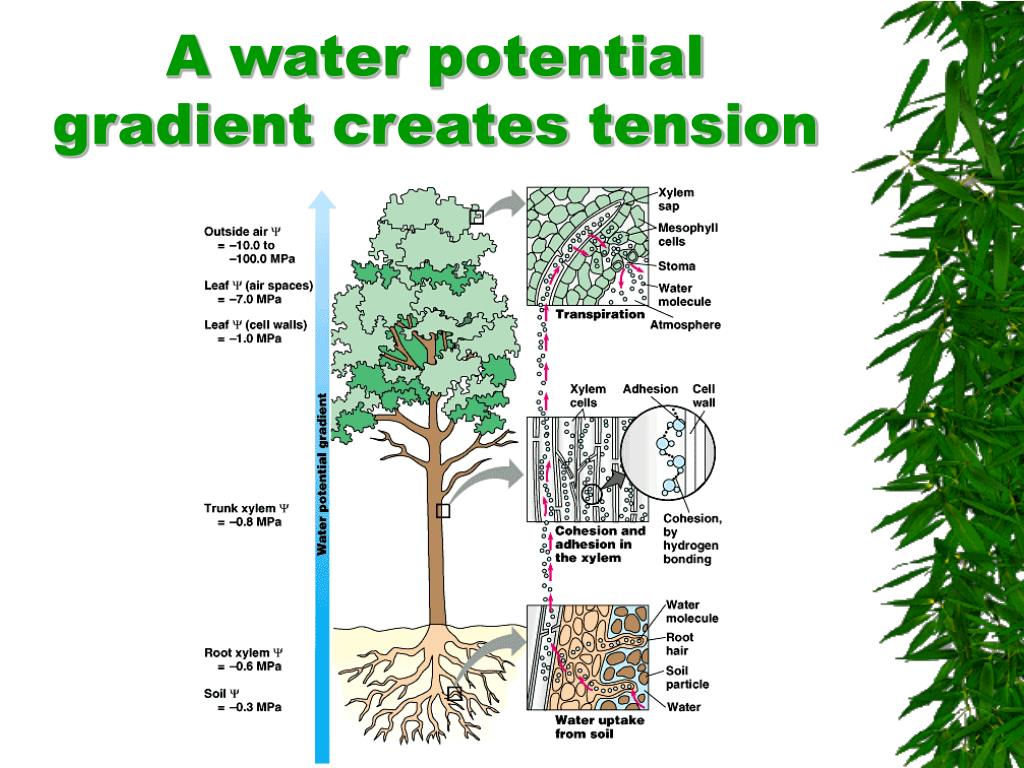
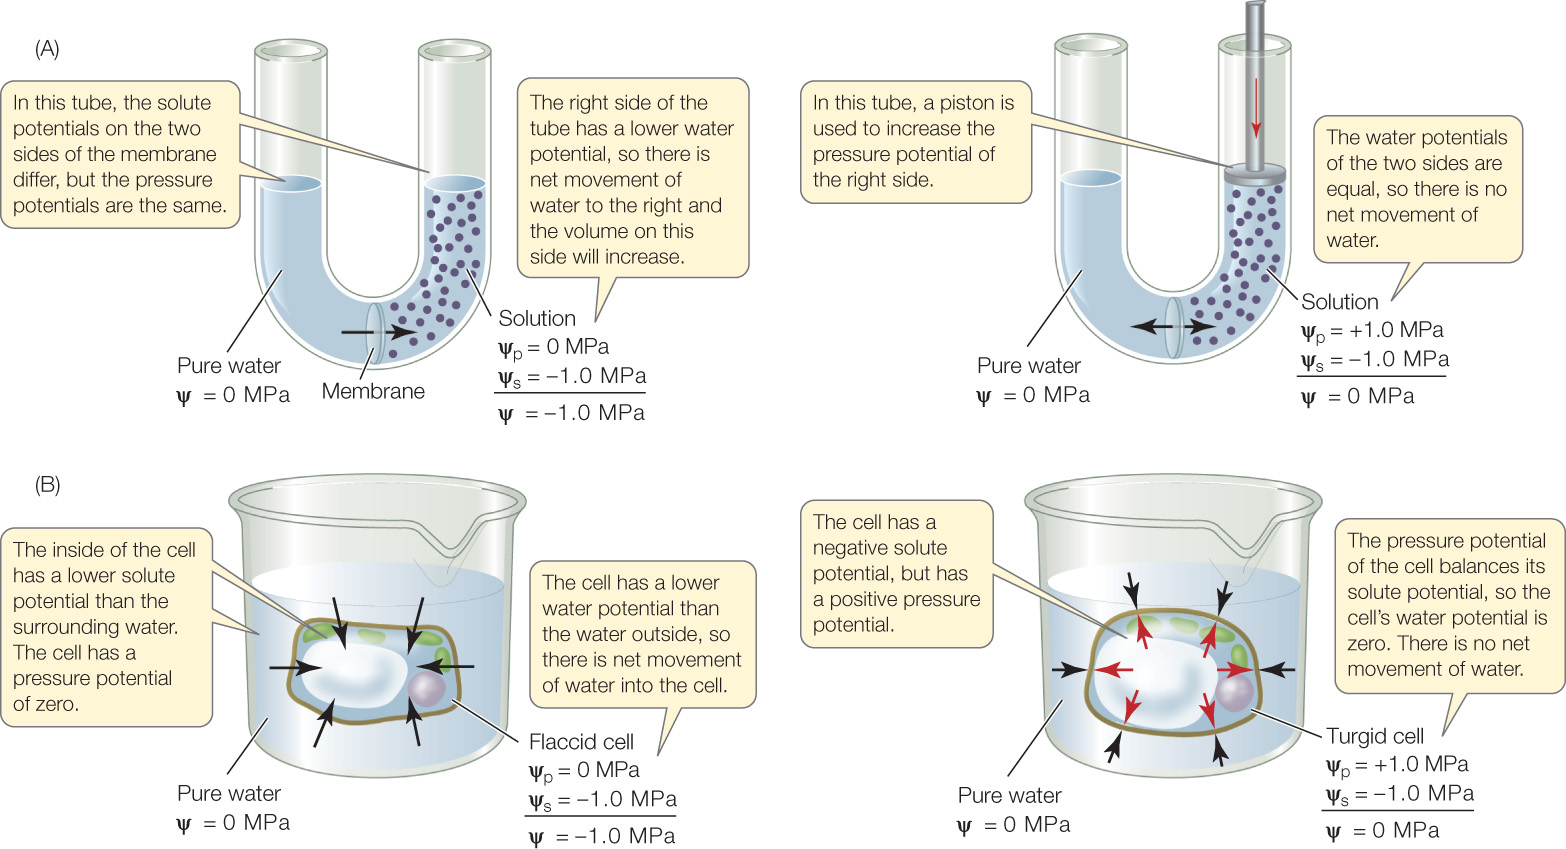
At the core of it, water potential tells you the direction water will move. Water always moves from a region of higher water potential to a region of lower water potential. Pure water at sea level and room temperature has a water potential of zero by definition. Anything with solutes in it has a negative value. Freezing point depression, matric forces in soil, and pressure inside a turgid cell all shift that value around. The equation is Psi equals Psi os plus Psi p plus Psi m plus Psi g. Most introductory courses drop the gravity term because it matters only when you are dealing with tall trees or elevation differences. In a potted plant on a bench, gravity is irrelevant. In a 30-meter pine, it is the difference between the top needles wilting and the roots pulling hard enough to sustain them. I have seen students ignore Psi g and then wonder why their model of water transport in conifers predicted impossible flow rates. Osmotic potential, Psi os, comes from dissolved solutes. Sugar, salts, ions. The more solutes, the more negative the value. A typical mesophyll cell might sit around minus 0.8 to minus 1.2 megapascals depending on species and environmental conditions. Salt stress pushes that deeper into negative territory. That is why saline soils damage plants so quickly. The root cells cannot maintain a gradient steep enough to pull water in against the external osmotic pressure.
Pressure potential, Psi p, is the physical push or pull on the water. In a flaccid cell it is zero. In a turgid cell it is positive, usually around plus 0.5 to plus 1.0 megapascals for most herbaceous plants. Xylem under tension has a negative pressure potential. That is the controversial part. The cohesion-tension theory relies on water being pulled rather than pushed, and negative pressure in xylem is physically stable because water molecules stick to each other through hydrogen bonding. But if an embolism forms, the whole column can snap. I have seen entire branches die from a single cavitation event during a drought pulse. The rest of the tree keeps functioning, but that branch is dead wood.
Get the Full Details

Measuring It Without Losing Your Mind
The Scholander pressure chamber is the standard tool. You clip a leaf in, apply nitrogen pressure until sap appears at the cut stem surface, and the pressure you read is the absolute value of the xylem water potential at the moment of sampling. It works. It is also tedious and destructive. Each leaf can be measured only once. You need a calm day. Wind messes up the readings because transpiration pull changes the internal state faster than the chamber can stabilize. I switched to thermocouple psychrometers for longer-term monitoring. You insert the junction into a leaf, let it equilibrate for twenty minutes, and the instrument calculates water potential from the dew point depression. Slower than a pressure chamber for a quick snapshot, but you can log data every hour without sacrificing tissue. The downside is that psychrometers are sensitive to temperature gradients. If your environmental chamber fluctuates by even half a degree during the equilibration period, your reading drifts. I learned this the hard way when I spent a week troubleshooting a dataset that turned out to be an artifact of a faulty temperature controller. There is also the new generation of micro-scale sensors using capacitive or optical principles. They are smaller, faster, and less destructive, but they cost more and require calibration against a known standard. If you skip calibration, the absolute values are useless even if the relative trends look reasonable. I have seen papers published with uncalibrated sensor data and the conclusions were wrong by nearly 0.5 megapascals. In plant stress research, that is the difference between mild water deficit and severe drought.
Common Mistakes That Waste Time
The biggest error I see is treating water potential as a fixed property of a tissue. It is not. It changes with time of day, light intensity, humidity, soil moisture, and the plant’s own stomatal regulation. A spinach leaf measured at noon on a dry day might be at minus 1.8 megapascals. The same leaf at predawn after a night of rehydration could be at minus 0.4. If you compare those two values without noting the timing, your interpretation of the plant’s water status is garbage. Another trap is assuming that osmotic potential and water potential are interchangeable. They are not. Osmotic potential is one component. Water potential includes pressure and matric forces too. In xylem, the pressure term dominates and osmotic potential is often negligible. In the apoplast, matric forces can matter more than solute effects, especially in dry soil where water is held tightly by capillary action. People also conflate water potential with water content. They are related but distinct. Two soils can have the same water content but very different water potentials if their texture differs. Sandy soil at ten percent volumetric water content has a water potential around minus 1.5 megapascals. Clay soil at the same water content might be at minus 0.3. Plants respond to water potential, not water content. That is why sandy soils feel wet but plants still wilt, while clay soils hold water that plants cannot access.
Edge Cases Where the Theory Breaks Down
Succulent plants are a problem for standard water potential calculations. Their cells store large volumes of water in vacuoles with dynamic solute concentrations that shift throughout the day. The osmotic potential can change by more than 0.5 megapascals between dawn and dusk simply from photosynthetic sugar accumulation. If you use a single measurement to characterize their water relations, you will miss half the story. Halophytes are another edge case. Plants adapted to salty environments maintain very negative osmotic potentials, sometimes below minus 3.0 megapascals in extreme cases. Standard pressure chambers can handle this, but interpreting the data requires knowing whether the plant is osmotically adjusted or simply suffering from ion toxicity. I worked with a sample of Atriplex that looked water-stressed by all standard metrics, but ion analysis showed sodium buildup in the vacuole. The low water potential was not a drought response. It was a salt accumulation artifact. Correct identification required separating osmotic from electrical conductivity measurements, which most basic labs do not do routinely. Freezing temperatures introduce another complication. Supercooled water in xylem can exist below zero without ice formation, and water potential calculations based on liquid-phase assumptions fail when ice begins to form. I once lost an entire set of winter wheat samples because I left them in a walk-in cooler overnight and the water in the apoplast froze, concentrating solutes in the remaining liquid and shifting the measured potential by nearly two megapascals overnight. The cells survived, but the data was irrecoverable.

Practical Takeaways
If you are starting with this, measure at predawn when the plant is closest to equilibrium with soil water. That gives you a baseline. Then measure at midday to capture the transpiration pull. The difference between those two points tells you the hydraulic gradient driving water through the plant. For most crops, that gradient ranges from 0.5 to 2.0 megapascals depending on species and environmental conditions. Seedlings are more sensitive. Mature trees can sustain larger gradients because of their deeper root systems and greater xylem capacitance. Calibrate your instruments against a standard solution. A 1.0 molal sucrose solution has a known osmotic potential of approximately minus 2.4 megapascals at 20 degrees Celsius. Run it through your psychrometer or pressure probe and check that you get close to that value. If you are off by more than 0.1 megapascals, something in your setup needs attention before you trust any biological readings. Record environmental conditions alongside every measurement. Temperature, relative humidity, soil moisture, light level. Without those covariates, a water potential number is just a number. With them, it becomes data you can actually use to make decisions, whether that is irrigation scheduling, breeding for drought tolerance, or modeling plant responses to climate change.