Understanding How Populations Self-Limit in Real Ecosystems
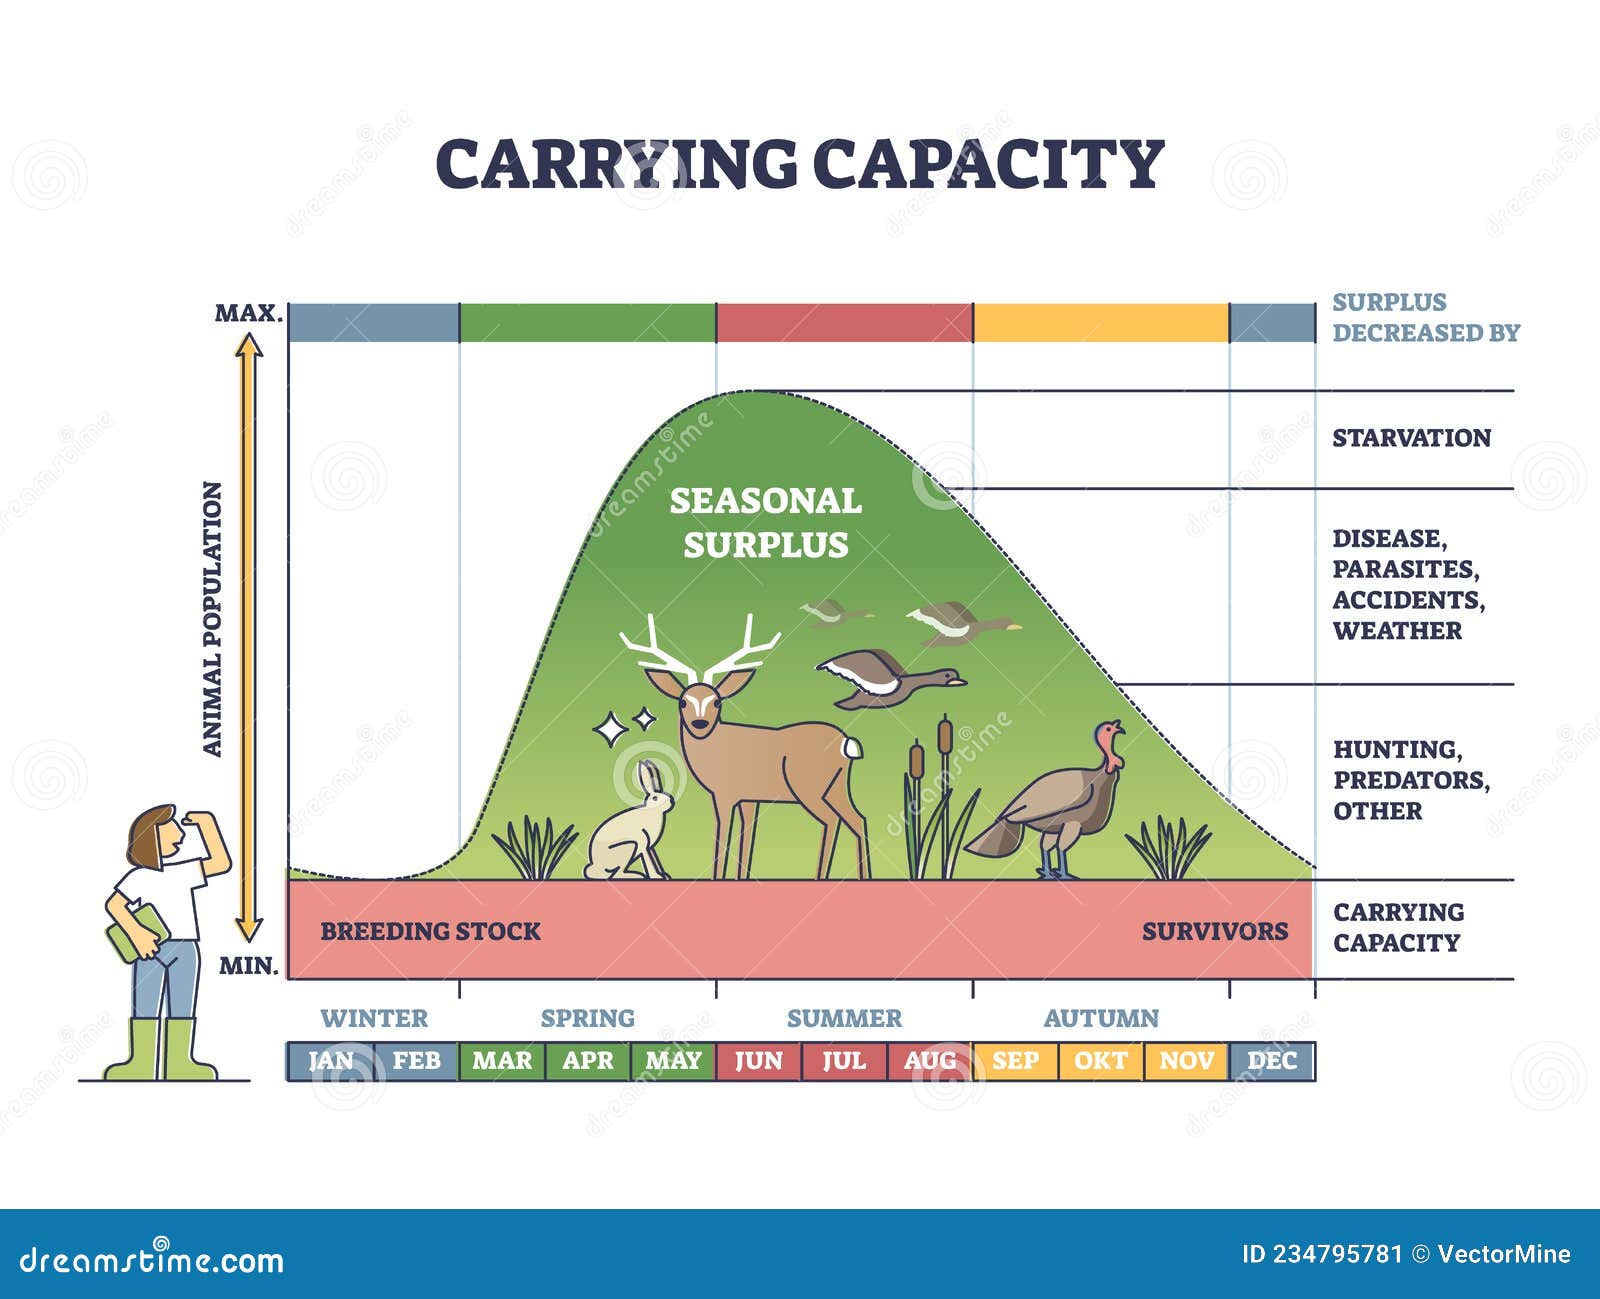
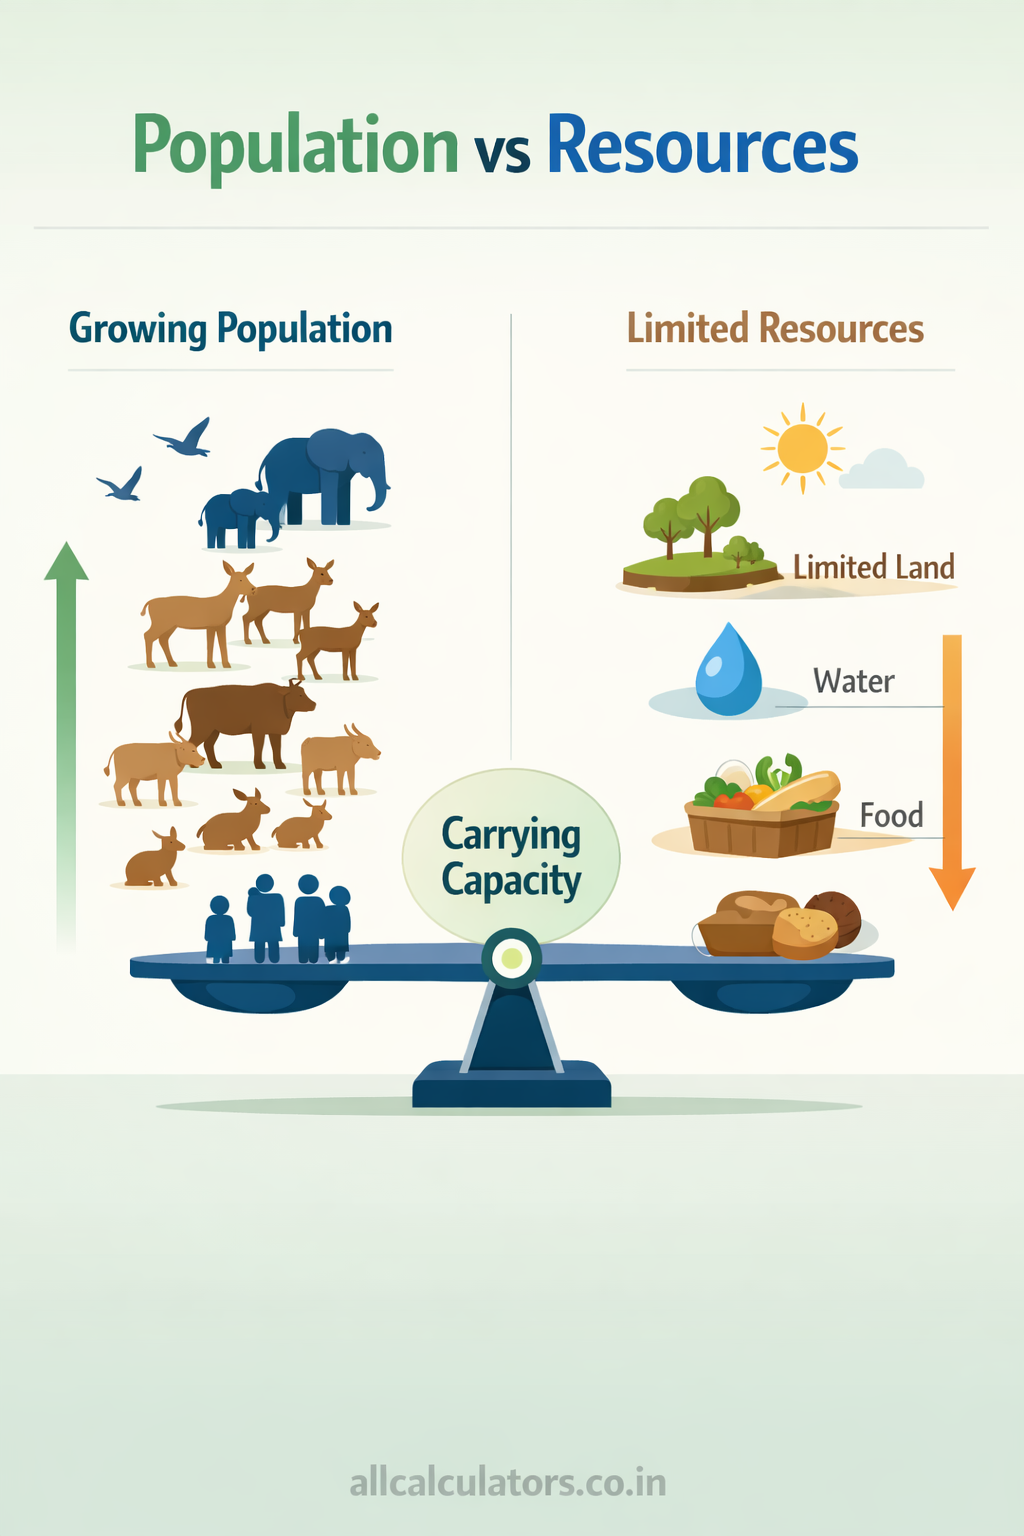
Most people learn carrying capacity as a clean line on a graph, but field ecology rarely works that way. The concept describes the maximum population size an environment can sustain indefinitely without degrading the resources that support it. Once you actually work with it, you quickly realize the number is not fixed. It shifts with seasons, weather events, migration, and sometimes a single introduced species. At its core, carrying capacity is the intersection of available resources and the per-capita demands of a population. Food, water, nesting space, disease pressure, predation — all of those compress together into a single working number that ecologists use for modeling, conservation planning, and wildlife management. You encounter it whenever you are estimating how many deer a parcel of forest can support, how many fish a lake will sustain, or how a species might respond to habitat loss. I spent years running population surveys in temperate forests, and one particular project taught me this concept more than any textbook ever did. We were modeling elk winter ranges in a valley that had been experiencing repeated overpopulation. The initial carrying capacity estimate looked solid on paper, but the herd kept depleting browse faster than our models predicted. We spent three weeks re-evaluating because the data did not match the curves. The problem turned out to be microhabitat variation. The elk were concentrating in riparian zones where winter forage was marginally better, creating localized overbrowsing that dragged the effective carrying capacity down well below the landscape-level average. Once we started measuring use intensity by microhabitat instead of treating the whole valley as one uniform block, our estimates aligned with what we were actually seeing in the field. That was a practical lesson in why carrying capacity is a range, not a point.
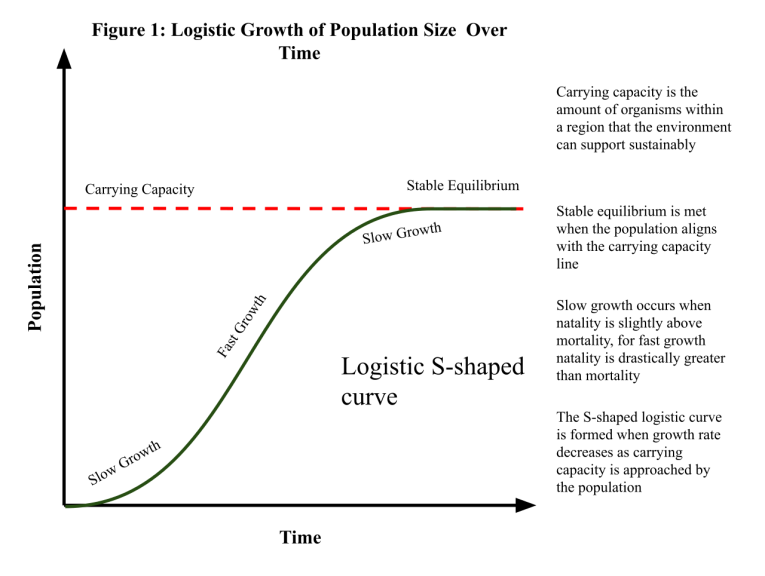
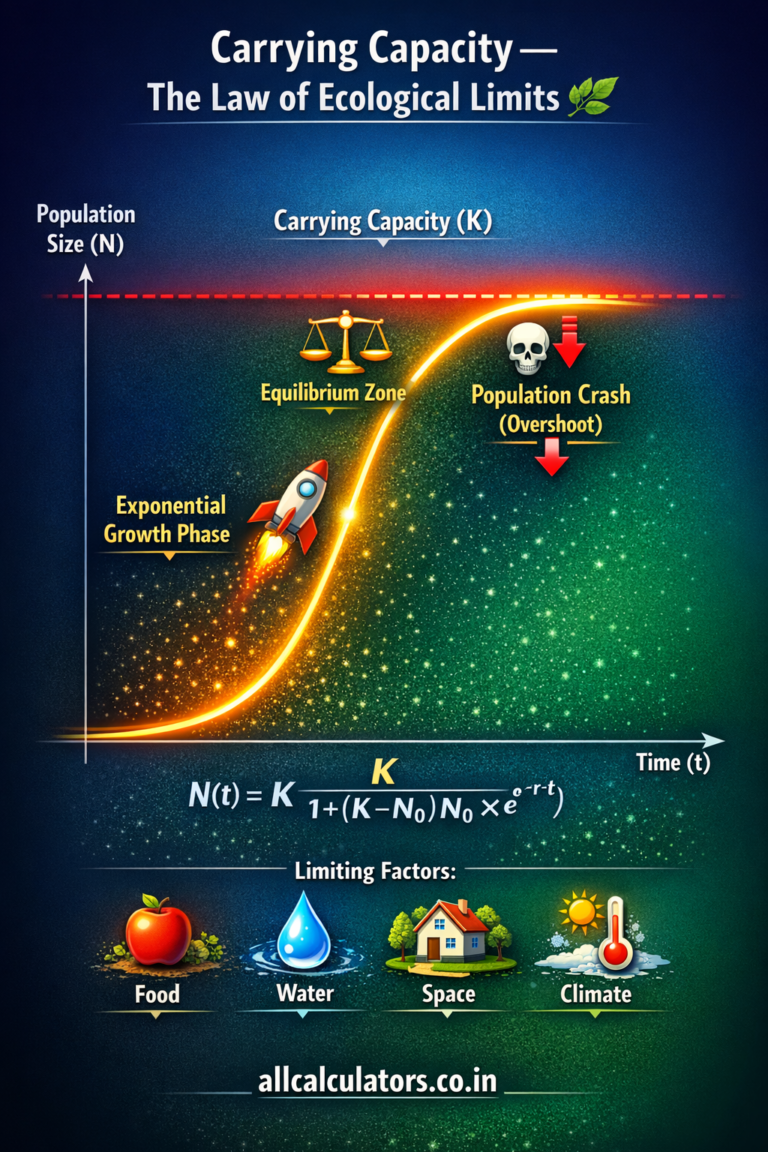
The logistic growth model is still the standard starting point, even though it is blunt. It uses a growth rate that slows as population approaches the carrying capacity limit, usually written with parameters for intrinsic growth rate and current population size. In practice, you rarely know those parameters precisely. You estimate them from mark-recapture data, aerial counts, or harvest records, and each method introduces its own bias. Aerial surveys tend to miss animals in dense cover. Mark-recapture assumes equal catchability, which almost never holds. Harvest data reflects hunter behavior more than animal behavior. So carrying capacity estimates always come with error bars, usually wider than people want to admit. One thing beginners consistently miss is that carrying capacity can be resource-based or space-based, and confusing the two leads to bad management decisions. A population might have plenty of food but no suitable nesting sites, or plenty of open space but toxic water conditions. If you only measure one limiting factor, your carrying capacity estimate will be wrong in whichever direction that missing factor pushes. I once saw a fishery assessment that estimated carrying capacity based on plankton biomass alone. The actual population crashed two years later because the substrate for spawning had been degraded by upstream development. The resource metric looked fine until the reproductive bottleneck showed up. Another counter-intuitive point is that carrying capacity does not guarantee stability. Populations can oscillate around it, overshoot it, or collapse after exceeding it by a wide margin. The classic overshoot-and-collapse pattern shows up frequently in isolated systems like islands, alpine meadows, or enclosed watersheds. A classic example is the Kaibab Plateau deer herd in the 1920s, where predator removal pushed the population well above the actual carrying capacity, followed by mass starvation when forage collapsed. The theoretical carrying capacity had not changed, but the realized carrying capacity dropped dramatically because the ecosystem had been pushed past a threshold.
When you are doing this work, you also have to deal with time lags. Plants do not regrow instantly after being browsed. Soil does not recover immediately after compaction. Predator populations do not respond the same way prey numbers change. These lags mean the environment you are measuring today may not reflect the environment next year. I usually recommend using multi-year datasets whenever possible. A single year of data can mislead you badly if it happens to coincide with a drought, an especially good mast year, or an unusual migration event. Three to five years of consistent data cuts the uncertainty significantly, though it does not eliminate it. If you need a practical workflow, start by defining the population boundary clearly. Then identify the limiting resources for that species across its relevant life stages. Map the spatial distribution of those resources. Collect abundance data across multiple seasons and years if you can. Fit a logistic or Beverton-Holt model, but treat the carrying capacity parameter as a range rather than a point estimate. Validate your model against independent data whenever possible. If validation fails, adjust the resource layers or the spatial assumptions, not just the model parameters. There are tools you can use for this. The free software package R has several packages for population modeling, including thepopbio and momentuHMM packages. For basic logistic curve fitting, standard nonlinear least squares in R works fine and takes only a few lines of code. I prefer using Bayesian frameworks when my data are sparse, because they give you proper uncertainty distributions instead of false precision. The rstan or brms packages handle this well, though they require more setup time upfront. If you want something quicker for simple cases, Excel can fit a logistic curve using the Solver add-in, though you should treat the output as exploratory rather than definitive.
Get the Full Details
One limitation I will state plainly is that carrying capacity models break down in systems with strong trophic cascades or non-equilibrium dynamics. Climate change is making this worse in real time. The baseline environment is shifting faster than most long-term datasets were collected under stable conditions. A carrying capacity estimate derived from twenty years of historical data may be irrelevant if the climate regime has already shifted. I have seen this play out with alpine plant communities where the effective carrying capacity for certain herbivores has changed because snowmelt timing has shifted by weeks, altering the entire growth season. No amount of better modeling fixes that without updating the underlying environmental data. If you need a working alternative when carrying capacity assumptions fail, consider using dynamic energy budget models or individual-based simulations. They are more computationally expensive and require more input data, but they handle changing conditions better than static carrying capacity estimates. For quick assessments under high uncertainty, I also recommend using scenario analysis rather than point estimates. Present three versions: optimistic, baseline, and pessimistic. Decision-makers understand ranges better than false precision. The bottom line is that carrying capacity is a useful concept, but it is not a law. It is an approximation that depends entirely on what you measure, how you measure it, and whether your environment is changing. Treat it like a working hypothesis, validate it against real data, and revise it when the data disagree. The animals do not care about your model equations.